Related Experiment Video
Updated: Aug 10, 2026

T-wave Ion Mobility-mass Spectrometry: Basic Experimental Procedures for Protein Complex Analysis
Published on: August 1, 2010
The association rate constant for heme binding to globin is independent of protein structure
M S Hargrove1, D Barrick, J S Olson
1Department of Biochemistry and Cell Biology, Rice University, Houston, Texas 77251-1892, USA.

Rate constants for CO-heme binding to 35 different recombinant apomyoglobins and several other apoproteins were measured in an effort to understand the factors governing heme affinity and the velocity of the association reaction. Surprisingly, the rate constant for the binding of monomeric heme is approximately 1 x 10(8) M-1 s-1 regardless of the structure or overall affinity of the apoprotein for iron-porphyrin. Major differences between the proteins are reflected primarily in the rates of dissociation of the prosthetic group. Slow phases observed in the reaction of CO heme with excess apomyoglobin result from formation of nonspecific heme-protein complexes which must dissociate before heme can bind specifically in the heme pocket. Once the specific heme-globin complex is formed, the heme pocket rapidly collapses around the porphyrin, simultaneously forming the bond between the proximal His93 and the heme iron atom. The overall affinity of sperm whale apomyoglobin for hemin is approximately 1 x 10(14) M-1. Nonspecific hydrophobic interactions between the porphyrin and the apolar heme cavity account for a factor of 10(5)-10(7). Covalent bond formation between Fe3+ and His93(F8) provides an additional factor of 10(3)-10(4). Specific interactions with conserved amino acids in the heme pocket contribute the final factor of 10(3)-10(4).
Rate constants for CO-heme binding to 35 different recombinant apomyoglobins and several other apoproteins were measured in an effort to understand the factors governing heme affinity and the velocity of the association reaction. Surprisingly, the rate constant for the binding of monomeric heme is approximately 1 x 10(8) M-1 s-1 regardless of the structure or overall affinity of the apoprotein for iron-porphyrin. Major differences between the proteins are reflected primarily in the rates of dissociation of the prosthetic group. Slow phases observed in the reaction of CO heme with excess apomyoglobin result from formation of nonspecific heme-protein complexes which must dissociate before heme can bind specifically in the heme pocket. Once the specific heme-globin complex is formed, the heme pocket rapidly collapses around the porphyrin, simultaneously forming the bond between the proximal His93 and the heme iron atom. The overall affinity of sperm whale apomyoglobin for hemin is approximately 1 x 10(14) M-1. Nonspecific hydrophobic interactions between the porphyrin and the apolar heme cavity account for a factor of 10(5)-10(7). Covalent bond formation between Fe3+ and His93(F8) provides an additional factor of 10(3)-10(4). Specific interactions with conserved amino acids in the heme pocket contribute the final factor of 10(3)-10(4).
Related Concept Videos
 02:15
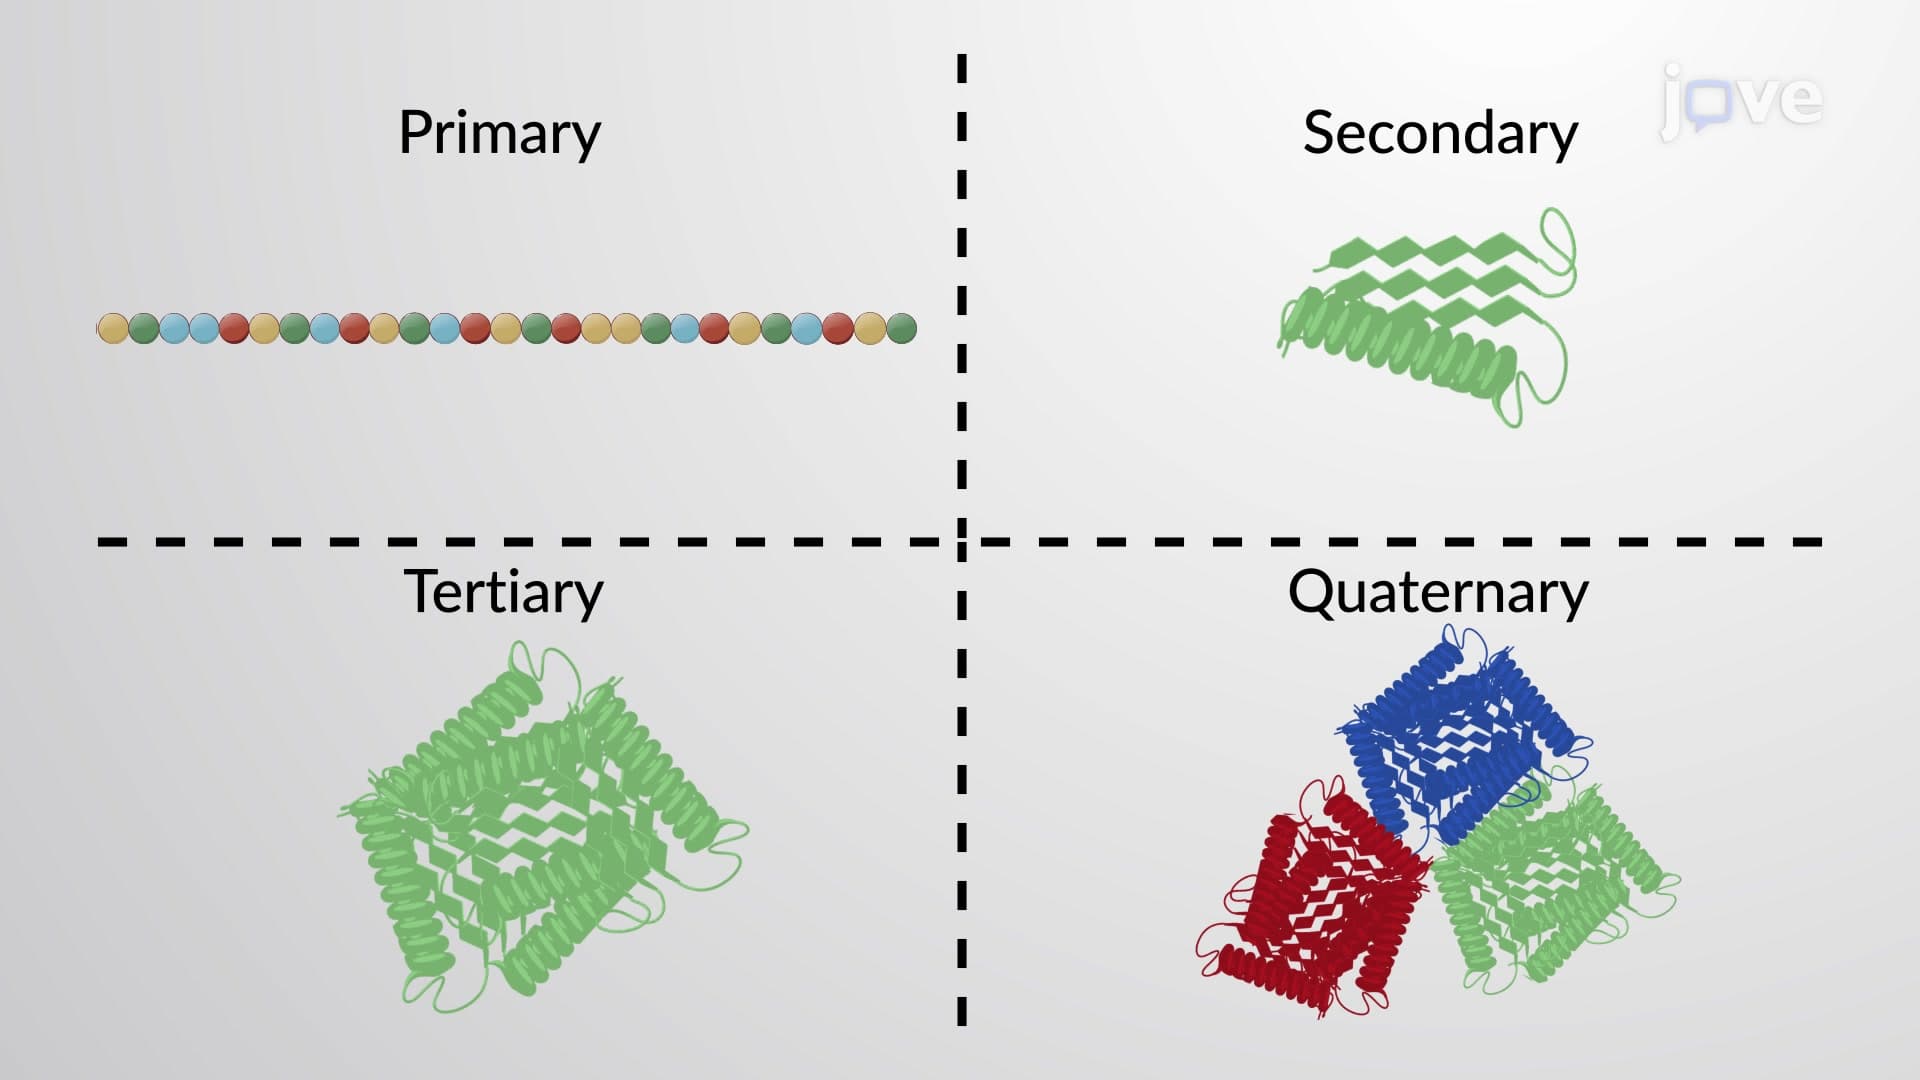
Protein and Protein Structure
A protein's shape is critical to its function. For example, an enzyme can...
 02:18
The Equilibrium Binding Constant and Binding Strength
 01:58
Cooperative Allosteric Transitions
02:18The Equilibrium Binding Constant and Binding Strength
01:58Cooperative Allosteric Transitions
 01:27
Globular Proteins
Globular proteins serve many important physiological functions, such as acting as enzymes, cellular messengers, and molecular transporters. These roles often require the proteins to be soluble in the aqueous...