Related Experiment Video
Updated: Oct 2, 2026

Use of Single Chain MHC Technology to Investigate Co-agonism in Human CD8+ T Cell Activation
Published on: February 28, 2019
A continuous central motif of invariant chain peptides, CLIP, is essential for binding to various I-A MHC class II
S M Weenink1, P J Milburn, A M Gautam
1Human Genetics Group, John Curtin School of Medical Research, The Australian National University, Canberra.

Invariant chain (li) associates with MHC class II molecules and performs a number of crucial functions in antigen presentation. A nested set of class II-associated li peptides (CLIP) has been isolated, comprising the li sequence between residues 82 and 107. Recently, X-ray crystallographic analysis has revealed that residues 87-101 occupy the HLA-DR3 peptide-binding groove. Based on our previous results, Lee and McConnell have also proposed a model for the binding of CLIP to various mouse I-A molecules in the binding groove. CLIP sequences are able to bind many MHC class II molecules but the molecular basis of this promiscuity has not yet been resolved. We have shown recently that CLIP binding to I-A class II molecules is generally tolerant to side chain substitutions, suggesting that the backbone structure of CLIP may provide the features critical for its interaction with class II. In pursuit of this, backbone stereochemical disruptions by serial D-alanine substitutions in CLIP86-104 have been used in competitive binding assays to I-A class II molecules. These studies have revealed that the phylogenetically conserved central continuous region, CLIP91-99, is intolerant to such configurational substitutions. Experiments with truncated and frame-shift analogues of CLIP showed that for effective binding to class II, the sequence element CLIP90-100 must be incorporated into a peptide of 13 or more residues including at least three residues N-terminal to this motif. Additionally, it appears that different I-A molecules accommodate CLIP in different binding frames. These investigations of the relationship between the structure and binding of CLIP analogues lead us to propose that there is a general backbone motif of a periodic nature within the CLIP sequence that minimizes deleterious contacts and allows promiscuous binding to class II molecules.
Invariant chain (li) associates with MHC class II molecules and performs a number of crucial functions in antigen presentation. A nested set of class II-associated li peptides (CLIP) has been isolated, comprising the li sequence between residues 82 and 107. Recently, X-ray crystallographic analysis has revealed that residues 87-101 occupy the HLA-DR3 peptide-binding groove. Based on our previous results, Lee and McConnell have also proposed a model for the binding of CLIP to various mouse I-A molecules in the binding groove. CLIP sequences are able to bind many MHC class II molecules but the molecular basis of this promiscuity has not yet been resolved. We have shown recently that CLIP binding to I-A class II molecules is generally tolerant to side chain substitutions, suggesting that the backbone structure of CLIP may provide the features critical for its interaction with class II. In pursuit of this, backbone stereochemical disruptions by serial D-alanine substitutions in CLIP86-104 have been used in competitive binding assays to I-A class II molecules. These studies have revealed that the phylogenetically conserved central continuous region, CLIP91-99, is intolerant to such configurational substitutions. Experiments with truncated and frame-shift analogues of CLIP showed that for effective binding to class II, the sequence element CLIP90-100 must be incorporated into a peptide of 13 or more residues including at least three residues N-terminal to this motif. Additionally, it appears that different I-A molecules accommodate CLIP in different binding frames. These investigations of the relationship between the structure and binding of CLIP analogues lead us to propose that there is a general backbone motif of a periodic nature within the CLIP sequence that minimizes deleterious contacts and allows promiscuous binding to class II molecules.
More Related Videos
Related Concept Videos
 01:19
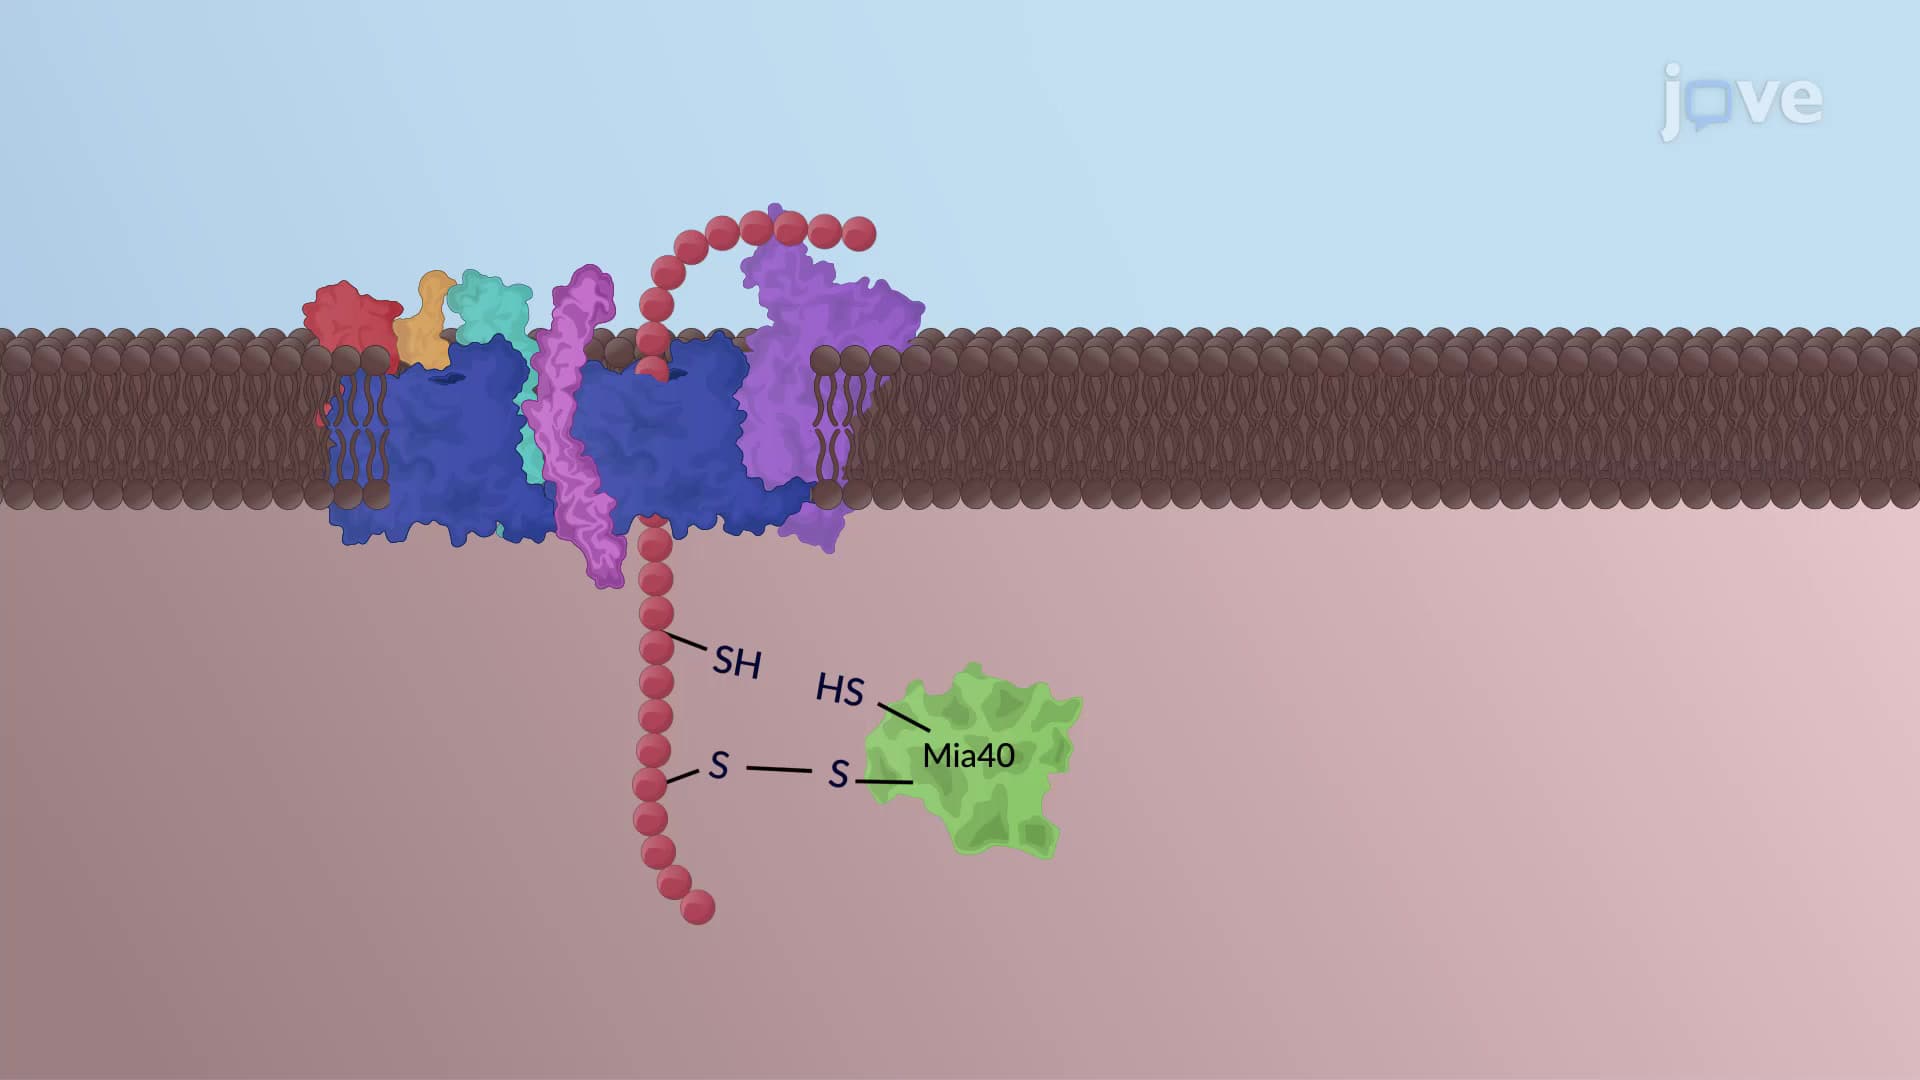
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:10
Integrins
Some ECM proteins assemble into a basement membrane to which the remaining components adhere. Proteoglycans typically form the bulk of the ECM while fibrous proteins, like collagen,...
 01:17
Intracellular Signaling Affects Focal Adhesions
Some...
 01:31
Immunoglobulin-like Cell Adhesion Molecules
Ig-CAMs exhibit either homophilic binding (to other Ig-CAMs) or heterophilic binding (to other ligands such as integrins). While most Ig-CAMs...
 01:26
Antigens Involved in Adaptive Immunity
Complete Antigens
Complete antigens possess both immunogenicity and reactivity.
 01:31
Antigen Processing Pathways
MHC Class I: Presenting Endogenous...