Related Experiment Video
Updated: Oct 21, 2026
Amplification, Next-generation Sequencing, and Genomic DNA Mapping of Retroviral Integration Sites
Published on: March 22, 2016
Implication of a central cysteine residue and the HHCC domain of Moloney murine leukemia virus integrase protein in
G A Donzella1, O Leon, M J Roth
1Department of Biochemistry, University of Medicine and Dentistry of New Jersey-Robert Wood Johnson Medical School, Piscataway 08854, USA.

Abstract:
Moloney murine leukemia virus (M-MuLV) IN-IN protein interactions important for catalysis of strand transfer and unimolecular and bimolecular disintegration reactions were investigated by using a panel of chemically modified M-MuLV IN proteins. Functional complementation of an HHCC-deleted protein (Ndelta105) by an independent HHCC domain (Cdelta232) was severely compromised by NEM modification of either subunit. Productive Ndelta105 IN-DNA interactions with a disintegration substrate lacking a long terminal repeat 5'-single-stranded tail also required complementation by a functional HHCC domain. Virus encoding the C209A M-MuLV IN mutation exhibited delayed virion production and replication kinetics.
Related Concept Videos
 02:41
Protein Complex Assembly
Many viruses self-assemble into a fully functional unit using the infected host cell to...
 02:04
Protein-protein Interfaces
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:29
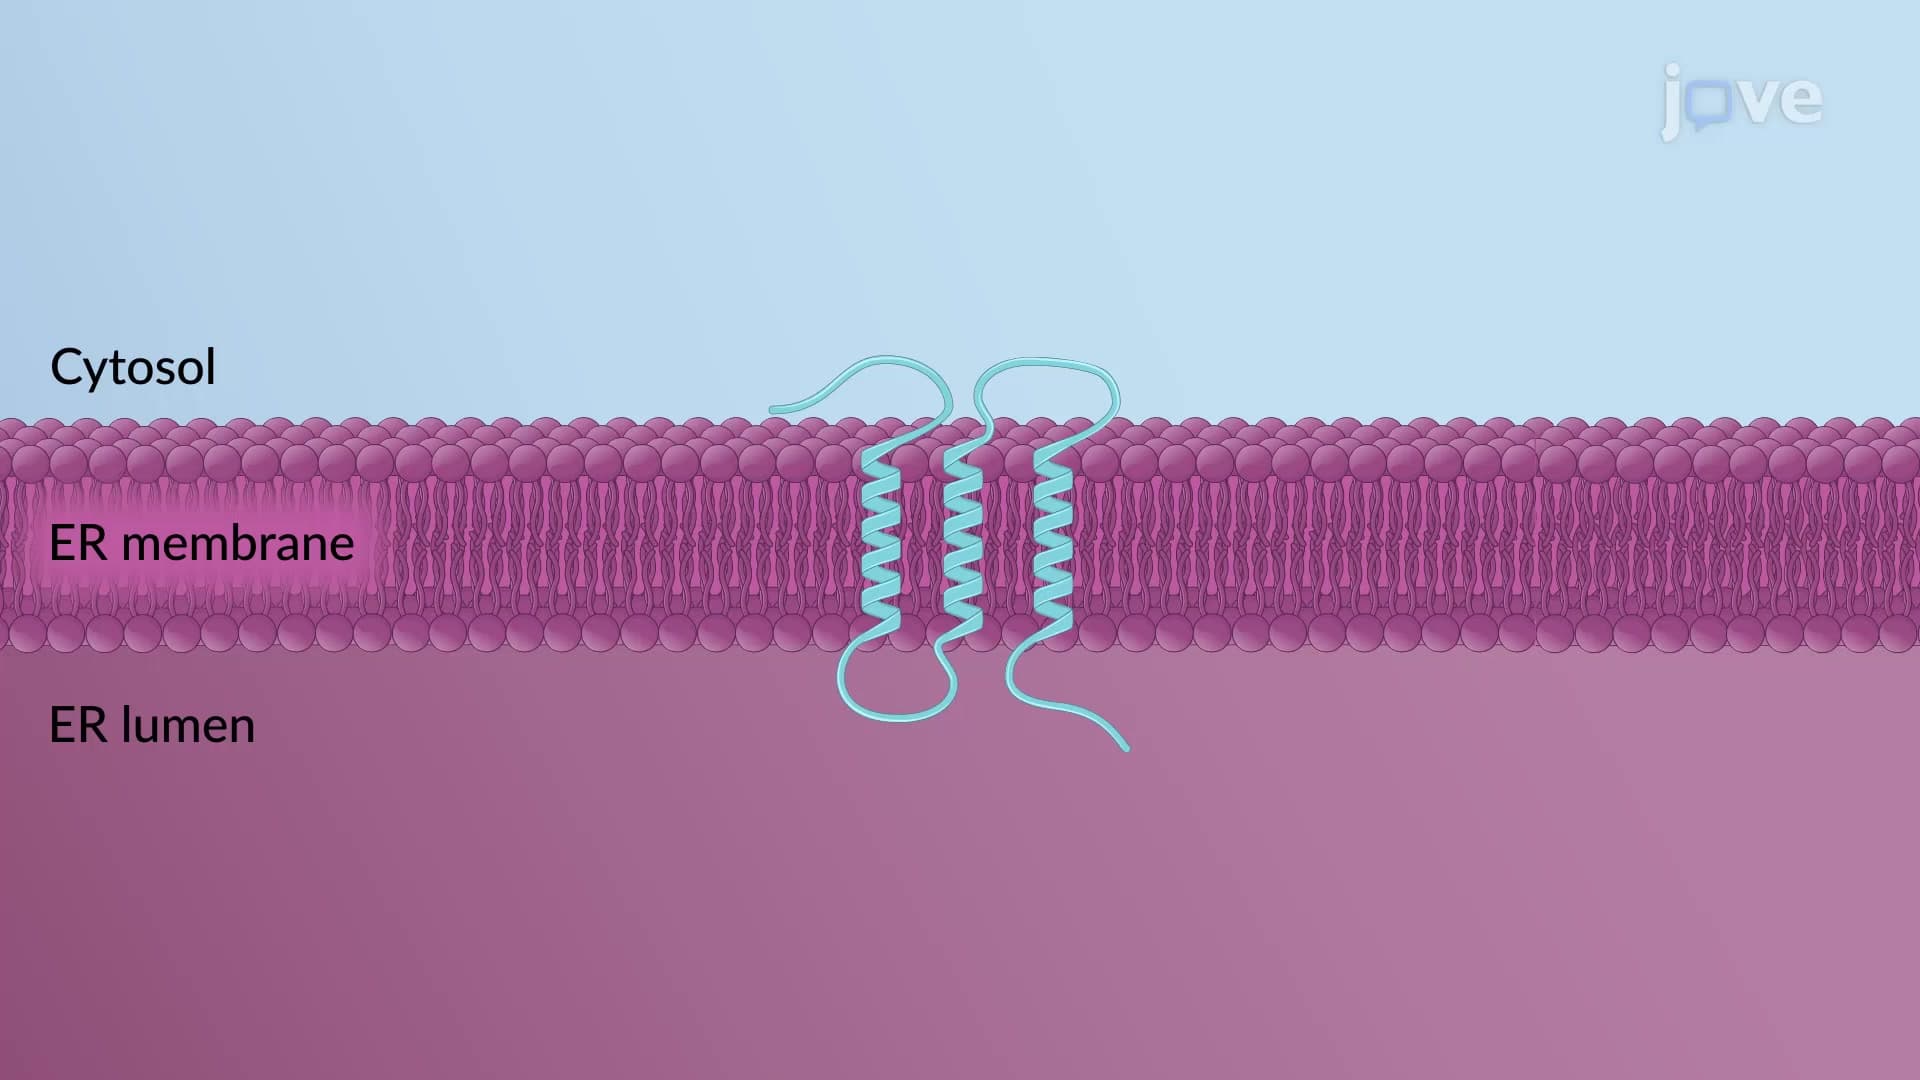
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:09
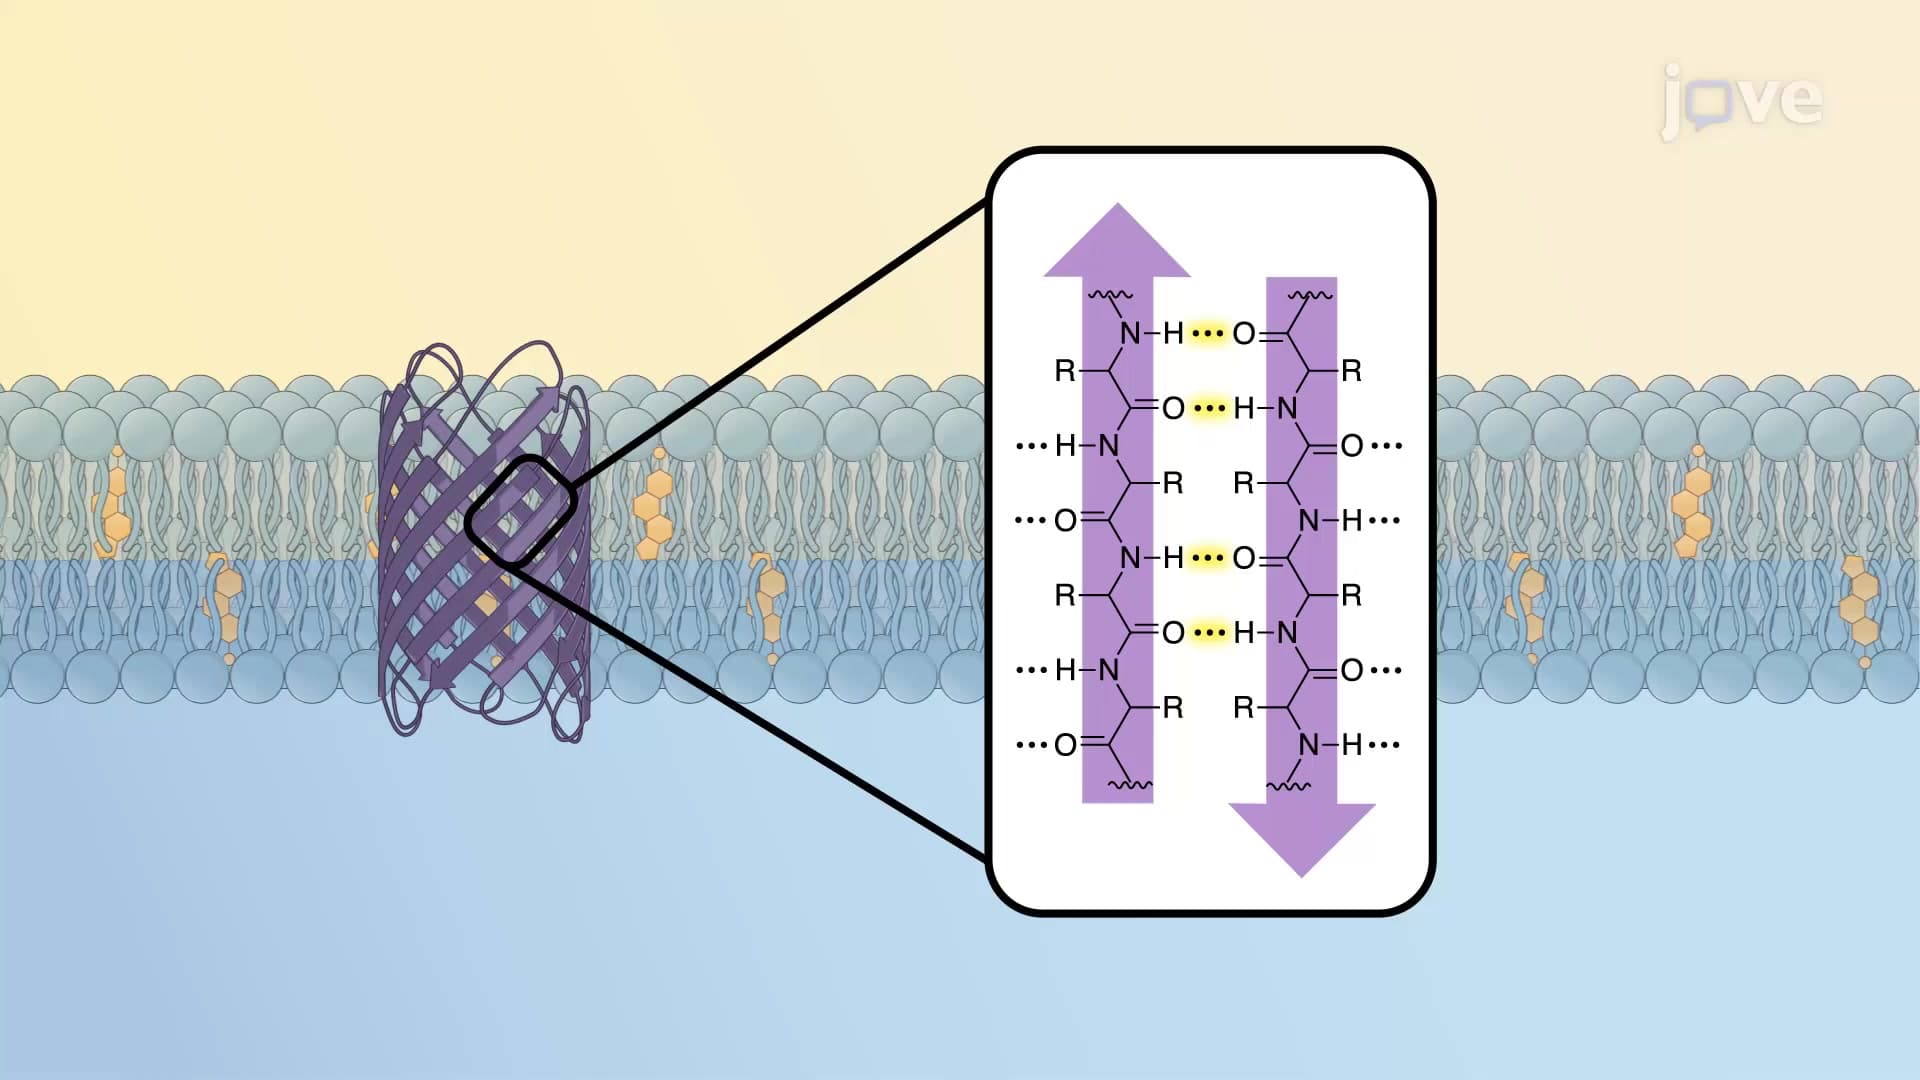
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...