Related Experiment Video
Updated: Jul 11, 2026
PIP-on-a-chip: A Label-free Study of Protein-phosphoinositide Interactions
Published on: July 27, 2017
Another factor besides hydrophobicity can affect signal peptide interaction with signal recognition particle
1Institute of Marine Resources, University of California, Davis, California 95616, USA.

Abstract:
Translocation of alkaline extracellular protease (AEP) into the endoplasmic reticulum of Yarrowia lipolytica is cotranslational and signal recognition particle (SRP)-dependent, whereas translocation of P17M AEP (proline to methionine at position 17, second amino acid in the pro-region) is posttranslational and SRP-independent. P17M signal peptide mutations that resulted in more rapid SRP-dependent translocation of AEP precursor were isolated. Most of these mutations significantly increased hydrophobicity, but the A12P/P17M mutation did not. The switch from SRP-dependent to SRP-independent translocation without a decrease in hydrophobicity (wild type to P17M) and restoration of SRP-dependent translocation without an increase in hydrophobicity (P17M to A12P/P17M) indicate that some factor(s) in addition to hydrophobicity determines selection of targeting pathway. Models of extended forms of wild type and A12P/P17M signal peptides are kinked, whereas the P17M signal peptide is relatively straight. Possibly the conformation/orientation of signal peptides at the ribosomal surface affects SRP binding and consequently the targeting route to the endoplasmic reticulum. Kinked signal peptides might approach SRP more closely more often. Most likely, these effects were only detectable because of the short length and low average hydrophobicity of the AEP signal peptide.
Insights
Yarrowia lipolytica alkaline extracellular protease (AEP) translocation to the endoplasmic reticulum depends on signal peptide properties beyond hydrophobicity. Signal peptide conformation influences the targeting pathway, affecting protein secretion efficiency.
Area of Science:
- Molecular Biology
- Protein Trafficking
- Yeast Genetics
Background:
- Protein translocation into the endoplasmic reticulum (ER) is crucial for secreted proteins in organisms like Yarrowia lipolytica.
- The alkaline extracellular protease (AEP) in Y. lipolytica is translocated into the ER via a signal recognition particle (SRP)-dependent, cotranslational pathway.
- A specific mutation, P17M, alters AEP translocation to an SRP-independent, posttranslational pathway.
Purpose of the Study:
- To investigate the factors governing the switch between SRP-dependent and SRP-independent protein translocation pathways.
- To identify mutations in the AEP signal peptide that alter its translocation mechanism.
- To understand the role of signal peptide hydrophobicity and conformation in protein targeting to the ER.
Main Methods:
- Site-directed mutagenesis was used to create mutations in the AEP signal peptide, including P17M and others.
- Analysis of AEP precursor translocation kinetics and dependence on the signal recognition particle (SRP).
- Computational modeling to assess the conformation and hydrophobicity of wild-type and mutant signal peptides.
Main Results:
- Mutations were identified that restored SRP-dependent translocation of the P17M mutant AEP precursor.
- Some mutations increased signal peptide hydrophobicity, but the A12P/P17M mutation restored SRP dependence without increasing hydrophobicity.
- Signal peptide models suggest that 'kinked' conformations (wild-type, A12P/P17M) may favor SRP binding more than a 'straight' conformation (P17M).
Conclusions:
- Signal peptide conformation, in addition to hydrophobicity, plays a critical role in determining the SRP-dependent or SRP-independent translocation pathway.
- The findings suggest that the orientation of the signal peptide at the ribosomal surface influences SRP interaction and subsequent ER targeting.
- These observations are particularly relevant for short, low-hydrophobicity signal peptides like that of AEP.
Related Concept Videos
 01:32
Lipids as Anchors
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains the...
 01:41
Signal Sequences and Sorting Receptors
 01:45
Regulation of Nuclear Protein Sorting
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
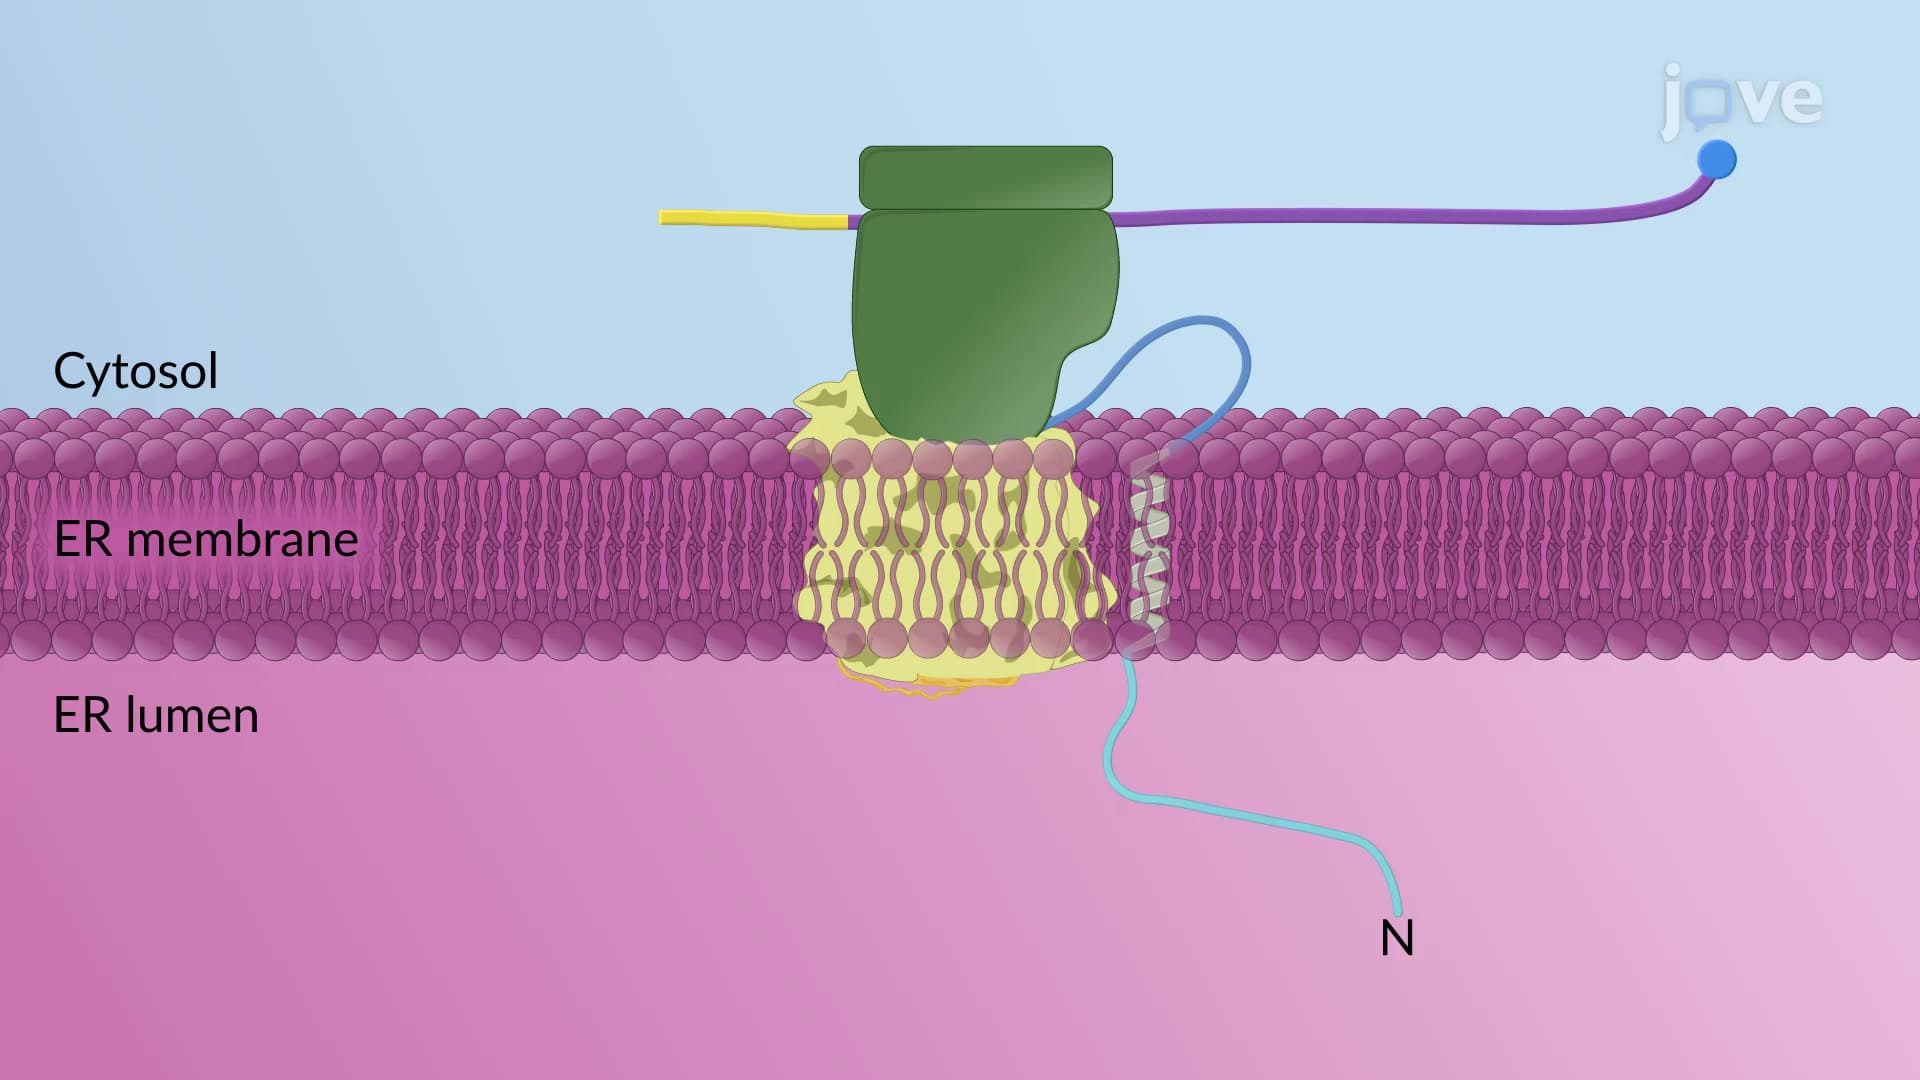
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:45
Tail-anchoring of Proteins in the ER Membrane