Related Experiment Video
Updated: Aug 8, 2026
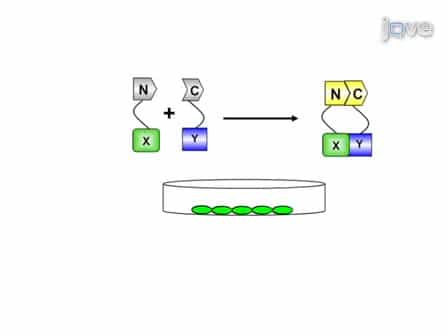

Bimolecular Fluorescence Complementation
Published on: April 15, 2011
I2B is a small cytosolic protein that participates in vacuole fusion
P Slusarewicz1, Z Xu, K Seefeld
1Department of Biochemistry, Dartmouth Medical School, Hanover, NH 03755-3844, USA.

Insights
Two low molecular weight activities, LMA1 and LMA2, are essential for Saccharomyces cerevisiae vacuole inheritance. LMA2 is monomeric protease B inhibitor 2 (I2B), with a novel function in vacuole fusion distinct from its inhibitory role.
Area of Science:
- Cell Biology
- Molecular Biology
- Yeast Genetics
Background:
- Vacuole inheritance in Saccharomyces cerevisiae is a complex process.
- Two low molecular weight activities, LMA1 and LMA2, have been identified as crucial for this process.
- LMA1 is known to be a heterodimer of thioredoxin and protease B inhibitor 2 (I2B).
Purpose of the Study:
- To elucidate the molecular identity and function of LMA2.
- To determine the role of protease B inhibitor 2 (I2B) in vacuole fusion.
- To differentiate the functions of LMA1 and LMA2 in vacuole inheritance.
Main Methods:
- Biochemical characterization of LMA2.
- Analysis of vacuole fusion in yeast strains with varying protease B activity.
- Comparative studies of LMA1 and LMA2 activities in vacuole fusion and protease B inhibition.
Main Results:
- LMA2 was identified as monomeric I2B.
- The protease inhibitor activity of I2B is not directly responsible for promoting vacuole fusion.
- LMA1, the thioredoxin-I2B complex, exhibits significantly higher activity in promoting vacuole fusion compared to monomeric I2B (LMA2).
Conclusions:
- Monomeric I2B (LMA2) plays a distinct role in vacuole fusion, separate from its protease inhibitory function.
- Complex formation of I2B with thioredoxin (LMA1) enhances its role in vacuole fusion.
- These findings establish a new function for I2B in Saccharomyces cerevisiae vacuole inheritance.
Abstract:
Saccharomyces cerevisiae vacuole inheritance requires two low molecular weight activities, LMA1 and LMA2. LMA1 is a heterodimer of thioredoxin and protease B inhibitor 2 (I2B). Here we show that the second low molecular weight activity (LMA2) is monomeric I2B. Though LMA2/I2B was initially identified as a protease B inhibitor, this protease inhibitor activity is not related to its ability to promote vacuole fusion: (i) Low Mr protease B inhibitors cannot substitute for LMA1 or LMA 2, (ii) LMA1 and LMA2 promote the fusion of vacuoles from a strain that has no protease B, (iii) low concentrations of LMA2 that fully inhibit protease B do not promote vacuole fusion, and (iv) LMA1, in which I2B is complexed with thioredoxin, is far more active than LMA2/I2B in promoting vacuole fusion and far less active in inhibiting protease B. These studies establish a new function for I2B.
More Related Videos
Related Concept Videos
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...
 01:30
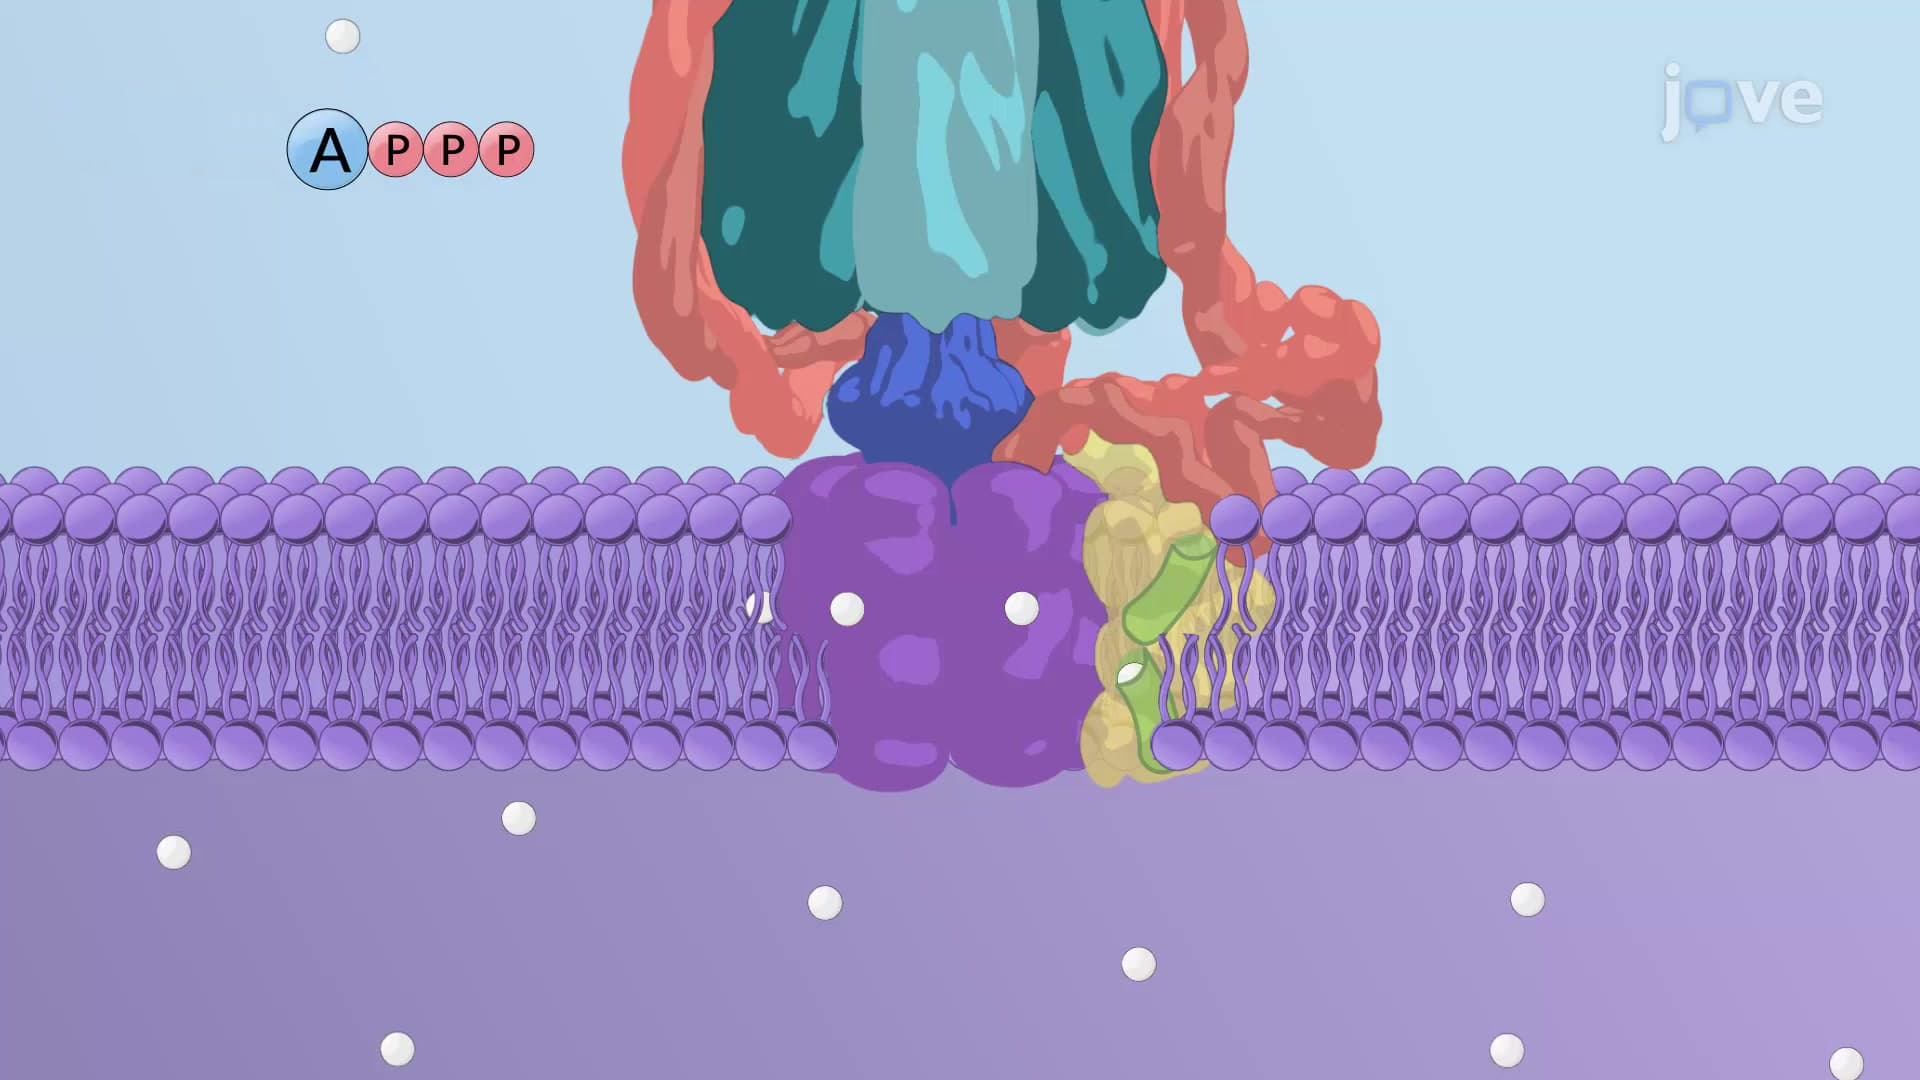
ATP Driven Pumps III: V-type Pumps
The peripheral or cytosolic V1 domain with eight subunits is involved in ATP hydrolysis. The integral or transmembrane V0 domain containing at least five subunits...