Video Experimental Relacionado
Updated: Jul 14, 2026
20:28
A Toolkit to Enable Hydrocarbon Conversion in Aqueous Environments
Published on: October 2, 2012
La activación dependiente de Sir2 de la acetil-CoA sintetasa por desacetilación de la lisina activa
V J Starai1, I Celic, R N Cole
1Department of Bacteriology, University of Wisconsin, Madison, WI 53706-1567, USA.
Science (New York, N.Y.)
|December 21, 2002

Resumen
La acetilación regula la actividad de la enzima acetil-CoA sintetasa (Acs) en Salmonella mediante la modificación de la lisina-609. Esta modificación postraslacional es revertida por la proteína CobB Sir2, revelando un mecanismo regulador común.
Área de la Ciencia:
- La bioquímica es la bioquímica.
- Biología Molecular Biología Molecular
- Enzimología Enzimología.
Sus antecedentes:
- La acetil-coenzima A (CoA) sintetasa (Acs) es una enzima metabólica crucial tanto en procariotas como en eucariotas.
- Acs sintetiza el acetil CoA a partir del acetato, el trifosfato de adenosina (ATP) y el CoA, con la participación de un intermediario monofosfato de acetil-adenosina (AMP).
Objetivo del estudio:
- Para investigar la regulación post-traducional de la actividad de la enzima Salmonella enterica Acs.
- Identificar el mecanismo específico y los factores regulatorios involucrados en la modulación de Acs.
Principales métodos:
- Se emplearon inmunoblotación y espectrometría de masas para analizar la actividad de la enzima Acs.
- Investigó el papel de la acetilación y la proteína CobB Sir2 en la regulación de Acs.
Principales resultados:
- La actividad de la enzima Salmonella enterica Acs está regulada por la acetilación posttranslacional en la lisina-609.
- La acetilación inhibe la síntesis de adenilato intermedio pero no la formación de tioesteros.
- La activación de los Acs acetilados requiere la actividad de la desacetilasa de la proteína CobB Sir2.
Conclusiones:
- La acetilación de lisina es un mecanismo regulador común tanto en procariotas como en eucariotas.
- Los hallazgos sugieren que la acetilación modula las enzimas formadoras de AMP, incluidas las sintetasas de péptidos no ribosómicos y las sintetasas de acil-CoA.
- Amplía la comprensión de las funciones de la proteína Sir2 en el silenciamiento de genes, la estabilidad cromosómica y el envejecimiento.
Más Videos Relacionados
Videos de Conceptos Relacionados
 01:15
Pyruvate Oxidation
After glycolysis, the charged pyruvate molecules enter the mitochondria via active transport and undergo three enzymatic reactions. These reactions ensure that pyruvate can enter the next metabolic pathway so that energy stored in the pyruvate molecules can be harnessed by the cells.
First, the enzyme pyruvate dehydrogenase removes the carboxyl group from pyruvate and releases it as carbon dioxide. The stripped molecule is then oxidized and releases electrons, which are then picked up by NAD+...
First, the enzyme pyruvate dehydrogenase removes the carboxyl group from pyruvate and releases it as carbon dioxide. The stripped molecule is then oxidized and releases electrons, which are then picked up by NAD+...
 01:26
Protein Modifications in the RER
Modification of secretory and transmembrane proteins entering the rough ER begins in the ER lumen. These modifications aid in protein folding and stabilize the acquired tertiary structure. Protein modifications in the rough ER co-occur at different stages of protein folding.
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal sequences.
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal sequences.
 01:07
Catalytically Perfect Enzymes
The theory of catalytically perfect enzymes was first proposed by W.J. Albery and J. R. Knowles in 1976. These enzymes catalyze biochemical reactions at high-speed. Their catalytic efficiency values range from 108-109 M-1s-1. These enzymes are also called 'diffusion-controlled' as the only rate-limiting step in the catalysis is that of the substrate diffusion into the active site. Examples include triose phosphate isomerase, fumarase, and superoxide dismutase.
 01:19
Allosteric Proteins-ATCase
Binding sites linkages can regulate a protein's function. For example, enzyme activity is often regulated through a feedback mechanism where the end product of the biochemical process serves as an inhibitor.
Aspartate transcarbamoylase (ATCase) is a cytosolic enzyme that catalyzes the condensation of L-aspartate and carbamoyl phosphate to N-carbamoyl-L-aspartate. This reaction is the first step in pyrimidine biosynthesis. UTP and CTP, the end products of the pyrimidine synthesis pathway,...
Aspartate transcarbamoylase (ATCase) is a cytosolic enzyme that catalyzes the condensation of L-aspartate and carbamoyl phosphate to N-carbamoyl-L-aspartate. This reaction is the first step in pyrimidine biosynthesis. UTP and CTP, the end products of the pyrimidine synthesis pathway,...
 01:18
Amino Acid Catabolism
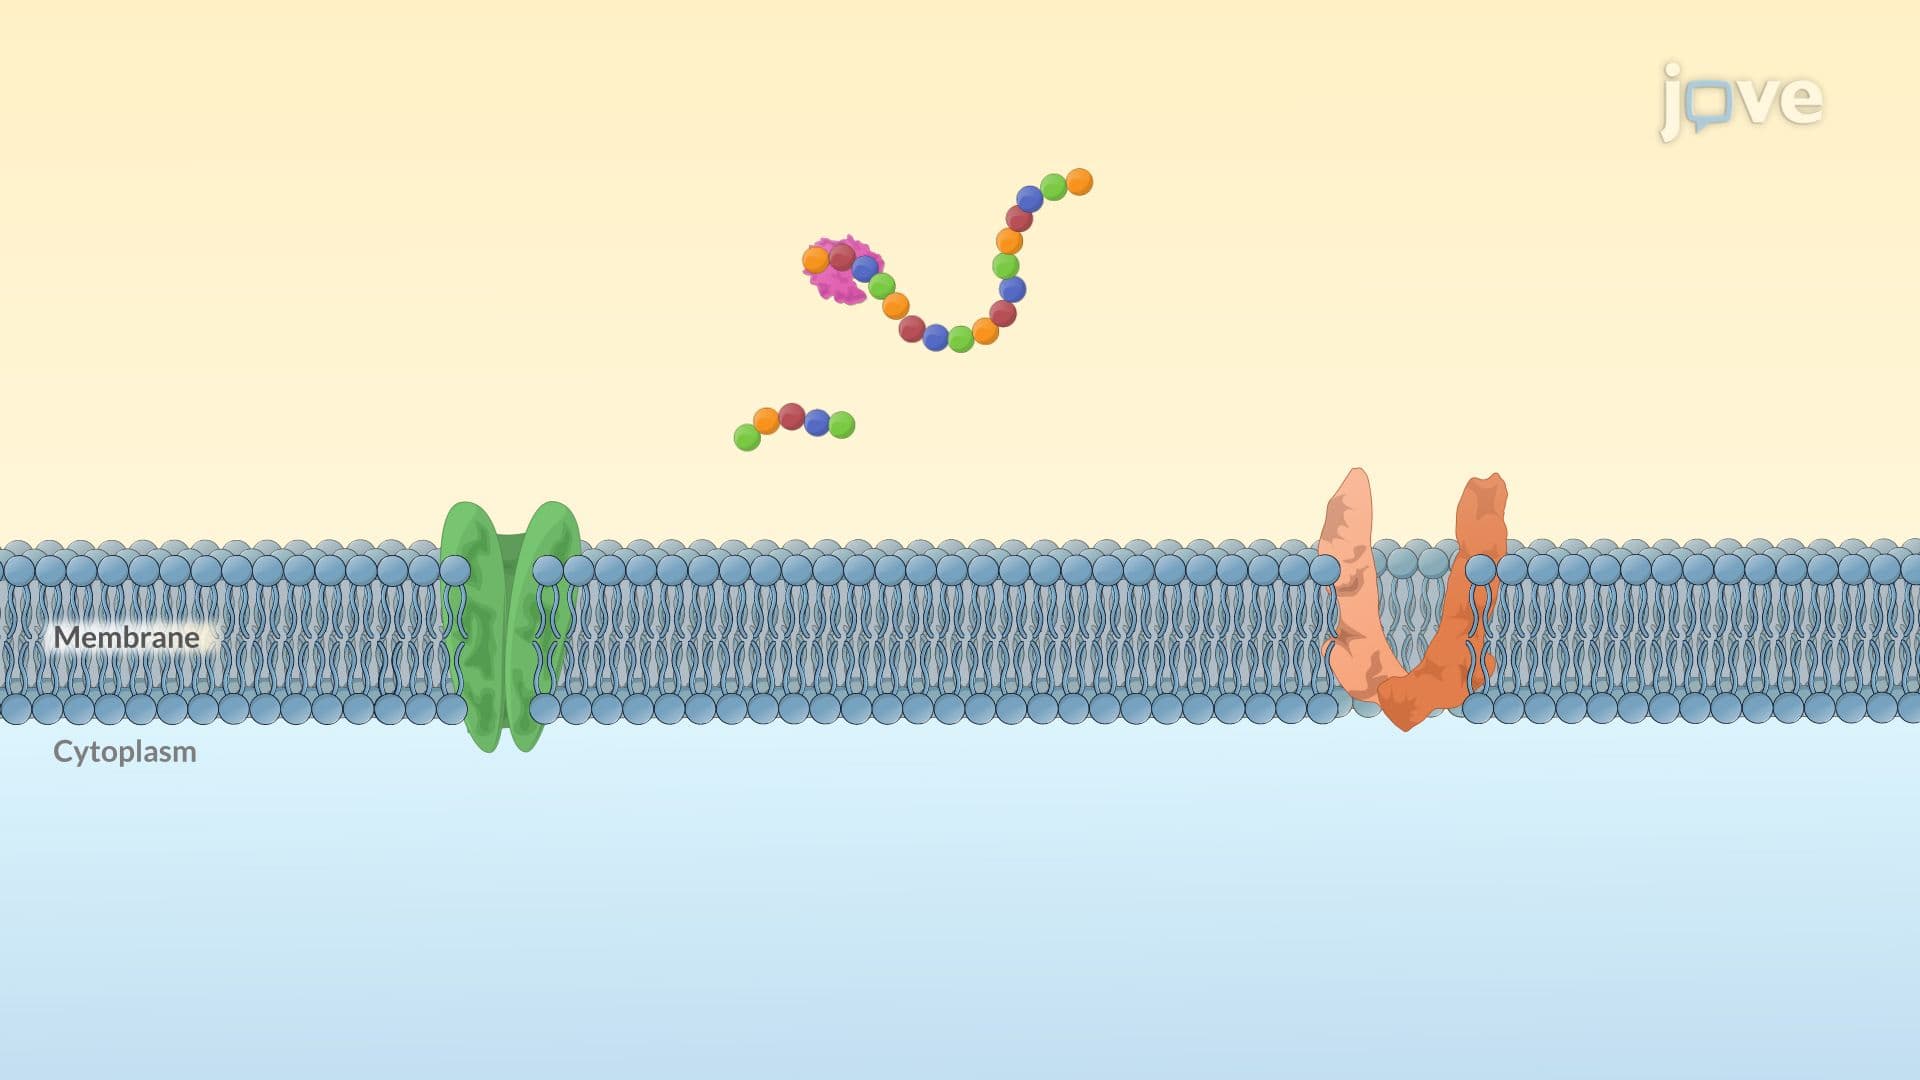
Microorganisms rely on proteins as an essential carbon and energy source, particularly in environments with limited polysaccharides or lipids. However, proteins are too large to cross the plasma membrane unaided, necessitating enzymatic degradation. Microbes secrete extracellular proteases and peptidases that hydrolyze proteins into peptides, which can then be transported across the membrane. Once inside the cell, intracellular proteases degrade these peptides into free amino acids, which...
 01:20
Sulfur Assimilation
Sulfur is an essential element in biological systems, contributing to synthesizing key biomolecules, including amino acids such as cysteine and methionine, and cofactors such as coenzyme A and biotin. Microorganisms primarily assimilate sulfur as sulfate (SO₄²⁻) from the environment, which must undergo a series of biochemical transformations before it can be incorporated into cellular components. As sulfate is highly oxidized, it must undergo assimilatory sulfate reduction to become...