Video Experimental Relacionado
Updated: Jul 17, 2026

The Logic, Experimental Steps, and Potential of Heterologous Natural Product Biosynthesis Featuring the Complex Antibiotic Erythromycin A Produced Through E. coli
Published on: January 13, 2013
Estructura de Ero1p, fuente de enlaces disulfuro para el plegamiento oxidativo de proteínas en la célula
Einav Gross1, David B Kastner, Chris A Kaiser
1Department of Structural Biology, Weizmann Institute of Science, Rehovot 76100, Israel.

La flavoenzima Ero1p genera enlaces disulfuro para el plegamiento de las proteínas. Su estructura cristalina revela un mecanismo catalítico similar al de Erv2p, lo que sugiere una estrategia de transferencia de electrones conservados en las flavoenzimas generadoras de disulfuro.
Área de la Ciencia:
- La bioquímica es la bioquímica.
- Biología Estructural Biología estructural.
- Biología Molecular Biología Molecular
Sus antecedentes:
- La flavoenzima Ero1p es crucial para el plegamiento de proteínas oxidativas en el retículo endoplasmático.
- Genera enlaces disulfuro a través de reacciones de intercambio diotiol-disulfuro con la proteína disulfuro isomerasa y las proteínas del sustrato.
- El mecanismo preciso de la oxidación del tiol catalizado por Ero1p permanece en gran parte sin aclarar.
Objetivo del estudio:
- Para dilucidar el mecanismo molecular de la oxidación del tiol catalizado por Ero1p.
- Para determinar la estructura cristalográfica de rayos X de Ero1p.
- Comprender el papel del motivo CXXCXXC y la disposición espacial de las cisteínas del sitio activo y el cofactor.
Principales métodos:
- Cristalografía de rayos X con rayos X.
- Análisis estructural de Ero1p.
- Análisis comparativo con Erv2pp.
Principales resultados:
- La estructura cristalina de Ero1p revela características moleculares detalladas de su centro catalítico.
- Se identificó un motivo CXXCXXC conservado y la relación espacial entre las cisteinas clave y el cofactor unido.
- El sitio activo de Ero1p comparte una notable similitud estructural con el módulo de tiol oxidasa de Erv2p, a pesar de carecer de homología de secuencia.
- Tanto Ero1p como Erv2p utilizan motivos esenciales de dicisteína ubicados en segmentos de polipéptidos móviles.
Conclusiones:
- Los datos estructurales proporcionan información sobre el mecanismo de oxidación del tiol catalizado por Ero1p.
- Se propone un mecanismo de transferencia de electrones conservado que involucra motivos móviles de dicisteína y un sitio activo rígido para las flavoenzimas generadoras de disulfuro como Ero1p y Erv2p.
Videos de Conceptos Relacionados
 01:43
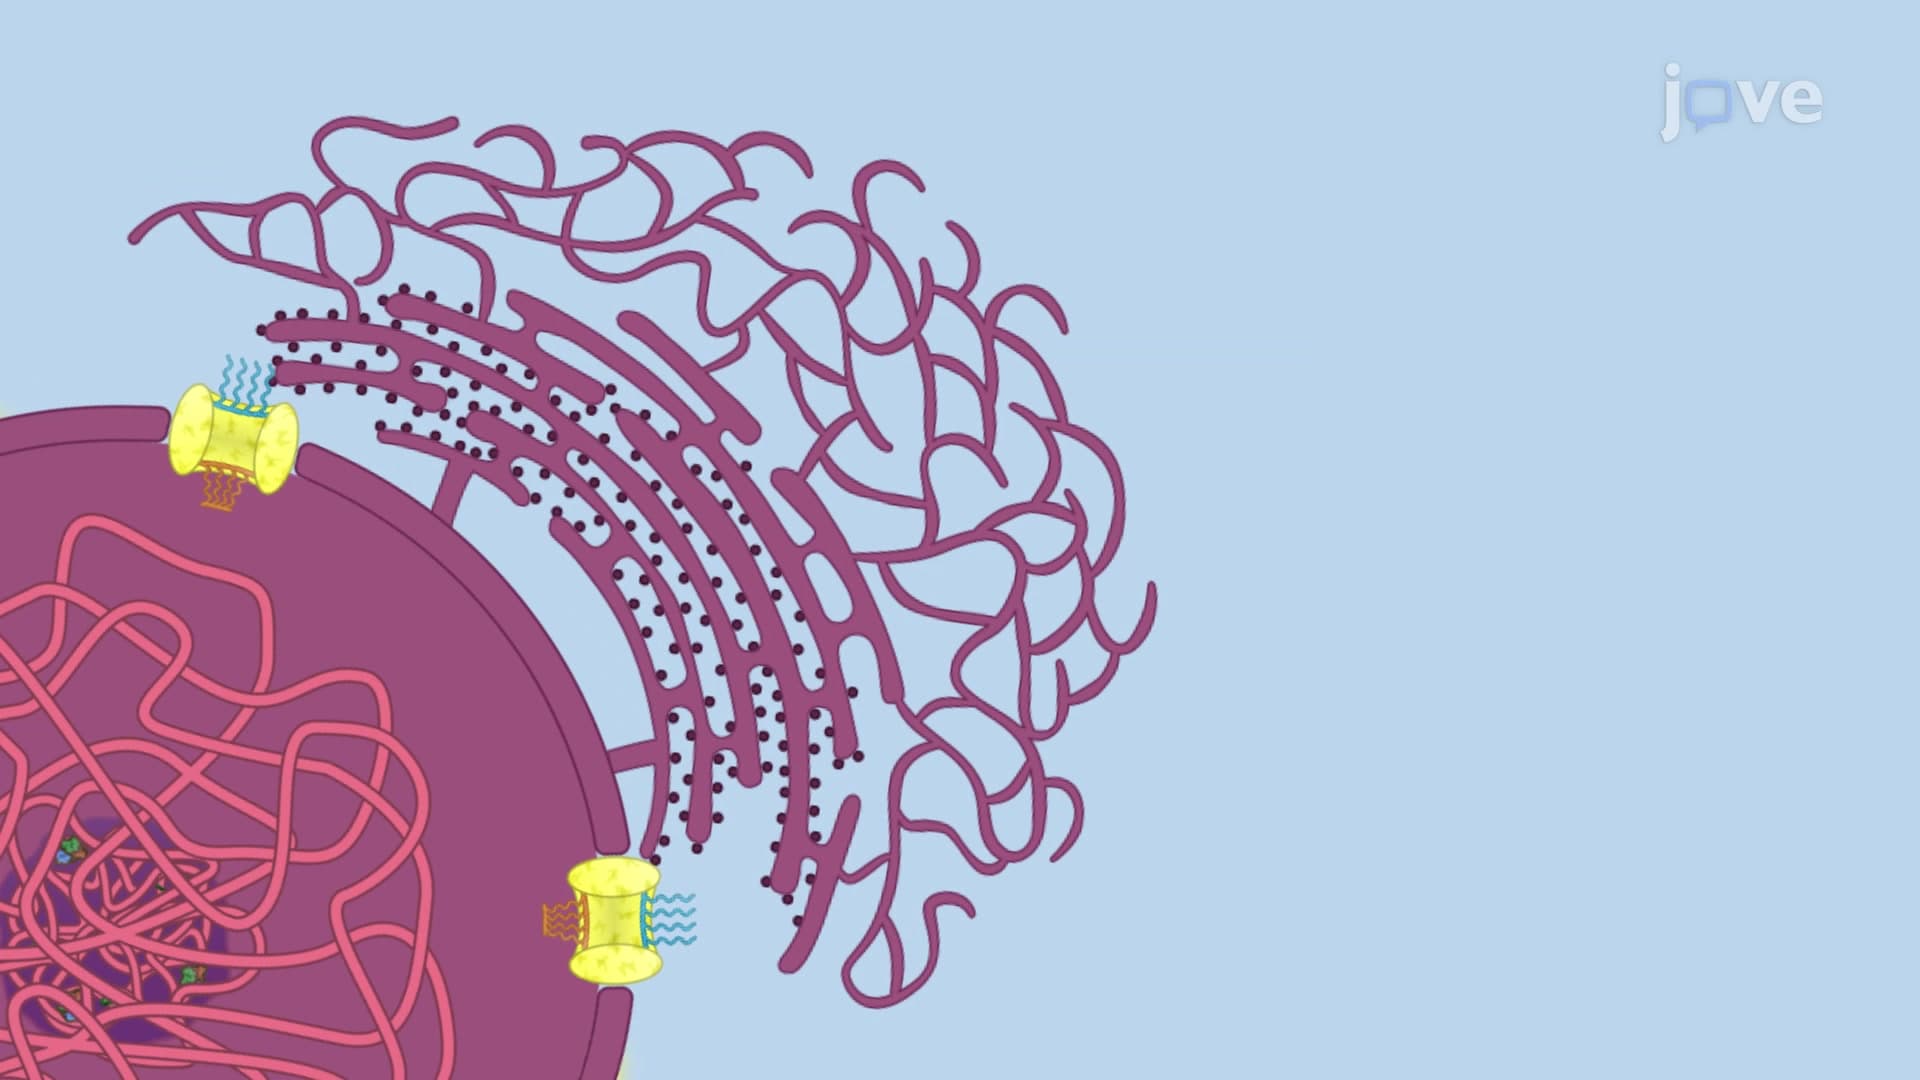
The Endoplasmic Reticulum
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 01:26
Protein Modifications in the RER
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal sequences.
 01:31
Regulation of the Unfolded Protein Response
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
01:43The Endoplasmic Reticulum