関連する実験動画
Updated: Apr 29, 2026
08:57
Aip1p Dynamics Are Altered by the R256H Mutation in Actin
Published on: July 30, 2014
7.8K
ARF1-ARFGAP複合体の構造的・機能的分析により,GTPの水解におけるコアトメアの役割が明らかになった
1Cellular Biochemistry and Biophysics Program, Memorial Sloan-Kettering Cancer Center, New York, New York 10021, USA. jonathan@ximpact4.ski.mskcc.org
Cell
|April 2, 1999

まとめ
ARF1 GTPase-activating protein (ARFGAP) とコアトーマー複合体の構造は,ARFGAPがGTPの水解をどのように促進するかを明らかにしています. この三重複合体は,COPIの膀層の分解を制御する.
科学分野:
- 分子生物学は分子生物学である.
- 構造生物学 構造生物学とは
- バイオケミストリー バイオケミストリー
背景:
- ADP-リボシライゼーションファクター1 (ARF1) は,小胞体輸送に不可欠な小さなGTPaseである.
- ARFのGTP酶活性化タンパク質 (ARFGAPs) は,GTPの水解を促進することによってARF1の活性を調節する.
- COPIでコーティングされた膀は,ゴルジ装置内の逆行輸送に関与しています.
研究 の 目的:
- ARF1.1のARFGAPによる規制の構造的基礎を明らかにする.
- GTPase反応におけるコアトメアの役割を理解するために.
- COPIベシクルコート分解を制御する三重複合体を特徴付けるために.
主な方法:
- 複雑な構造を決定するために1.95Aの解像度のX線結晶学.
- GTPの水解速度を評価するための生化学分析.
主要な成果:
- 結晶構造は,ARFGAPがARF1のスイッチ2とヘリックスalpha3に結合し,直接的な活性部位参加なしに,残基を触媒に指向することを示している.
- ARF1のエフェクター結合領域は,コンプレックス内でアクセス可能である.
- 生物化学実験では,コアトーマーがARFGAPに依存した方法でGTPの水解を1000倍加速することを示しています.
結論:
- ARF1,ARFGAP,コアトーマーを含む三重複合体は,GTPの水解を調節するために不可欠です.
- この複合体は,COPIの膀層の分解を誘発する.
- この発見は,膀輸送調節の分子メカニズムについての洞察を提供します.
関連する概念動画
 01:14
Generation of Straight or Branched Actin Filaments
2.9K
The straight or branched structure formation of actin filaments is controlled by nucleating proteins such as the formins and Arp2/3 complex. Formin-mediated assembly results in straight filaments, whereas Arp2/3 protein complex-mediated assembly results in branched actin filaments.
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
2.9K
 01:19
Actin Filament Depolymerization
3.0K
Actin filaments (F-actin) are composed of actin subunits. The dissociation of actin monomers can occur from either end of F-actin. The rate of dissociation is faster from the minus-end or the pointed end, where the actin subunits exist with a bound ADP, together known as ADP-actin. The depolymerization of F-actin is aided by proteins, including the actin-depolymerizing factor (ADF) and cofilin family of proteins, gelsolin, and glia maturation factor (GMF).
In F-actin, the ADF/cofilin proteins...
In F-actin, the ADF/cofilin proteins...
3.0K
 01:32
Pinching-off of Coated Vesicles
3.1K
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
3.1K
 01:33
Coat Assembly and GTPases
3.5K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.5K
 01:14
Rab Proteins
4.0K
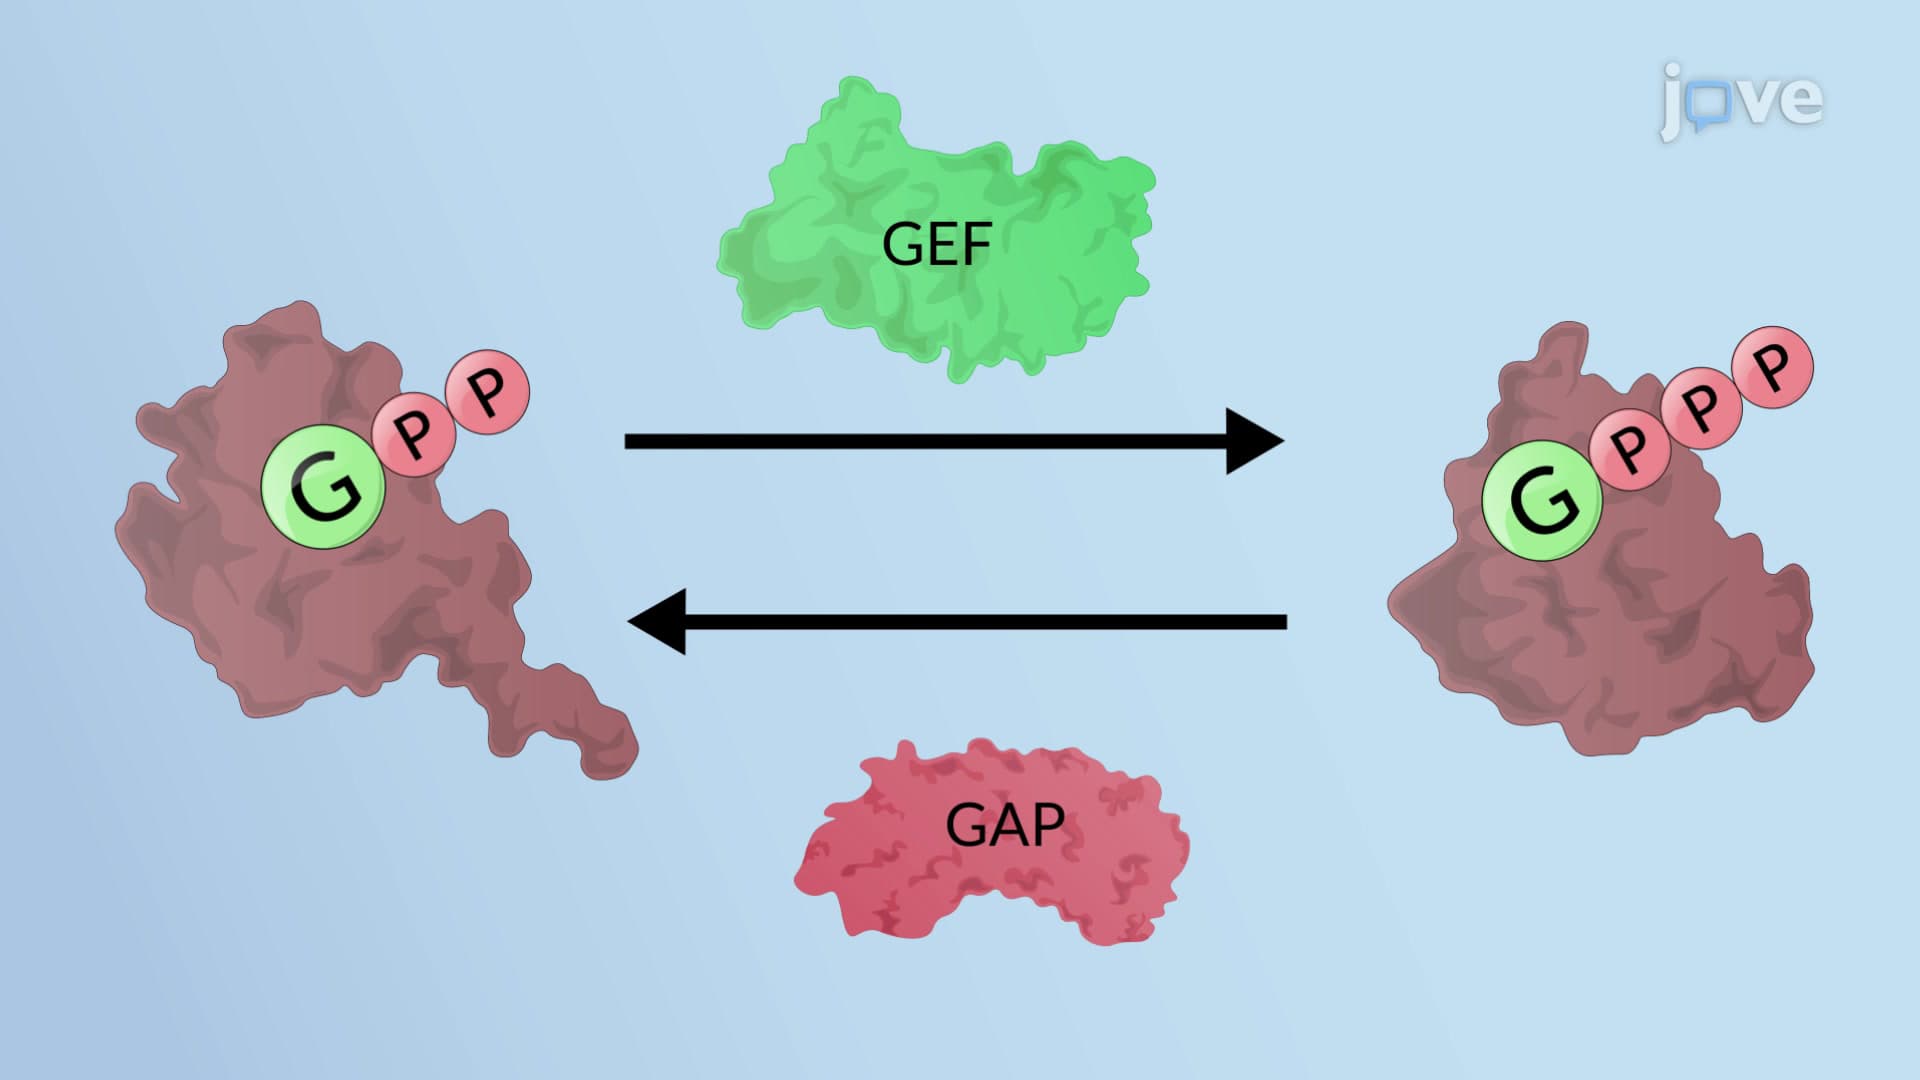
Rab proteins constitute the largest family of monomeric GTPases, of which 70 members are present in humans. Rab proteins and their effectors regulate consecutive stages of vesicle transport such as vesicle transport, docking, and fusion to the correct recipient membrane.
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
4.0K
 01:25
Rab Cascades
2.8K
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
2.8K