
Gcn5ブロモドメインは,核細胞の再編成を調整する
P Syntichaki1, I Topalidou, G Thireos
1Institute of Molecular Biology and Biotechnology, FORTH, and Department of Biology, University of Crete, Heraklion, Greece.
Nature
|April 4, 2000

まとめ
ヒストンアセチルトランスフェラーゼ (HAT) のブロモドメインは,ヒストンアセチル化と核細胞再構成を結びつける. この相互作用は,Swi2依存の転写活性化において極めて重要であり,Swi/Snf複合体を安定させる.
科学分野:
- 分子生物学は分子生物学である.
- エピジェネティクス エピジェネティクス
- 遺伝子規制 遺伝子規制
背景:
- ユカリオットプロモーターへの転写因子のアクセスは,多タンパク質複合体によるクロマチンの構造変化を必要とする.
- ヒストンアセチルトランスフェラーゼ (HAT) とATPアゼ (Swi/SnfにおけるSwi2のように) は,再構成複合体の主要なクラスである.
- プロモーターの規制におけるHATとSwi/Snf複合体の機能的関連性は不明である.
研究 の 目的:
- 保存されたHATモジュールであるブロモドメインが,ヒストンアセチル化と後の核細胞再構成を結びつける役割について調査する.
- ブロモドメイン-アセチル化されたリシン結合がHAT活性および下流イベントのためにin vivoにおいて不可欠であるかどうかを決定する.
主な方法:
- Gcn5ブロモドメインの in vivo 機能的要件を研究するために,特定のプロモーターシステムを利用しました.
- Gcn5媒介ヒストンアセチル化のための in vitro アセチルライシン結合に重要なブロモドメイン残留物の必要性を評価した.
- ブロモドメイン変異がSwi2依存の核細胞リモデリングと転写活性化に与える影響を評価した.
主要な成果:
- in vitro アセチルライシン結合に不可欠なブロモドメイン残基は,Gcn5媒介ヒストンアセチル化 in vivoでは不要である.
- これらの特定のブロモドメイン残基は,その後のSwi2依存の核細胞体改造と転写活性化に不可欠です.
- Gcn5ブロモドメインは,プロモーターのSwi/Snf複合体を安定させることが示されました.
結論:
- ブロモドメインはヒストンアセチル化と核細胞再構成機構の間の重要なリンクとして機能する.
- ブロモドメイン-アセチル-ライシン相互作用は,Swi/Snf複合体の標的と安定化に不可欠であり,転写活性化を促進します.
- この研究は,真核生物の遺伝子発現の調整された調節における重要なメカニズムを解明しています.
関連する概念動画
 02:33
The Nucleosome
DNA in a human cell is almost 2m long and it is packed inside a tiny nucleus that is only a few microns in diameter. The level of compaction of DNA inside the nucleus is astonishing. It is organized into several sequentially higher levels of compaction to fit into such a tiny space. The most compact form of DNA is a chromosome that can be seen under a microscope in a dividing cell.
DNA is wound twice around a protein complex called histone core, that consist of 8 histone proteins. This complex...
DNA is wound twice around a protein complex called histone core, that consist of 8 histone proteins. This complex...
 02:10
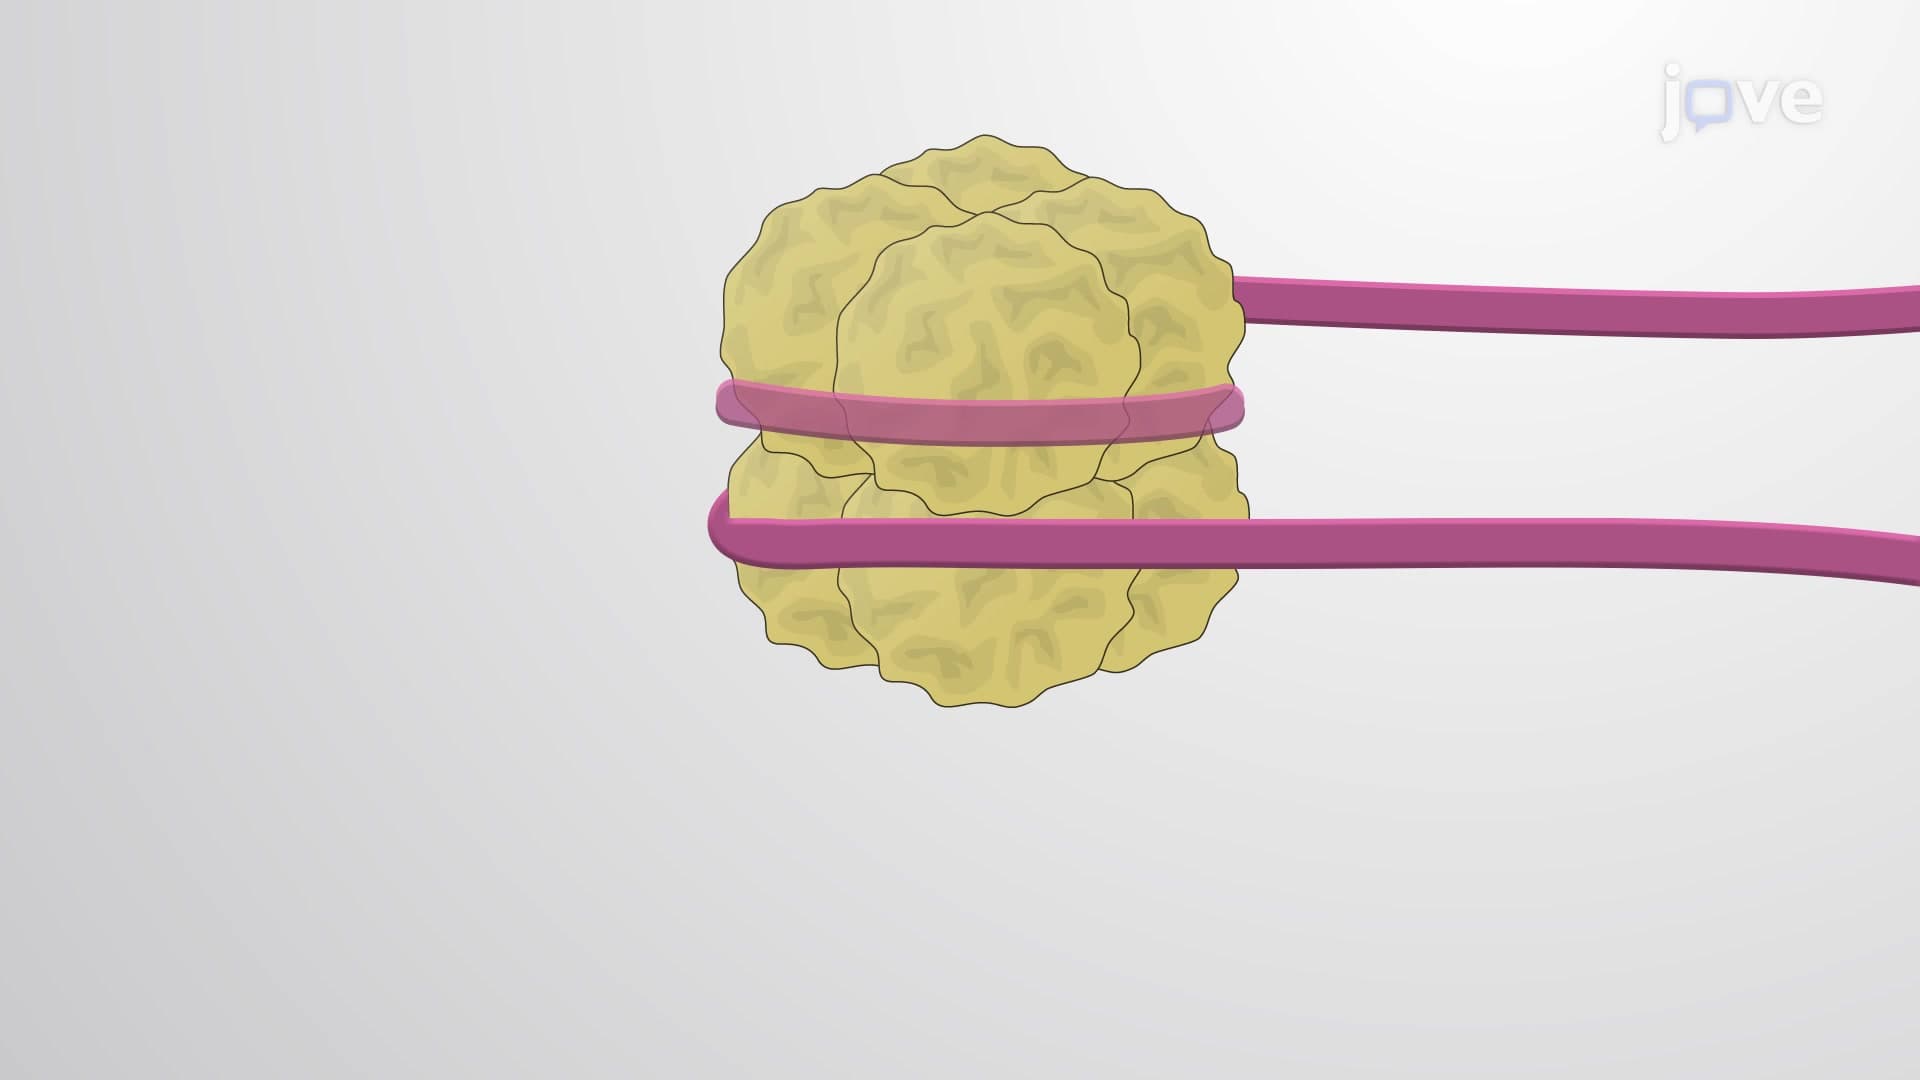
The Nucleosome Core Particle
Nucleosomes are the DNA-histone complex, where the DNA strand is wound around the histone core. The histone core is an octamer containing two copies of H2A, H2B, H3, and H4 histone proteins.
The paradox
Nucleosomes, paradoxically, perform two opposite functions simultaneously. On the one hand, their main responsibility is to protect the delicate DNA strands from physical damage and help achieve a higher compaction ratio. While on the other hand, they must allow polymerase enzymes to access DNA...
The paradox
Nucleosomes, paradoxically, perform two opposite functions simultaneously. On the one hand, their main responsibility is to protect the delicate DNA strands from physical damage and help achieve a higher compaction ratio. While on the other hand, they must allow polymerase enzymes to access DNA...
 02:54
Nucleosome Remodeling
Nucleosomes are the basic units of chromatin compaction. Each nucleosome consists of the DNA bound tightly around a histone core, which makes the DNA inaccessible to DNA binding proteins such as DNA polymerase and RNA polymerase. Hence, the fundamental problem is to ensure access to DNA when appropriate, despite the compact and protective chromatin structure.
Nucleosome remodeling complex
Eukaryotic cells have specialized enzymes called ATP-dependent nucleosome remodeling enzymes. These enzymes...
Nucleosome remodeling complex
Eukaryotic cells have specialized enzymes called ATP-dependent nucleosome remodeling enzymes. These enzymes...
 02:32
Histone Modification
The histone proteins have a flexible N-terminal tail extending out from the nucleosome. These histone tails are often subjected to post-translational modifications such as acetylation, methylation, phosphorylation, and ubiquitination. Particular combinations of these modifications form “histone codes” that influence the chromatin folding and tissue-specific gene expression.
Acetylation
The enzyme histone acetyltransferase adds acetyl group to the histones. Another enzyme, histone deacetylase,...
Acetylation
The enzyme histone acetyltransferase adds acetyl group to the histones. Another enzyme, histone deacetylase,...
02:32Histone Modification
The histone proteins have a flexible N-terminal tail extending out from the nucleosome. These histone tails are often subjected to post-translational modifications such as acetylation, methylation, phosphorylation, and ubiquitination. Particular combinations of these modifications form “histone codes” that influence the chromatin folding and tissue-specific gene expression.
Acetylation
The enzyme histone acetyltransferase adds acetyl group to the histones. Another enzyme, histone deacetylase,...
Acetylation
The enzyme histone acetyltransferase adds acetyl group to the histones. Another enzyme, histone deacetylase,...
 01:12
The Nucleosome Core Particle
Nucleosomes are the DNA-histone complex, where the DNA strand is wound around the histone core. The histone core is an octamer containing two copies of H2A, H2B, H3, and H4 histone proteins.
Nucleosomes, paradoxically, perform two opposite functions simultaneously. On the one hand, their primary aim is to protect the delicate DNA strands from physical damage and help achieve a higher compaction ratio. On the other hand, they must allow polymerase enzymes to access histone-bound DNA during...
Nucleosomes, paradoxically, perform two opposite functions simultaneously. On the one hand, their primary aim is to protect the delicate DNA strands from physical damage and help achieve a higher compaction ratio. On the other hand, they must allow polymerase enzymes to access histone-bound DNA during...