CNF1は,バクテリアの宿主細胞の侵入のためにRho GTPaseの活性化を制限するために,ユビキチン-プロテアソーム機構を利用します
Anne Doye1, Amel Mettouchi, Guillaume Bossis
1INSERM U452, IFR 50, Faculté de Médecine, 28 avenue de Valombrose, 06107, Nice, France.
Cell
|November 20, 2002

まとめ
E. coliからのCNF1毒素は,膀細胞内のRho GTPasesを一時的に活性化させます. この活性化は,Racの分解につながり,細菌の侵入と宿主細胞の運動を可能にします.
科学分野:
- 微生物学 微生物学とは
- 細胞生物学 細胞生物学
- バイオケミストリー バイオケミストリー
背景:
- 尿病原性E. coliからのCNF1毒素は,毒性の要因である.
- CNF1は,重要なグルタミン残基をデアミド化し,構成的活性につながることで,Rho GTPases (RhoA, Rac, Cdc42) を活性化します.
研究 の 目的:
- 膀細胞におけるCNF1によるRho GTPase活性化のダイナミクスを調査する.
- Rho GTPasesの一時的な活性化と,その後の無活性化に根本的なメカニズムを解明する.
主な方法:
- CNF1.1で治療された膀細胞におけるRho GTPase活性化の測定
- Racのユビキティレーションとプロテアソモール分解の分析.
- 宿主細胞の運動性と細菌の侵入の評価.
主要な成果:
- CNF1はRho GTPasesの一時的な活性化を誘導し,特にRac.
- Racの無効化は,ユビキチン/プロテアゾーム媒介の分解に対する感受性の増加と関連していた.
- 活性化されたRacの分解は宿主細胞の運動性と細菌の侵入を促した.
結論:
- CNF1の毒性は,Rho GTPasesの制御された活性化から生じる.
- 宿主細胞のプロテアソマル機構は,GTPaseの活性を調節するためにCNF1によってハイジャックされます.
- このメカニズムは,宿主細胞の機能を操作することによって,細菌の病原化を可能にします.
さらに関連する動画
関連する概念動画
 01:45
Regulation of Nuclear Protein Sorting
2.5K
Nuclear protein sorting regulates nucleus composition and gene expression, crucial for determining the fate of a eukaryotic cell. Hence, the entry and exit of molecules across the nuclear envelope is a tightly controlled process. Nuclear protein sorting can be inhibited by one of the following ways: 1) masking cargo signal sequences, 2) modifying the nuclear receptor's affinity for cargo, 3) controlling the nuclear pore size, 4) retaining the cargo during its transit to the cytosol or the...
2.5K
 01:14
Rab Proteins
4.0K
Rab proteins constitute the largest family of monomeric GTPases, of which 70 members are present in humans. Rab proteins and their effectors regulate consecutive stages of vesicle transport such as vesicle transport, docking, and fusion to the correct recipient membrane.
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
4.0K
 02:26
NF-κB-dependent Signaling Pathway
7.6K
The transcription factor NF-κB was discovered in 1986 in the lab of Nobel laureate Professor David Baltimore, for its interaction with the immunoglobulin light chain enhancer in B-cells. After more than three decades of study, it is now evident that NF-κB regulates the expression of over 100 genes. Most of these genes play an essential role in the innate and adaptive immune responses as well as the inflammatory responses of animals.
NF-κB-dependent Signaling Mechanism
The...
NF-κB-dependent Signaling Mechanism
The...
7.6K
 01:25
Rab Cascades
2.8K
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
2.8K
 01:24
Small GTPases - Ras and Rho
4.4K
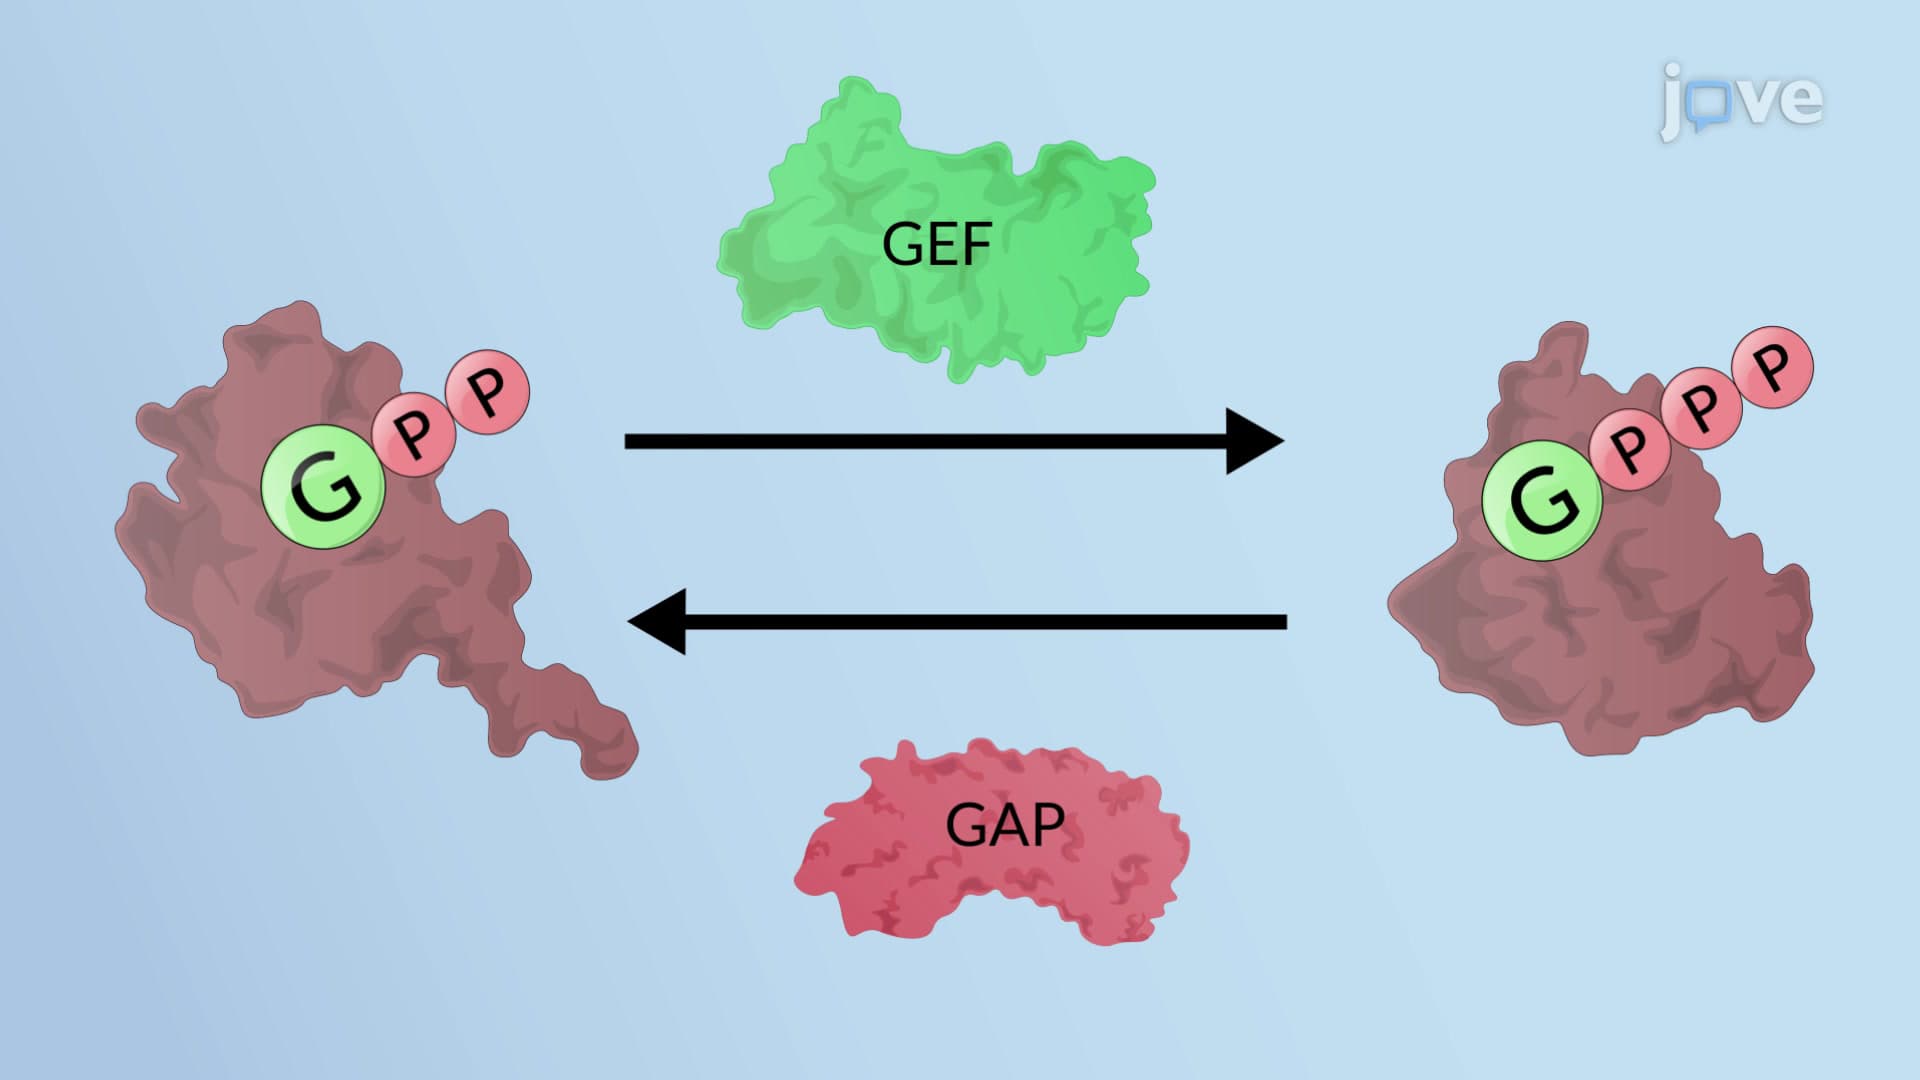
Ras and Rho are small monomeric GTPases that act downstream of receptor tyrosine kinase (RTK) and regulate various cellular processes. These GTPases switch between active and inactive states by binding to guanine nucleotides.
Three regulatory proteins control their activity:
Three regulatory proteins control their activity:
4.4K
 01:09
GPCRs Regulate Adenylyl Cylase Activity
6.9K
Some GPCRs transmit signals through adenylyl cyclase (AC), a transmembrane enzyme. AC helps synthesize second messenger cyclic adenosine monophosphate (cAMP). AC catalyzes cyclization reaction and converts ATP to cAMP by releasing a pyrophosphate. The pyrophosphate is further hydrolyzed to phosphate by the enzyme pyrophosphatase, which drives cAMP synthesis to completion. However, cAMP is rapidly degraded to 5′ AMP by the enzymes phosphodiesterase (PDE), preventing overstimulation of...
6.9K