シナプトタグミンの異なるドメインは,キス&ランと完全融合の選択を制御する
Chih-Tien Wang1, Juu-Chin Lu, Jihong Bai
1Department of Physiology, University of Wisconsin-Madison, Madison, Wisconsin 53706, USA.
Nature
|August 22, 2003

まとめ
シナプトタグミン (Syt) タンパク質は,エクソサイトーシスの経路を調節する. Syt IVはキス・アンド・ランを促し,Syt Iは完全な融合を好み,選択に影響を与える特定のドメインにカルシウムが結合する.
科学分野:
- 神経科学は神経科学である.
- 細胞生物学 細胞生物学
- バイオケミストリー バイオケミストリー
背景:
- 膀の内容を放出するプロセスであるエクソサイトーシスは,完全な融合またはキス&ランメカニズムを通じて発生します.
- これらのエクソサイトーシス経路の間の選択を左右する分子調節は,ほとんど不明のままである.
研究 の 目的:
- 完全融合とキス・アンド・ランエクソサイトーシスの選択を調節するシナプトタグミン (Syt) タンパク質の役割を調査する.
- この規制プロセスにおけるSytドメインへのカルシウム結合の関与を明らかにする.
主な方法:
- 個々の融合孔を通るカテキオラミン流出のアンペロメトリック記録.
- Syt発現レベルを変えるための遺伝子操作 (トランスフェクション).
- サイト・ディレクテッド・ミュータゲネシスで,Syt IとSyt IVにおけるCa2+リガンドドメインの機能を調べる.
- フォルスコリンの使用による内生性Syt IVの薬理学的誘導.
主要な成果:
- シナプトタグミンIV (Syt IV) の過剰発現は,振幅を変えることなくキス&ランイベントの頻度と期間を増加させた.
- Syt IのC2AドメインのCa2+リガンドの変異は完全な融合を阻害しました.
- Syt IVのC2Bドメインにおける同類のCa2+リガンドの変異がキス・アンド・ランを抑制した.
- 完全融合のためのカルシウム感受性は,Syt IでSyt IVよりも高かったが,キス&ランの差異は小さかった.
結論:
- シナプトタグミンタンパク質は,エクソサイトーシスのモード (完全な融合対キス&ラン) を決定する重要なレギュレータとして作用します.
- この経路の選択には,特定のC2ドメイン (Syt I のC2A,Syt IV のC2B) にカルシウムの結合が不可欠である.
- これらの発見は,膀融合イベントの微分調節に関する分子洞察を提供します.
関連する概念動画
 01:18
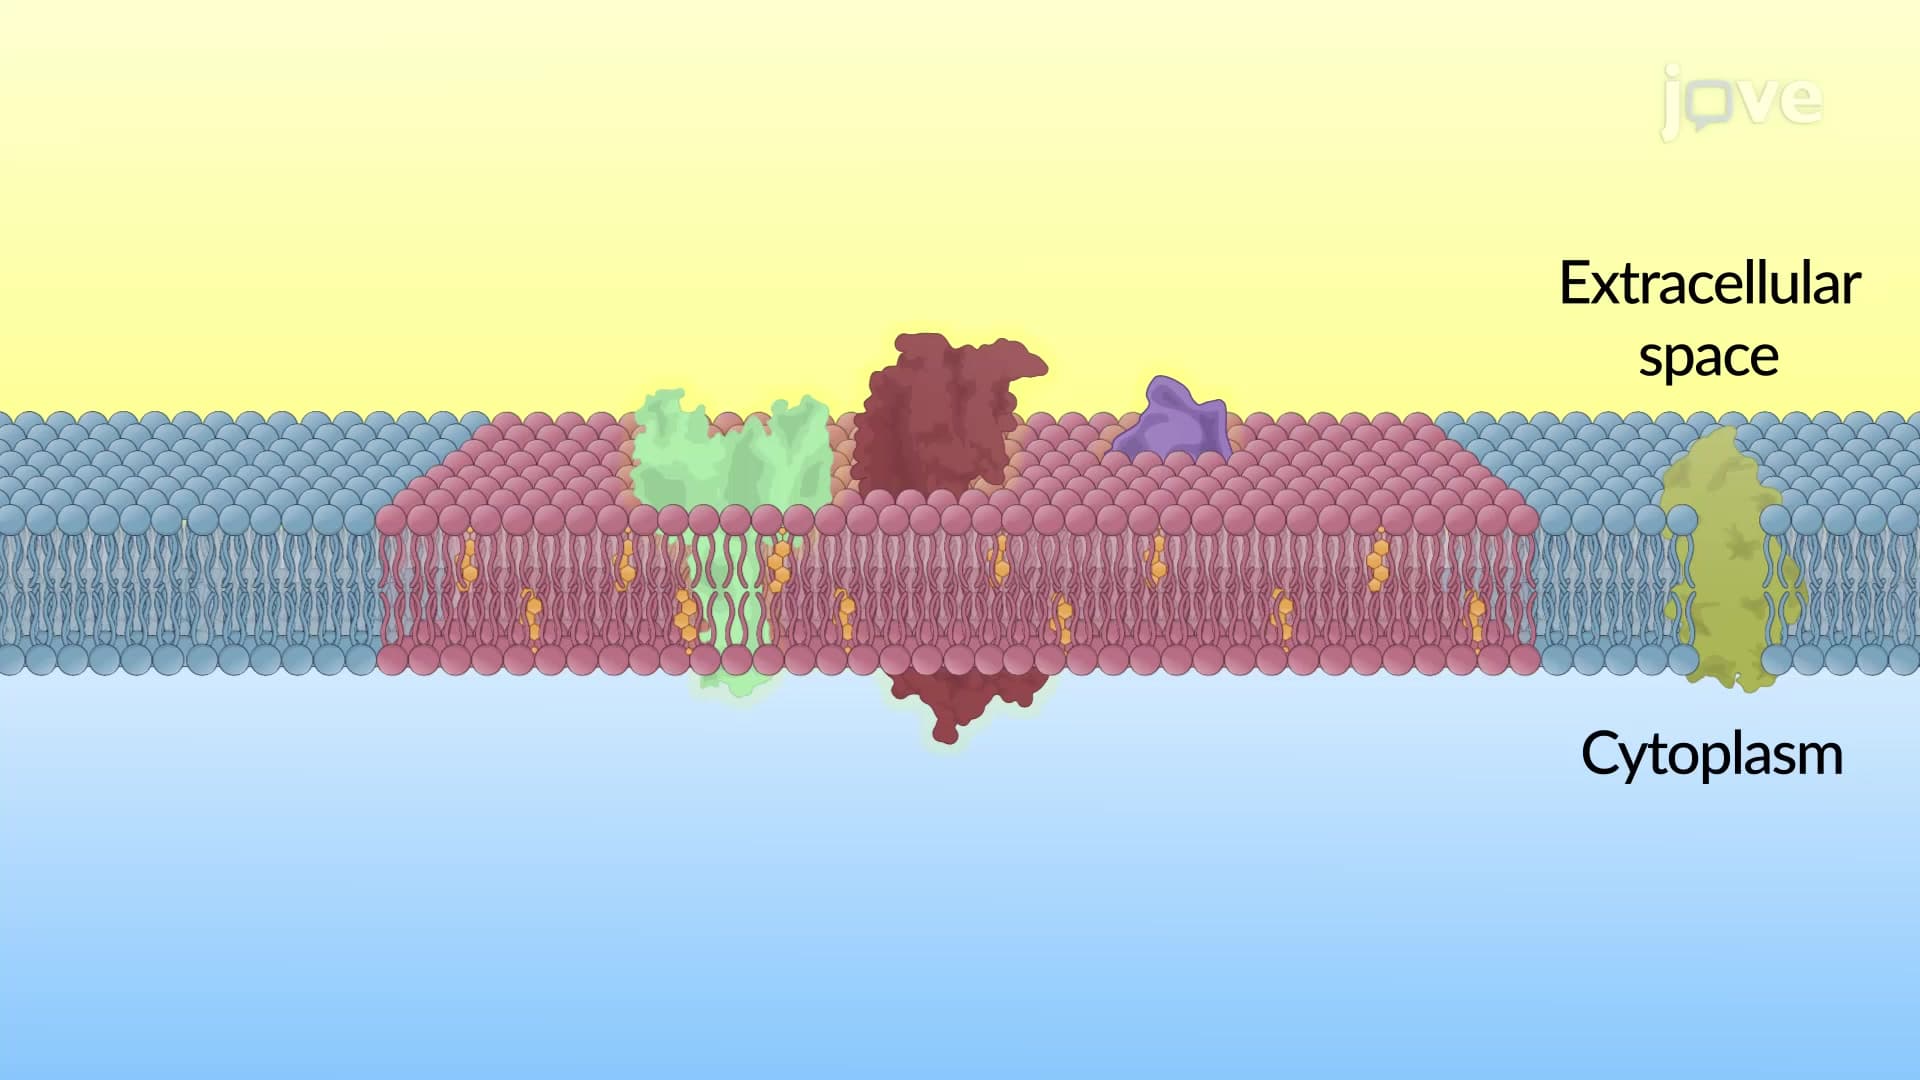
Membrane Domains
The membrane domains concentrate specific lipids and proteins at one place within the membrane, which helps in cell signaling, adhesion, and other critical cellular processes. These domains can differ in size, composition, function, and lifespan.
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the anterior...
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the anterior...
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:32
Pinching-off of Coated Vesicles
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
 01:43
SNAREs and Membrane Fusion
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 00:59
Mechanisms of Membrane Domain Formation
Different physical properties of lipids and proteins allow them to localize and form distinct islands or domains in the membrane. Some membrane domains are formed due to protein-protein interactions, whereas others are formed due to the presence of specific lipids such as sphingolipids and sterols—for example, large proteins, such as bacteriorhodopsin, aggregate and create distinct domains.
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:25
Rab Cascades
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.