関連する実験動画
Updated: Jul 15, 2026
12:15

In Vitro Polymerization of F-actin on Early Endosomes
Published on: August 28, 2017
フォーミンはプロセシブモーターで,プロフィリンはアクチン組立と関連するATP水解を加速するために必要です
Stéphane Romero1, Christophe Le Clainche, Dominique Didry
1Laboratoire d'Enzymologie et Biochimie Structurales, Centre National de la Recherche Scientifique, Avenue de la Terrasse, 91198 Gif-sur-Yvette, France.
Cell
|October 28, 2004

まとめ
フォーミン (アクチン組成を誘発するタンパク質) は,ATPエネルギーを利用して,迅速で過程的な繊維の成長を促進します. このメカニズムは,in vivoで観察された急速なアクチンベースの細胞運動を説明します.
科学分野:
- 細胞生物学 細胞生物学
- バイオケミストリー バイオケミストリー
- バイオフィジックス 生物物理学
背景:
- アクチンフィラメントの組み立ては,細胞の運動性と形態変異に不可欠です.
- フォーミンは,FH1およびFH2ドメインを有するアクチン組成の主要なイニシアターです.
- フォーミンがプロセシブアクチンポリメリゼーションを達成するメカニズムは不明である.
研究 の 目的:
- フォーミン媒介のプロセス性アクチンポリメリゼーションのメカニズムを解明する.
- フォーミン機能におけるATP水解とプロフィリンの役割を調査する.
- in vitroでホルミン誘発の運動性を復元するために.
主な方法:
- アクチンポリメリゼーションと結合したATPの水解速度を測定する生化学分析.
- フィラメントの刺さった端におけるプロフィリン-アクチン結合運動学的分析.
- フォルミン駆動のアクチンフィラメントの延長をビールを用いてin vitroで再構成する.
主要な成果:
- フォーミンFH1-FH2ドメインは,プロフィリン-アクチンのポリメリゼーション中にATPの水解を加速します.
- この加速水解は,プロセシブポリメリゼーションのための自由エネルギーを供給し,結合率を15倍に増加させます.
- プロフィリンは,プロセッシブ機能に不可欠であり,積極的に参加します.
- 長いアクチンフィラメント (≥10μm) は,分離することなく,実験室で形成されました.
- 暫定的なプロセスは,タンパク質を封じ込めることによる循環の阻害の結果である.
結論:
- フォーミンはATPに依存するモーターとして作用し,プロセシブアクチンアセンブリのためのカップリングされた水解を利用します.
- プロフィリンは,このプロセスの重要なコファクターです.
- in vitroで再構成されたシステムは,in vivoで観察された急速なホルミン駆動アクチンダイナミクスを説明します.
関連する概念動画
 01:42
Actin Polymerization
Actin polymerization occurs through the head-to-tail association of binding sites on monomeric actin or G-actin to form filamentous or F-actin. The polymerization can be divided into three phases ̶ nucleation, elongation, and steady-state phase.
The nucleation phase involves forming a stable nucleus consisting of three actin monomers to form a new actin filament. Actin-binding proteins such as formins and Arp2/3 complex help filament growth post-nucleation. The Formins form straight actin...
The nucleation phase involves forming a stable nucleus consisting of three actin monomers to form a new actin filament. Actin-binding proteins such as formins and Arp2/3 complex help filament growth post-nucleation. The Formins form straight actin...
 01:14
Generation of Straight or Branched Actin Filaments
The straight or branched structure formation of actin filaments is controlled by nucleating proteins such as the formins and Arp2/3 complex. Formin-mediated assembly results in straight filaments, whereas Arp2/3 protein complex-mediated assembly results in branched actin filaments.
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
 01:19
Actin Filament Depolymerization
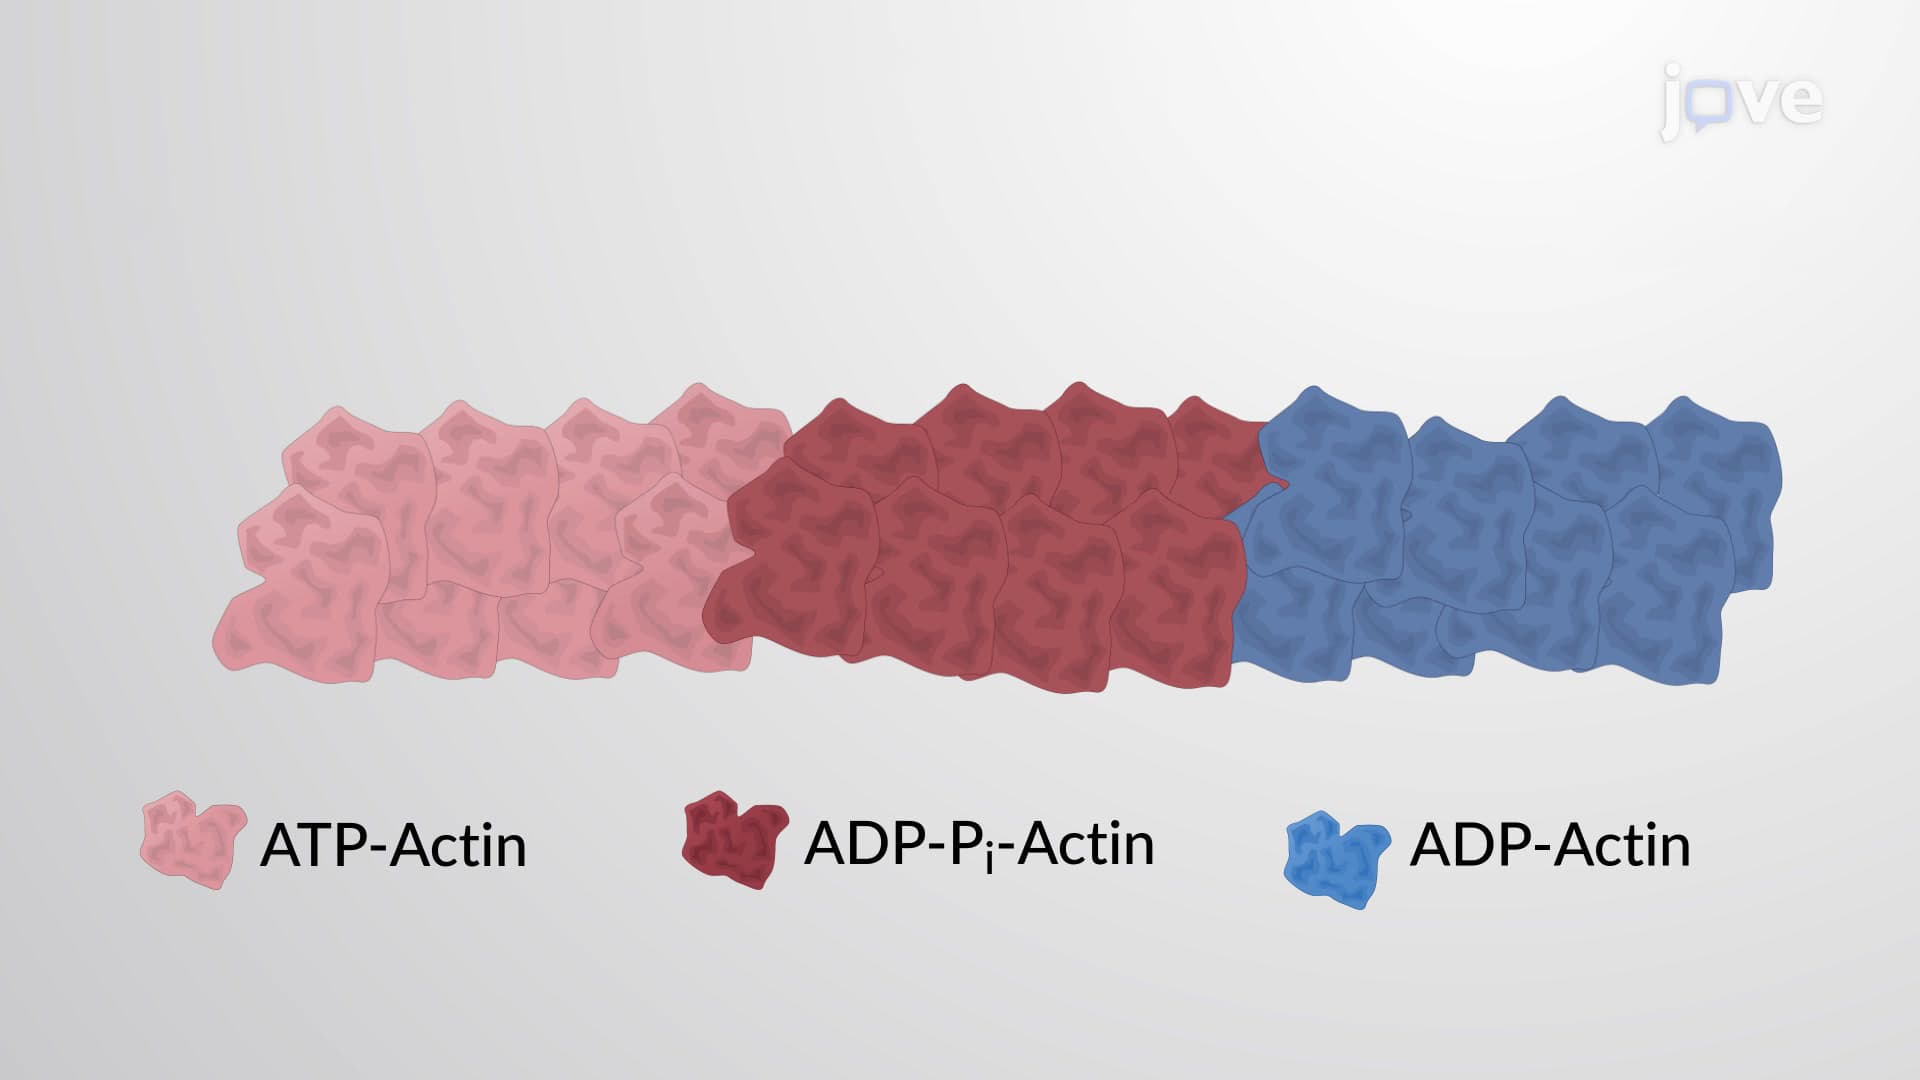
Actin filaments (F-actin) are composed of actin subunits. The dissociation of actin monomers can occur from either end of F-actin. The rate of dissociation is faster from the minus-end or the pointed end, where the actin subunits exist with a bound ADP, together known as ADP-actin. The depolymerization of F-actin is aided by proteins, including the actin-depolymerizing factor (ADF) and cofilin family of proteins, gelsolin, and glia maturation factor (GMF).
In F-actin, the ADF/cofilin proteins...
In F-actin, the ADF/cofilin proteins...
 01:11
Formation of Higher-order Actin Filaments
The polymerization of G-actin monomers into filamentous F-actin is a multi-step process. Once the F-actins are formed, they can bundle together in different arrangements to form higher-order networks and regulate cellular functions. Common examples include the formation of lamellipodia and filopodia at the cell's leading edge by actin reorganization in a migrating cell. The microvilli on the brush border epithelial cells are also formed through the F-actin network.
The high-order actin networks...
The high-order actin networks...
 01:39
Mechanism of Filopodia Formation
Filopodia are thin, actin-rich cellular protrusions that play an important role in many fundamental cellular functions. They vary in their occurrence, length, and positioning in different cell types, suggesting their diverse roles.
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
 01:18
Actin Treadmilling
Actin filaments undergo polymerization and depolymerization from either end. The polymerization and depolymerization rates depend on the cytosolic concentration of free G-actins. The polymerization rate is generally higher at the plus or barbed end, while the depolymerization rate is higher at the minus or pointed end. At a steady state, critical concentration describes the concentration of free G-actin monomers at which the polymerization rate at the plus end is equal to that of the...