
形式化ドメイン: 線形グラミシジニンの非リボソーム生物合成のための重要な修飾酵素
Georg Schoenafinger1, Nadine Schracke, Uwe Linne
1Fachbereich Chemie/Biochemie, Philipps-Universität Marburg, Hans-Meerwein-Strasse, D-35032 Marburg, Germany.
Journal of the American Chemical Society
|June 8, 2006

まとめ
この研究は,非リボソーム性ペプチド合成酵素LgrA1.1によるグラミシジン生物合成の開始にN型化が不可欠であることを明らかにしています. 形式化ドメインは,ホルミール基をバリンに転送し,ペプチド鎖の延長に必要なスタートユニットを作成します.
科学分野:
- バイオケミストリー バイオケミストリー
- 分子生物学は分子生物学である.
- 酵素学 酵素学とは
背景:
- N-ホルミレーションは,プロカリオットリボソームペプチド合成の重要なステップです.
- N-フォーミレーションは,非リボソームペプチド合成 (NPS) で珍しく,ほとんど研究されていない.
- 線形グラミシジン非リボソームペプチド合成酵素 (LgrA) システムの初期段階は完全に理解されていませんでした.
研究 の 目的:
- LgrA1モジュールのホルミルトランスフェラーゼ活性を調べるために.
- グラミシジンバイオシンセシスの開始にN形式化が必要かどうかを判断する.
- NPS.における新しい裁縫酵素を特定する.
主な方法:
- LgrA1モジュールのフォームリトランスフェラーゼ活性に対するインビトロ測定.
- フォルミルトラヒドロフォラート (fH4F) からバリンへのホルミル群の移転を試験する.
- 伸縮測定は,ホルミール群のドナーを含む,または含まない二模様LgrAシステムを用いて行われます.
主要な成果:
- LgrA1の推定形式化ドメインは,N10-およびN5-fH4Fから形式基をバリンに成功的に転送しました.
- フォーミル・ヴァリンは,グラミシジン生物合成の重要なスタートユニットとして確認されました.
- 延長測定では,ホルミールドナーなしではダイペプチドの形成が示されず,ホルミル-ヴァリル-グリシンが生成された.
結論:
- LgrAの第1ドメインはホルミルトランスフェラーゼ活性を示し,NPSにおけるその役割を確認した.
- この発見は,非リボソームペプチド合成経路における新しい調整酵素を特定しています.
- N-ホルミレーションは,グラミシジン生物合成の開始において,これまで認識されていない重要なステップです.
関連する概念動画
 01:27
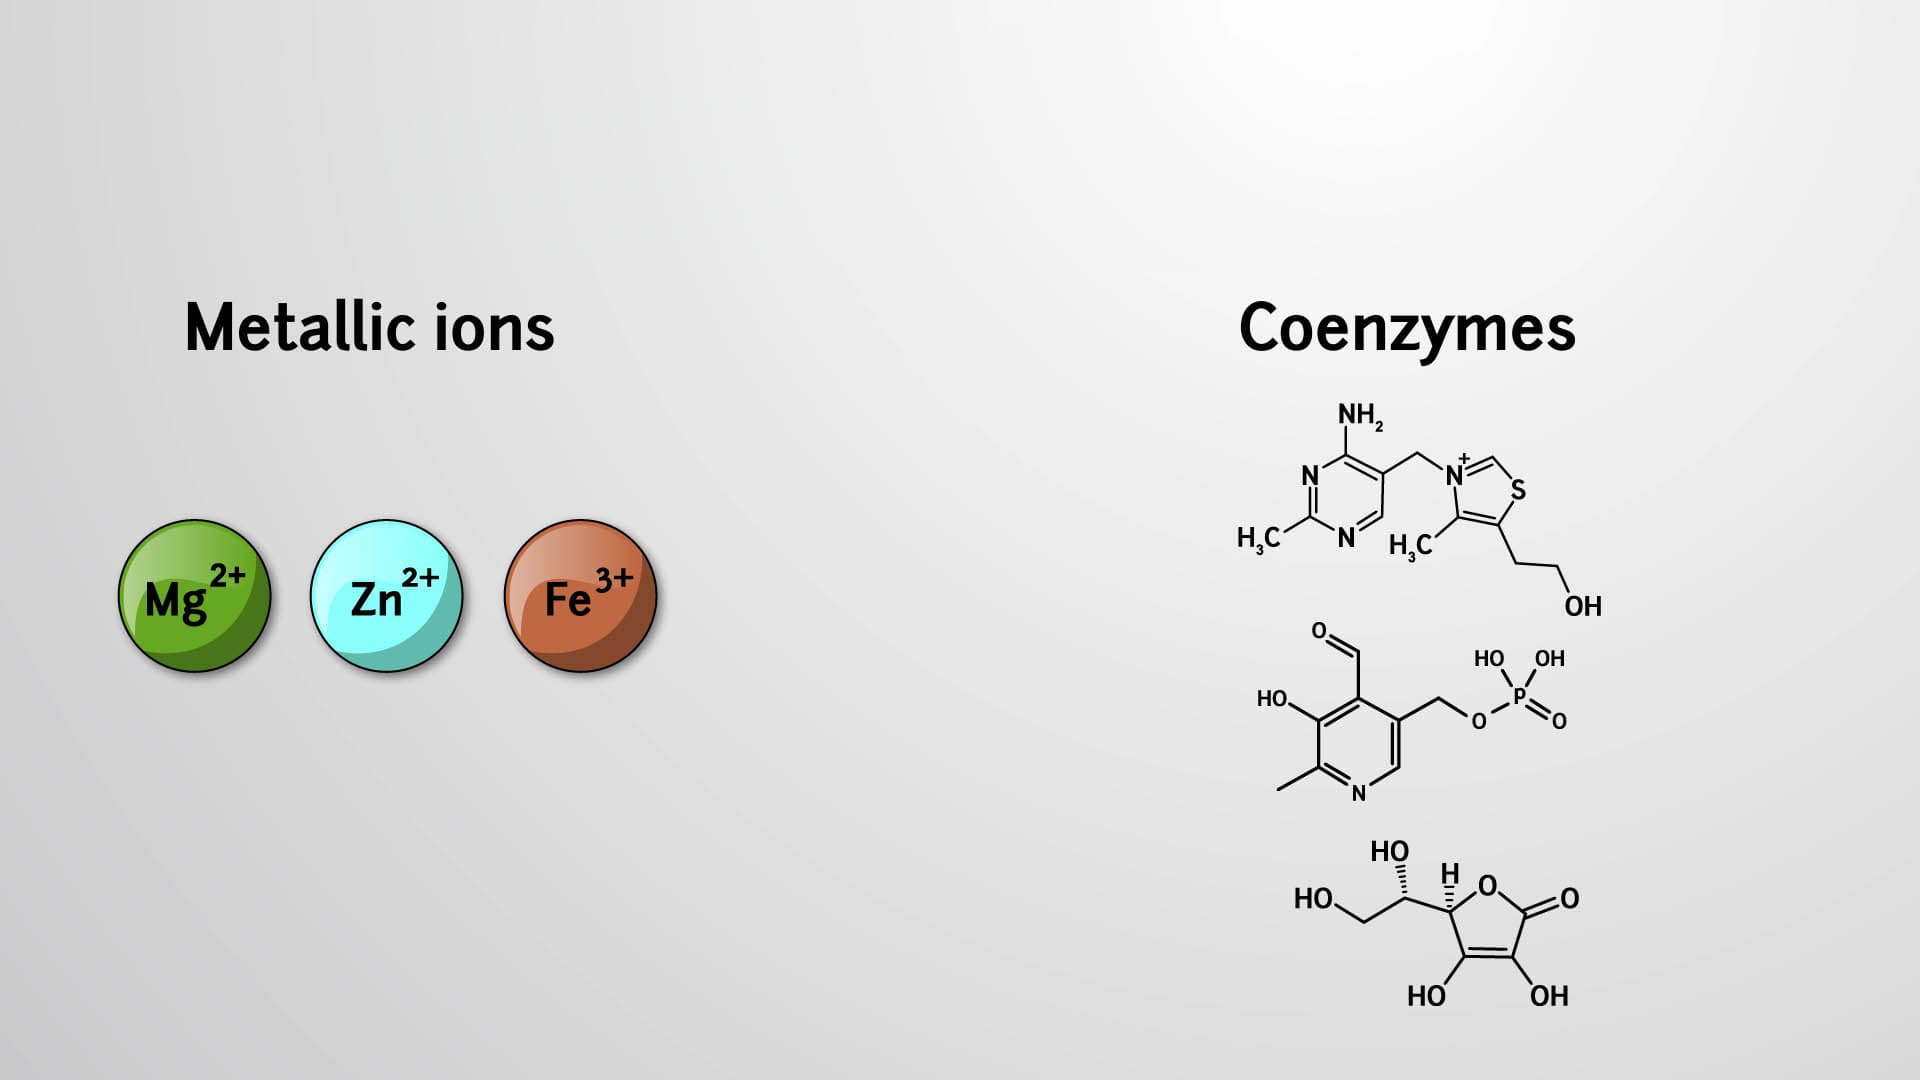
Cofactors and Coenzymes
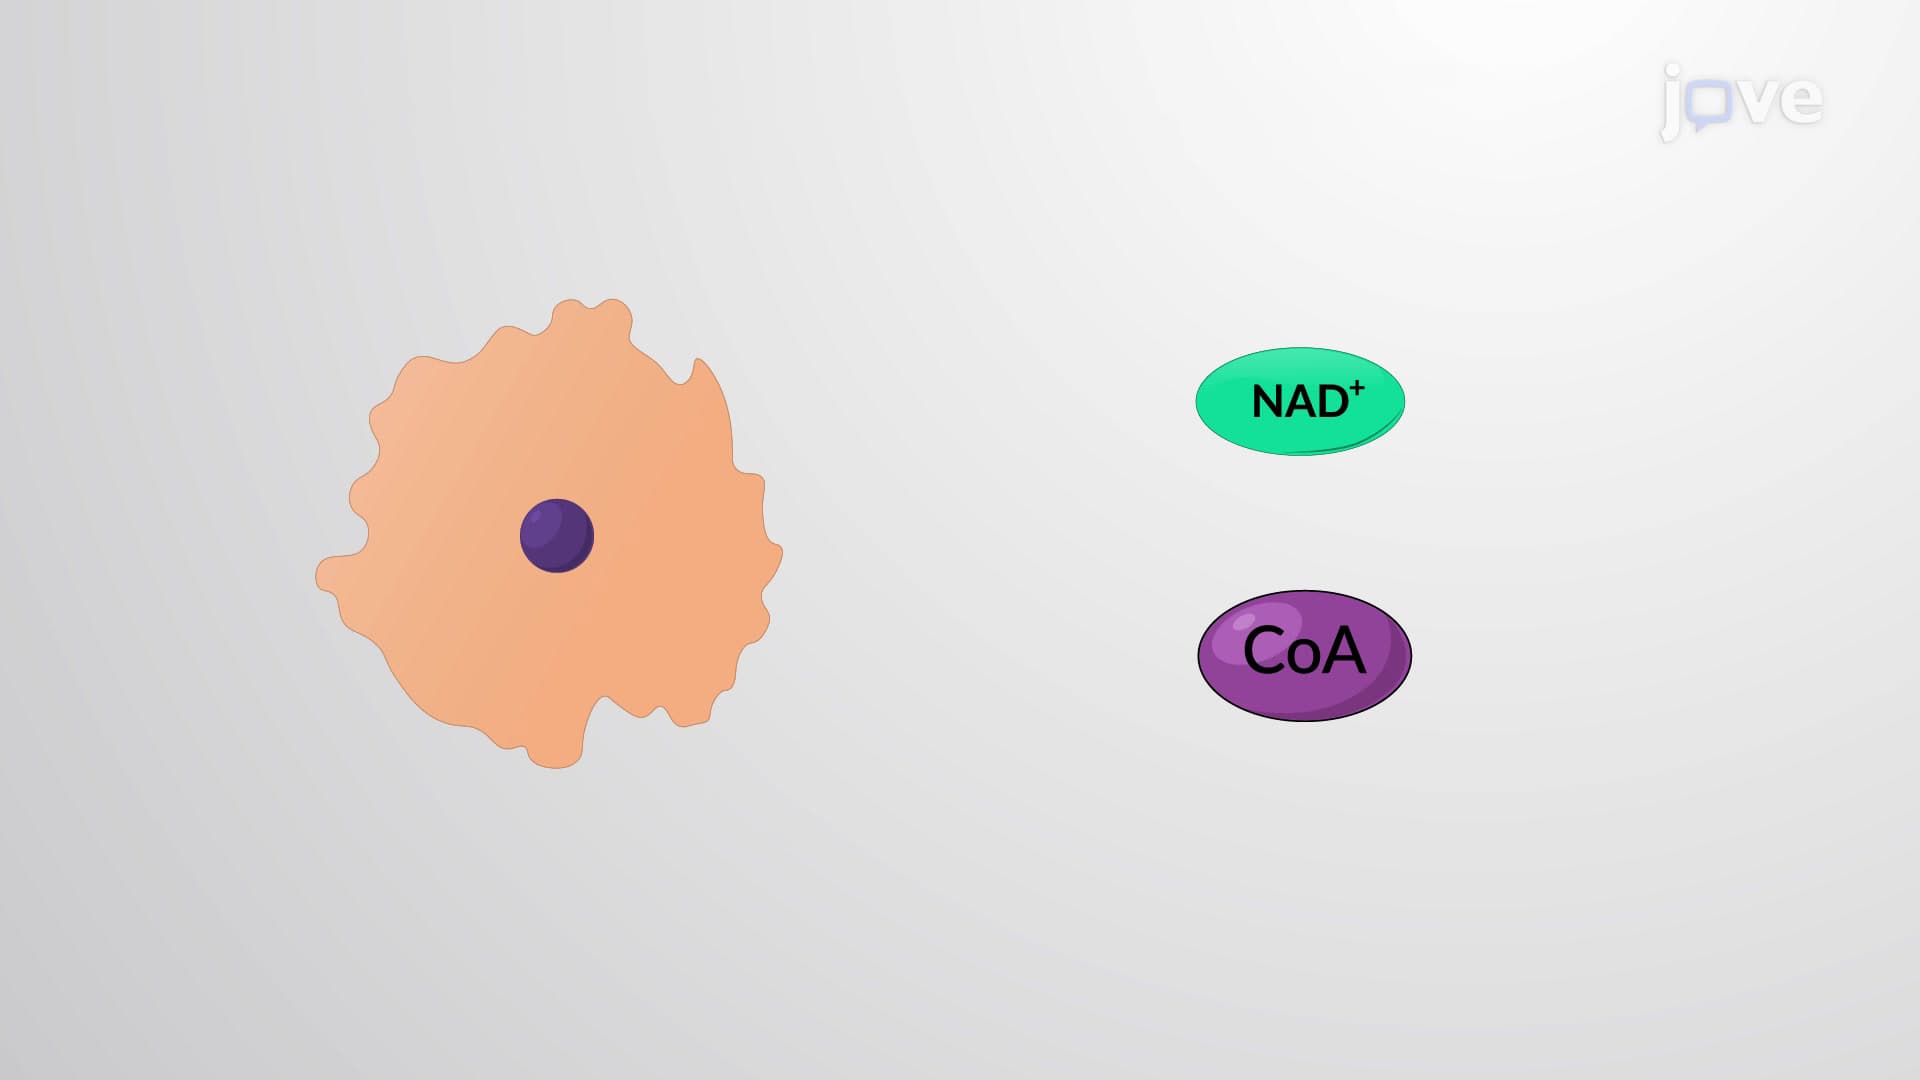
Enzymes require additional components for proper function. There are two such classes of molecules: cofactors and coenzymes. Cofactors are metallic ions and coenzymes are non-protein organic molecules. Both of these types of helper molecule can be tightly bound to the enzyme or bound only when the substrate binds.
01:27Cofactors and Coenzymes
Enzymes require additional components for proper function. There are two such classes of molecules: cofactors and coenzymes. Cofactors are metallic ions and coenzymes are non-protein organic molecules. Both of these types of helper molecule can be tightly bound to the enzyme or bound only when the substrate binds.
 01:24
Cofactors and Coenzymes
Enzymes are proteins made of amino acids. The functional group of each constituent amino acid catalyzes a wide variety of chemical reactions via ionic interactions or acid-base reactions. However, amino acids cannot catalyze oxidation-reduction and group transfer reactions and need to be aided by non-protein components called cofactors. Cofactors are also referred to as the chemical teeth of an enzyme.
Cofactors can be metallic ions or organic molecules called coenzymes. These types of helper...
Cofactors can be metallic ions or organic molecules called coenzymes. These types of helper...
 01:18
Amino Acid Catabolism
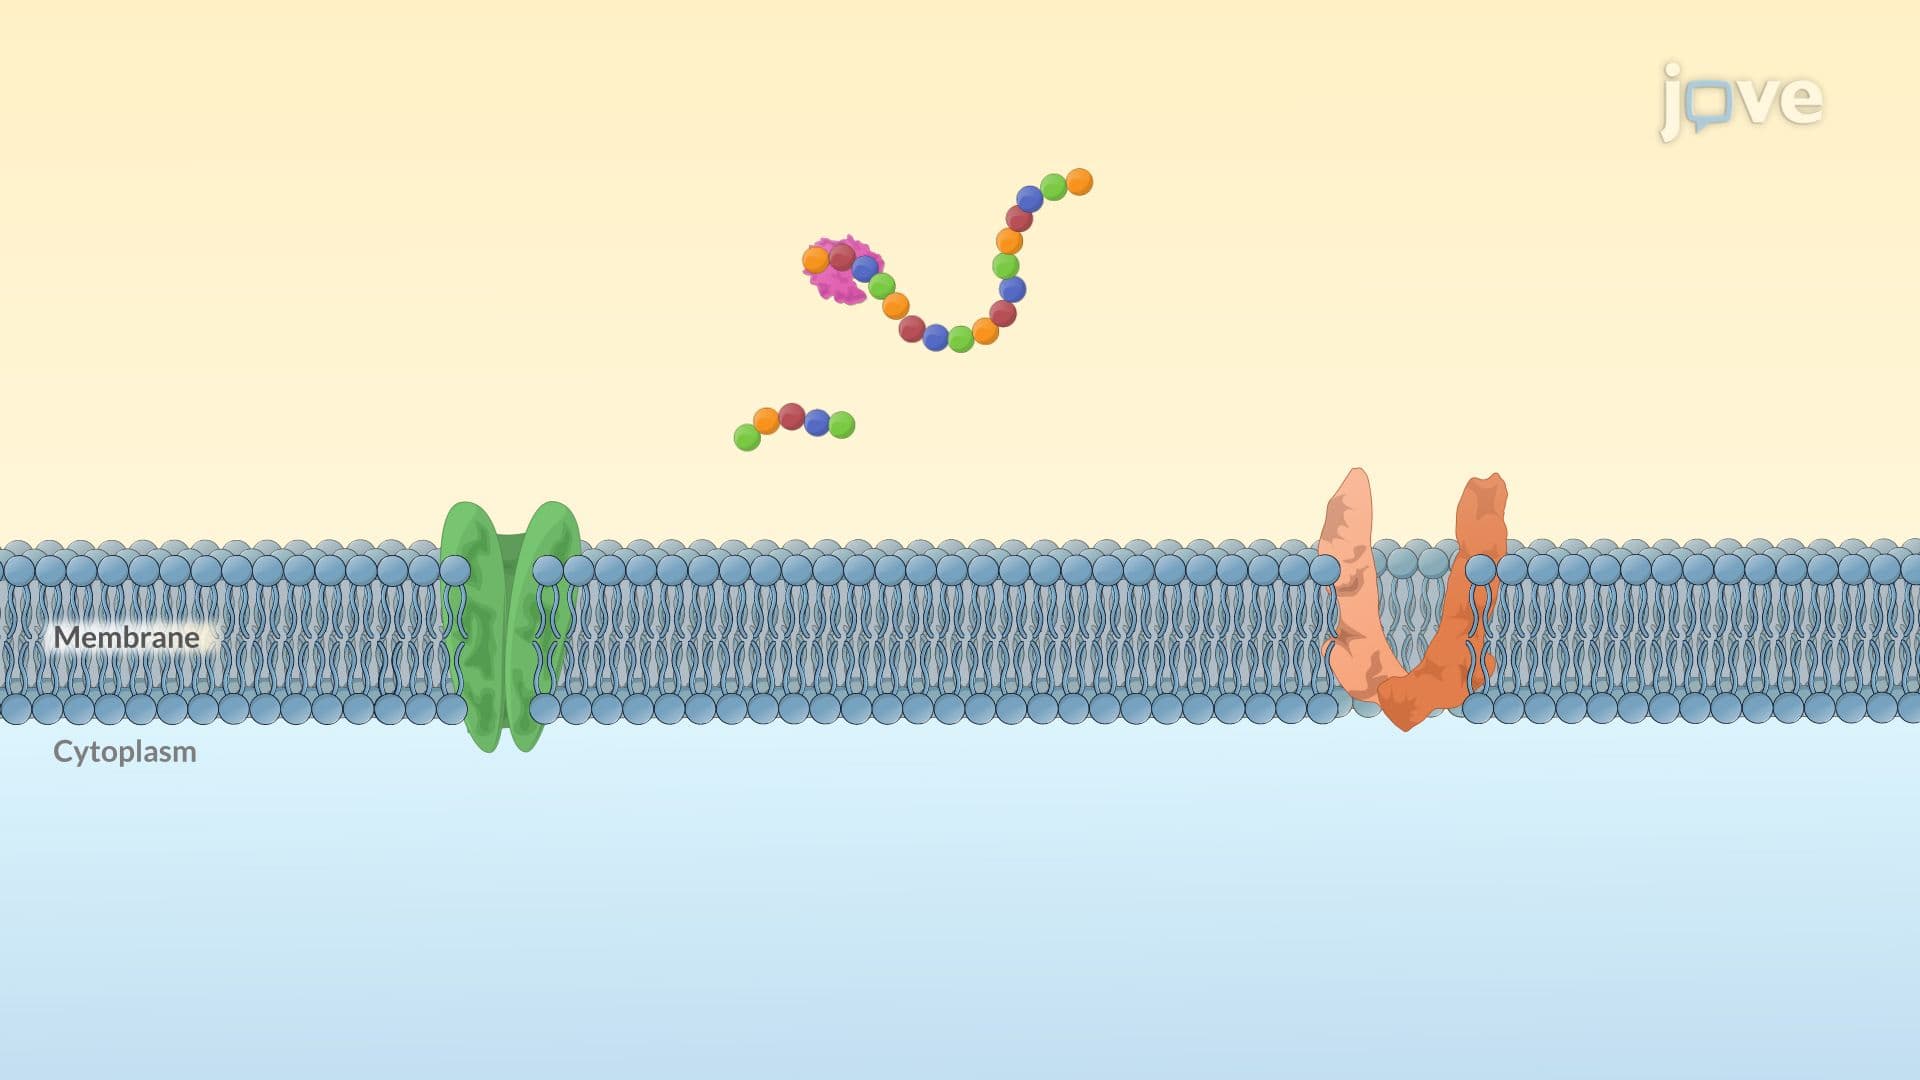
Microorganisms rely on proteins as an essential carbon and energy source, particularly in environments with limited polysaccharides or lipids. However, proteins are too large to cross the plasma membrane unaided, necessitating enzymatic degradation. Microbes secrete extracellular proteases and peptidases that hydrolyze proteins into peptides, which can then be transported across the membrane. Once inside the cell, intracellular proteases degrade these peptides into free amino acids, which...
 01:20
Sulfur Assimilation
Sulfur is an essential element in biological systems, contributing to synthesizing key biomolecules, including amino acids such as cysteine and methionine, and cofactors such as coenzyme A and biotin. Microorganisms primarily assimilate sulfur as sulfate (SO₄²⁻) from the environment, which must undergo a series of biochemical transformations before it can be incorporated into cellular components. As sulfate is highly oxidized, it must undergo assimilatory sulfate reduction to become...
 01:29
Amino Acid Biosynthetic Pathways
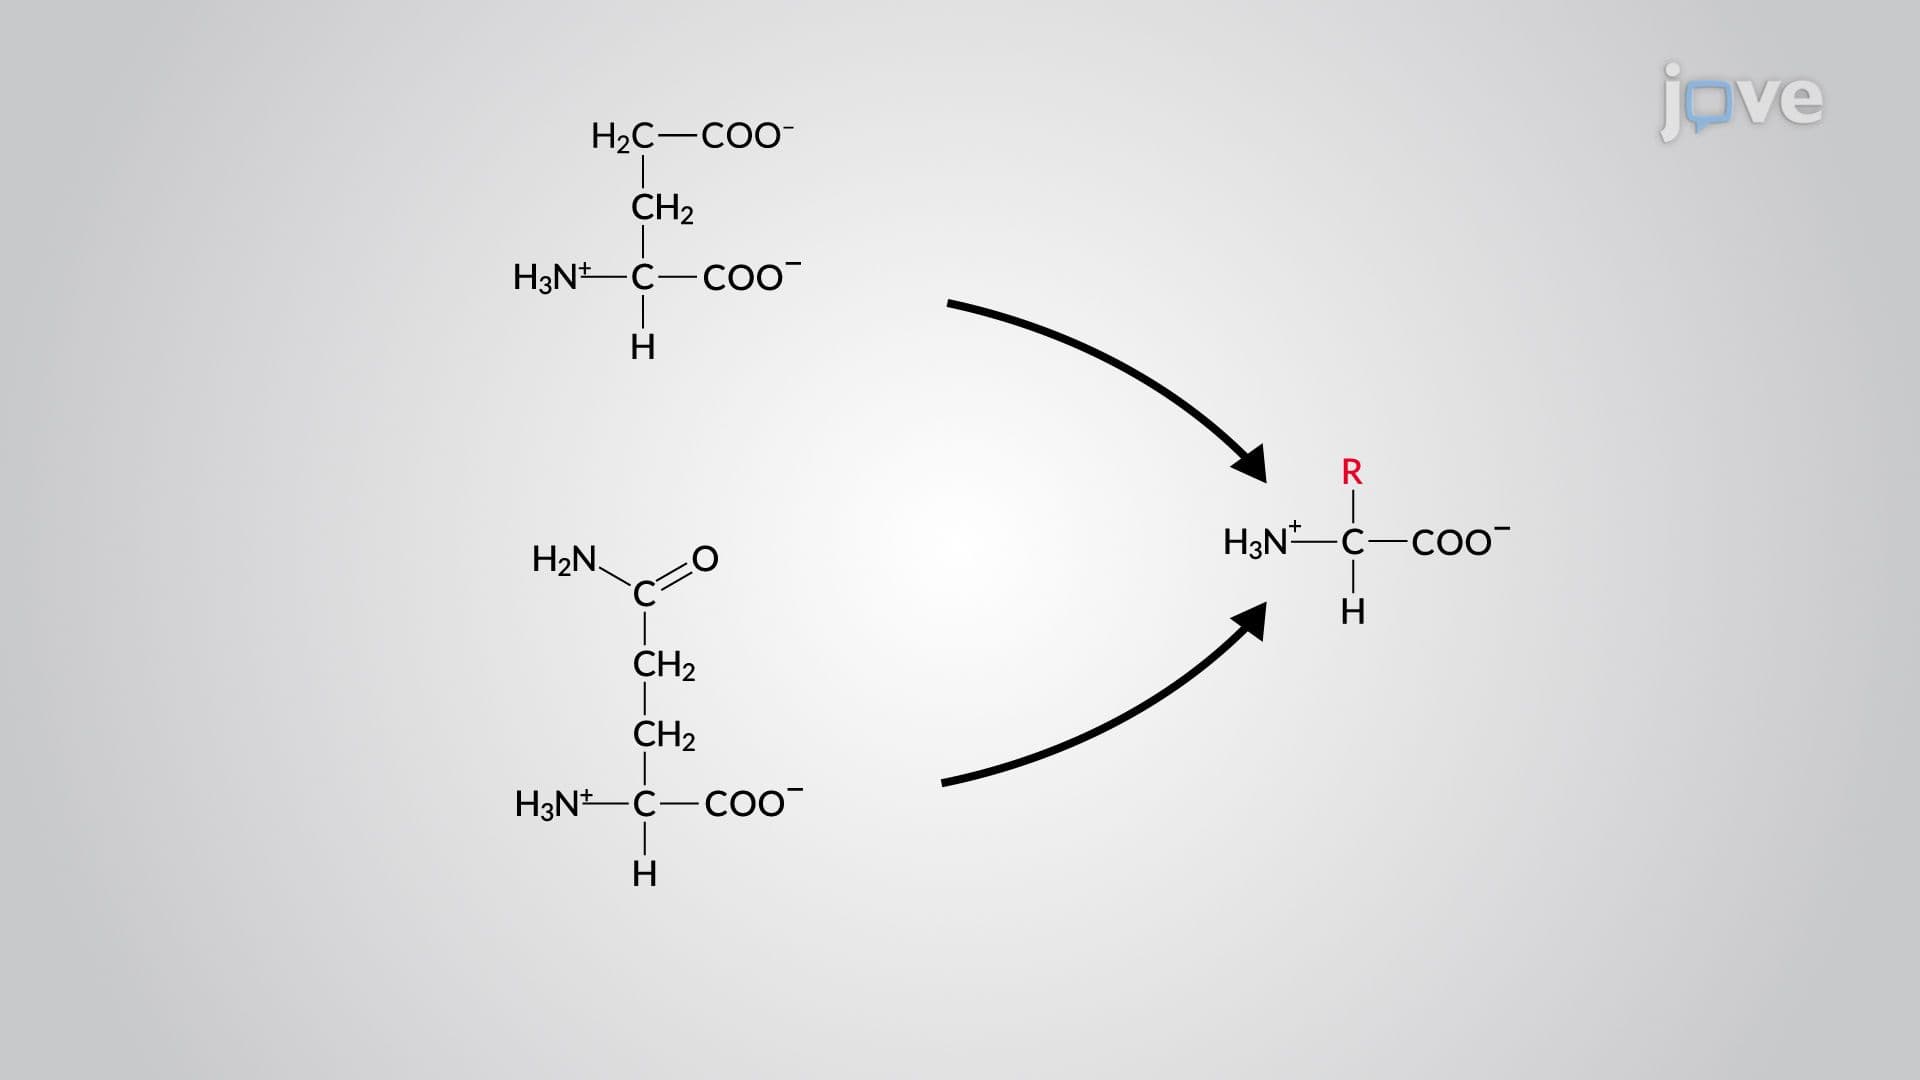
Amino acid biosynthesis is essential for cell growth, protein synthesis, and metabolic regulation. Cells generate essential and non-essential amino acids from metabolic intermediates to sustain vital biological functions. These intermediates originate from key metabolic pathways: glycolysis, the tricarboxylic acid (TCA) cycle, and the pentose phosphate pathway. Important precursors include α-ketoglutarate, pyruvate, oxaloacetate, phosphoenolpyruvate, and erythrose-4-phosphate, which provide...