関連する実験動画
Updated: Aug 9, 2026
07:17

Purification of Hsp104, a Protein Disaggregase
Published on: September 30, 2011
プリオンタンパク質のストップ移転の非水害性エクストラサイトプラズマ決定因子
C S Yost1, C D Lopez, S B Prusiner
1Department of Anesthesia, University of California, San Francisco 94143.
Nature
|February 15, 1990

まとめ
研究者らは,プリオンタンパク質の充電されたエキストラサイトプラズマシーケンスが,そのトランスメブラン統合と停止転送に不可欠であることを発見しました. この発見は,膜タンパク質バイオゲネシスの新しいメカニズムを明らかにしています.
科学分野:
- 分子生物学は分子生物学である.
- タンパク質生化学 タンパク質生化学
- 細胞生物学 細胞生物学
背景:
- 統合型トランスメブランタンパク質は,膜の横断と転位終結のために,普遍的に水害性ドメインを有している.
- タンパク質の停止移転とトランスメブラン統合における細胞外血質配列の役割は,以前は確立されていなかった.
- プリオンタンパク質は異常なストップ転送と代替トポロジーを示し,ユニークなトポゲンシーケンスを示唆しています.
研究 の 目的:
- トランスメブラントポロジーを支配するプリオンタンパク質のトポゲンシーケンス内の決定因子を調査する.
- ストップ転送プロセスにおけるエクストラサイトプラズマシーケンスの役割を明らかにする.
- 膜タンパク質バイオゲネシスのメカニズムを理解するために.
主な方法:
- 細胞フリートランスレーションシステム (小麦芽とウサギの網膜細胞溶解体) を用いて,タンパク質の転位を研究した.
- プリオンタンパク質のトポゲン配列内の特定のドメインの機能を調査した.
- プリオンタンパク質の配列のトポゲン特性を評価するために異質なタンパク質を設計した.
主要な成果:
- 照明的に配置された充電ドメインは,隣接する水害ドメインによって介されるストップ転送に不可欠です.
- 充電ドメインと排水ドメインの間の空間的配置は,効率的なストップ転送に不可欠です.
- プリオンタンパク質からのエクストラサイトプラズミック水性ドメインは,異質タンパク質にトランスメブラントポロジーを授与しました.
結論:
- プリオンタンパク質で予期せぬ機能的なエクストラサイトプラズマドメインが特定され,これはストップ転送に影響を与えます.
- 充電されたエキストラサイトプラズマシーケンスが,タンパク質のトポロジーを指向する上で重要な役割を果たしていることを実証した.
- これらの発見は,膜タンパク質の生体生成と統合の基本的メカニズムを理解するための意味を持つ.
関連する概念動画
 01:19
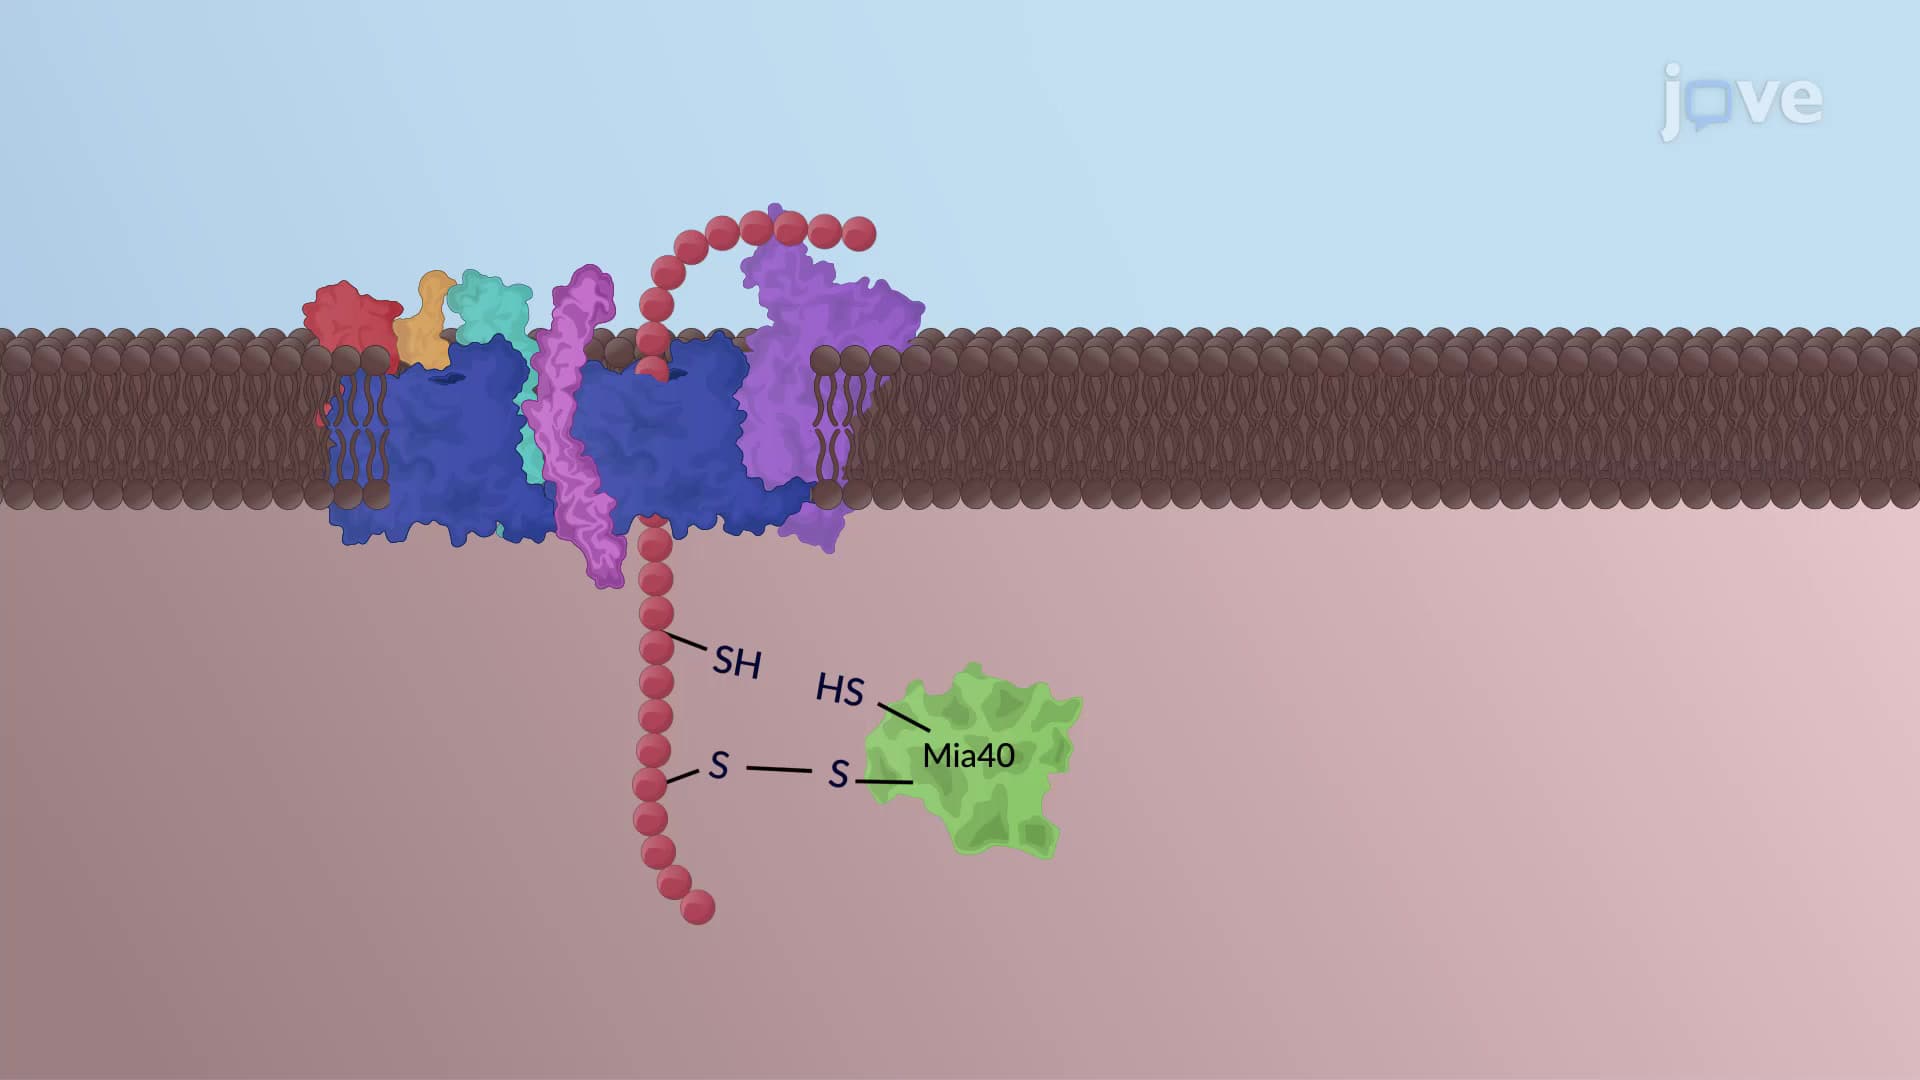
Translocation of Proteins into the Mitochondria
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
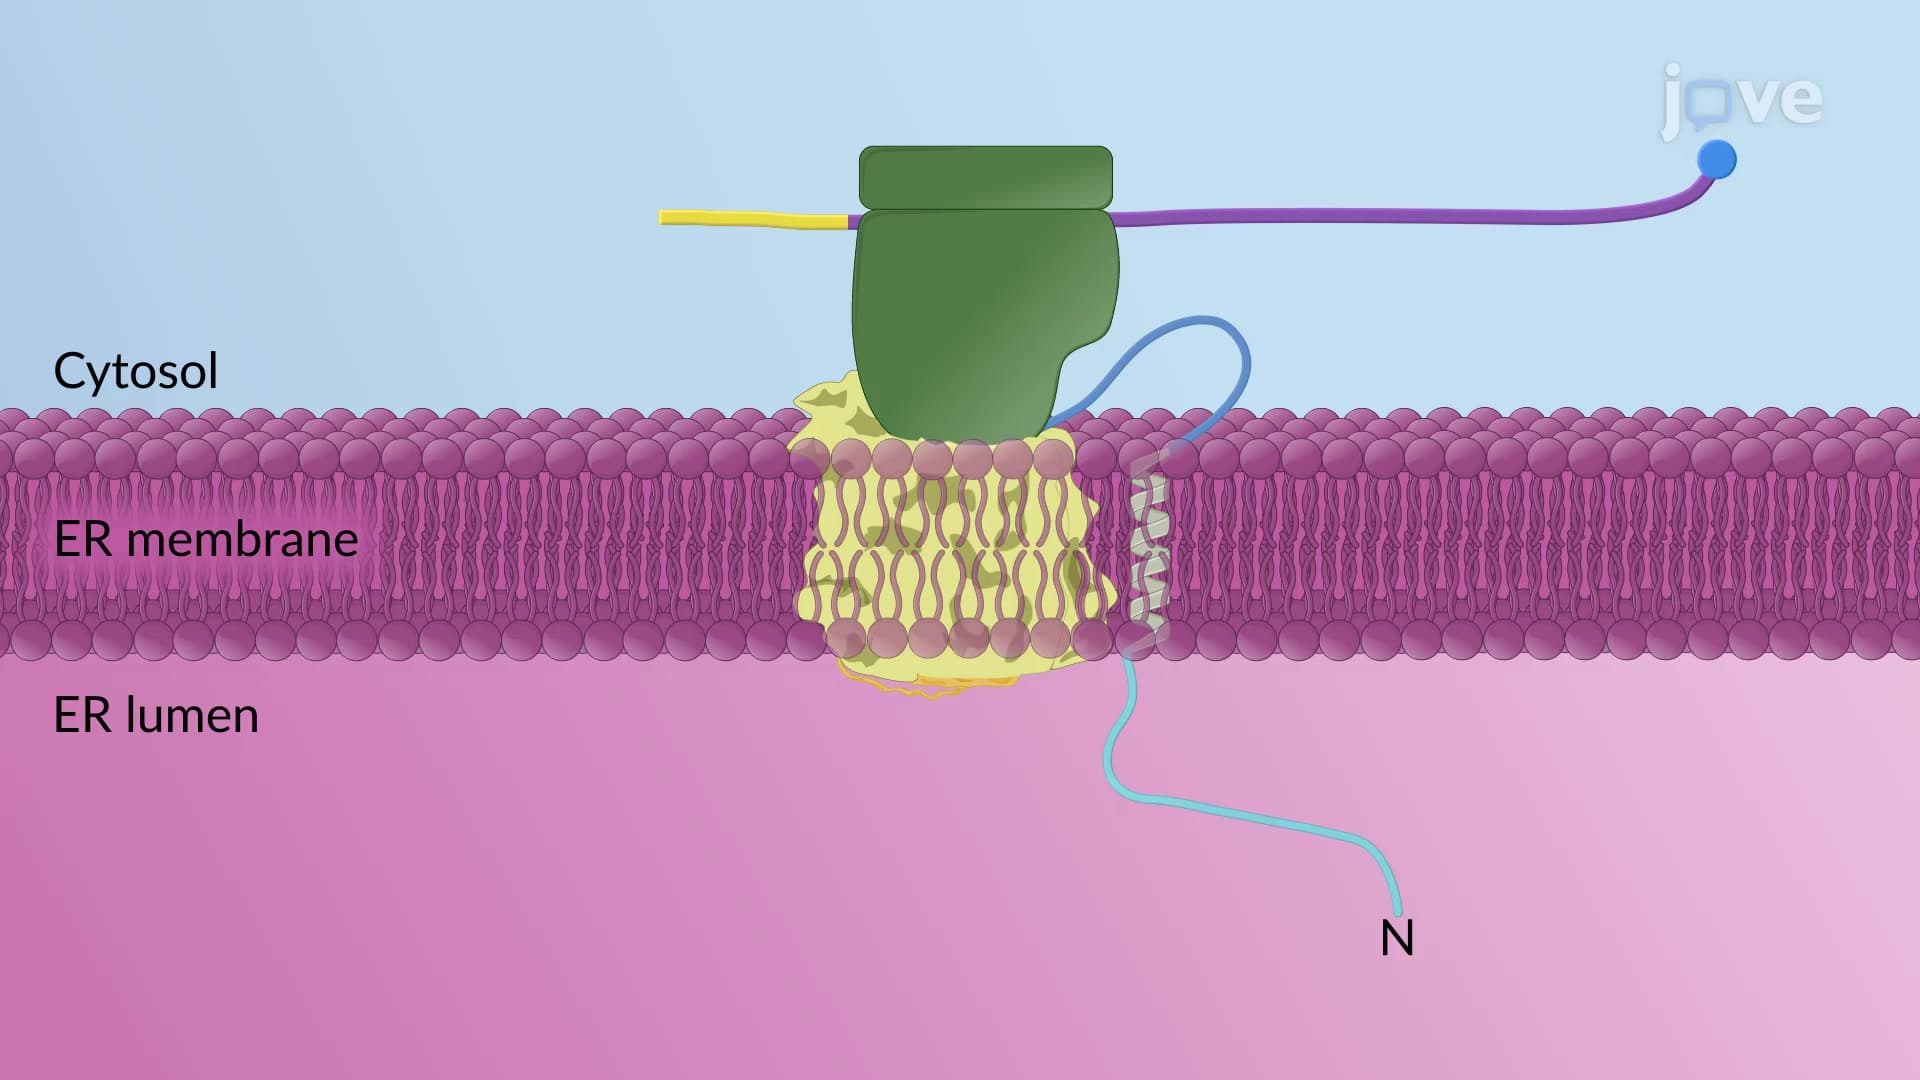 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
Integral membrane proteins are proteins adhered to the lipid bilayer of a cell organelle or membrane. They can be of two types: transmembrane integral proteins that span the lipid bilayer and monotopic proteins that are attached to either side of the membrane but do not pass through it.
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
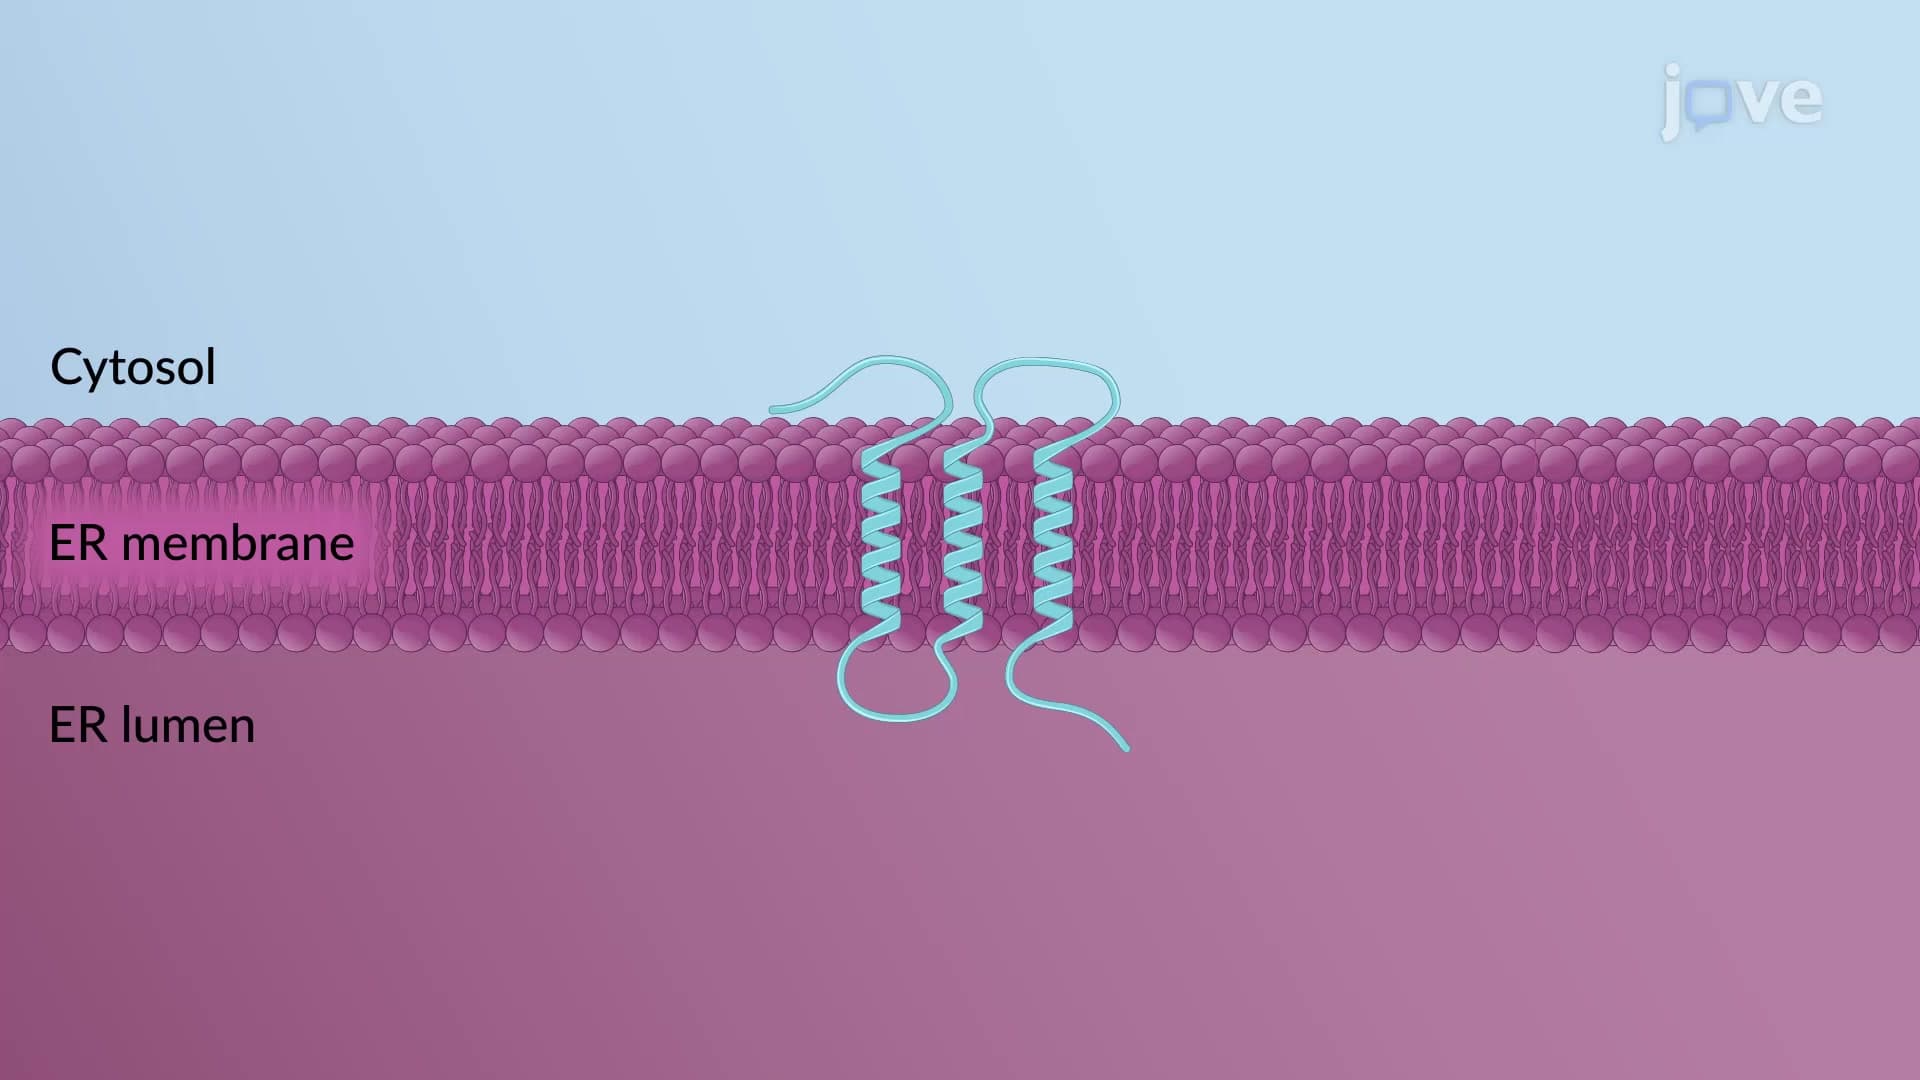 01:29
Insertion of Multi-pass Transmembrane Proteins in the RER
The rough ER membrane synthesizes, assembles, and embeds transmembrane proteins in diverse topologies. These proteins function as transporters or channels and can remain in the ER membrane or are sent to the Golgi complex, lysosome, and cell membrane.
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
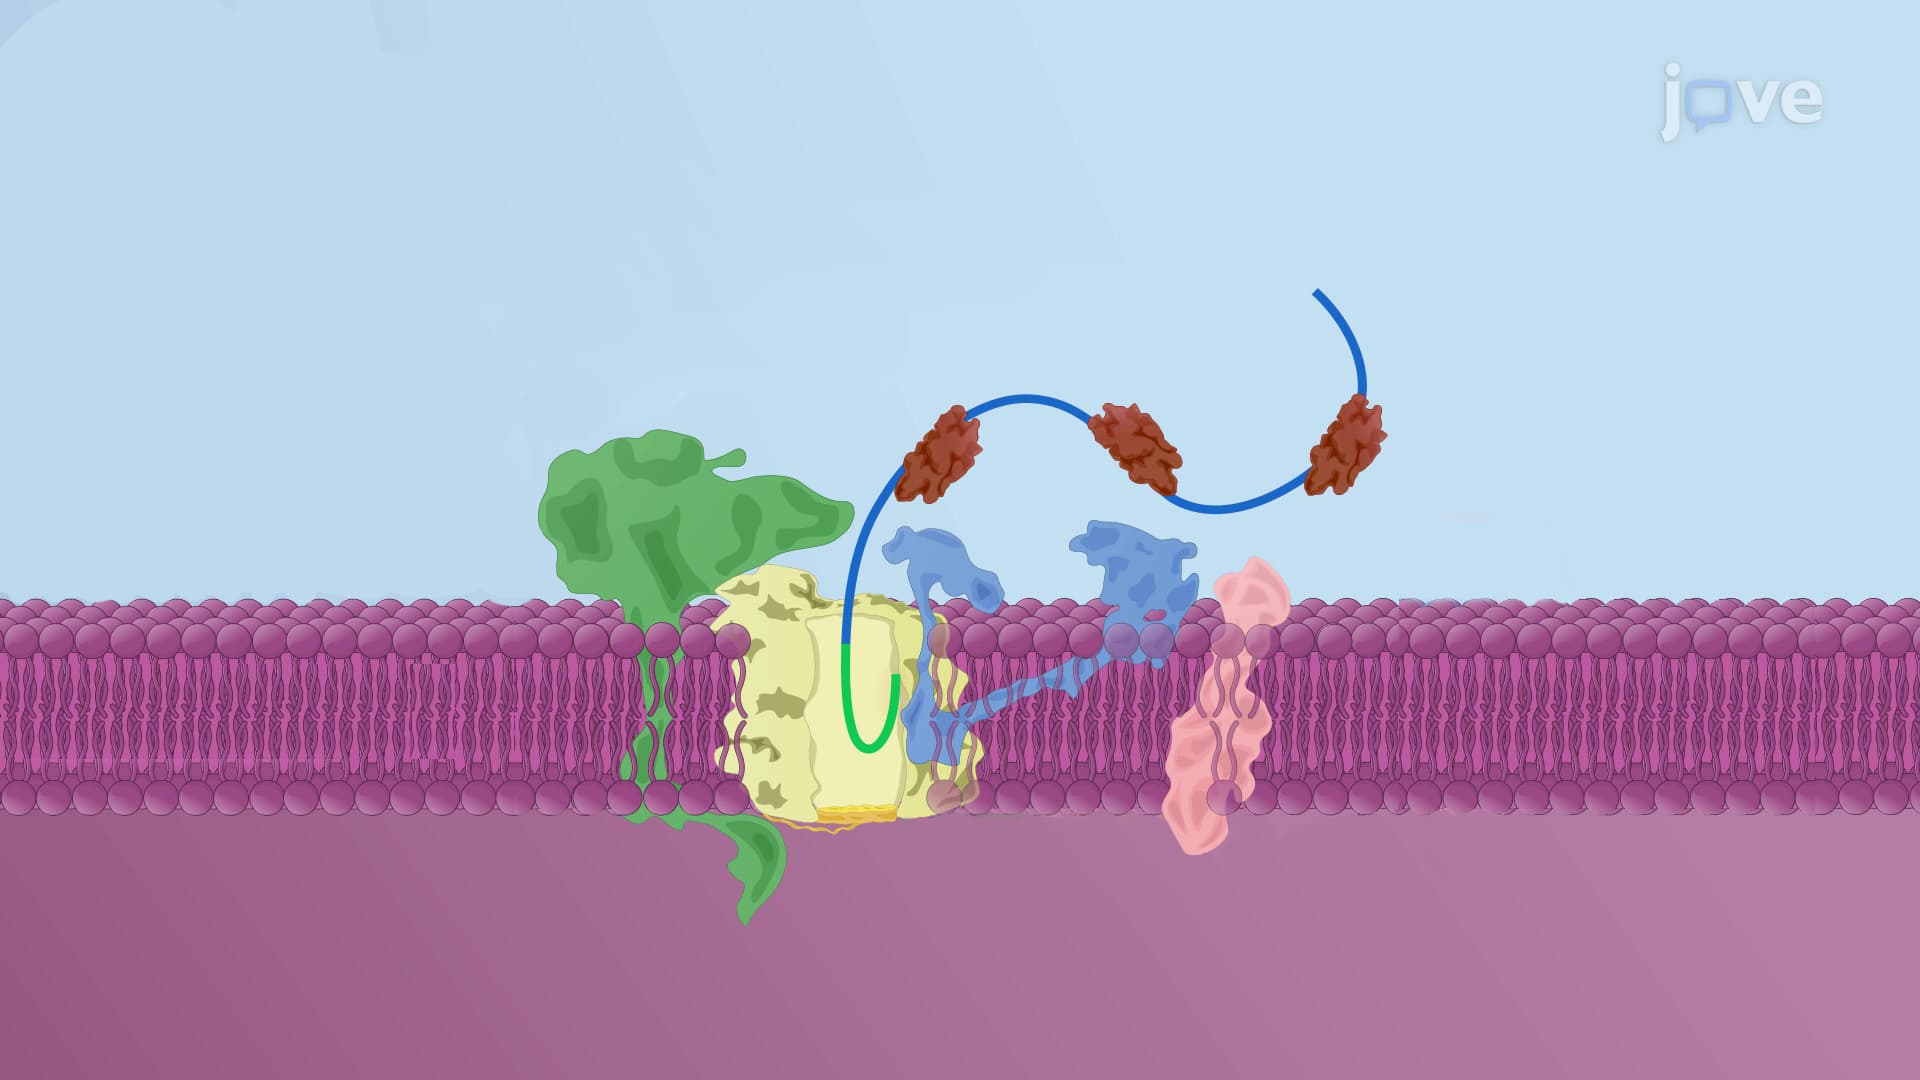 01:27
Post-translational Translocation of Proteins to the RER
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
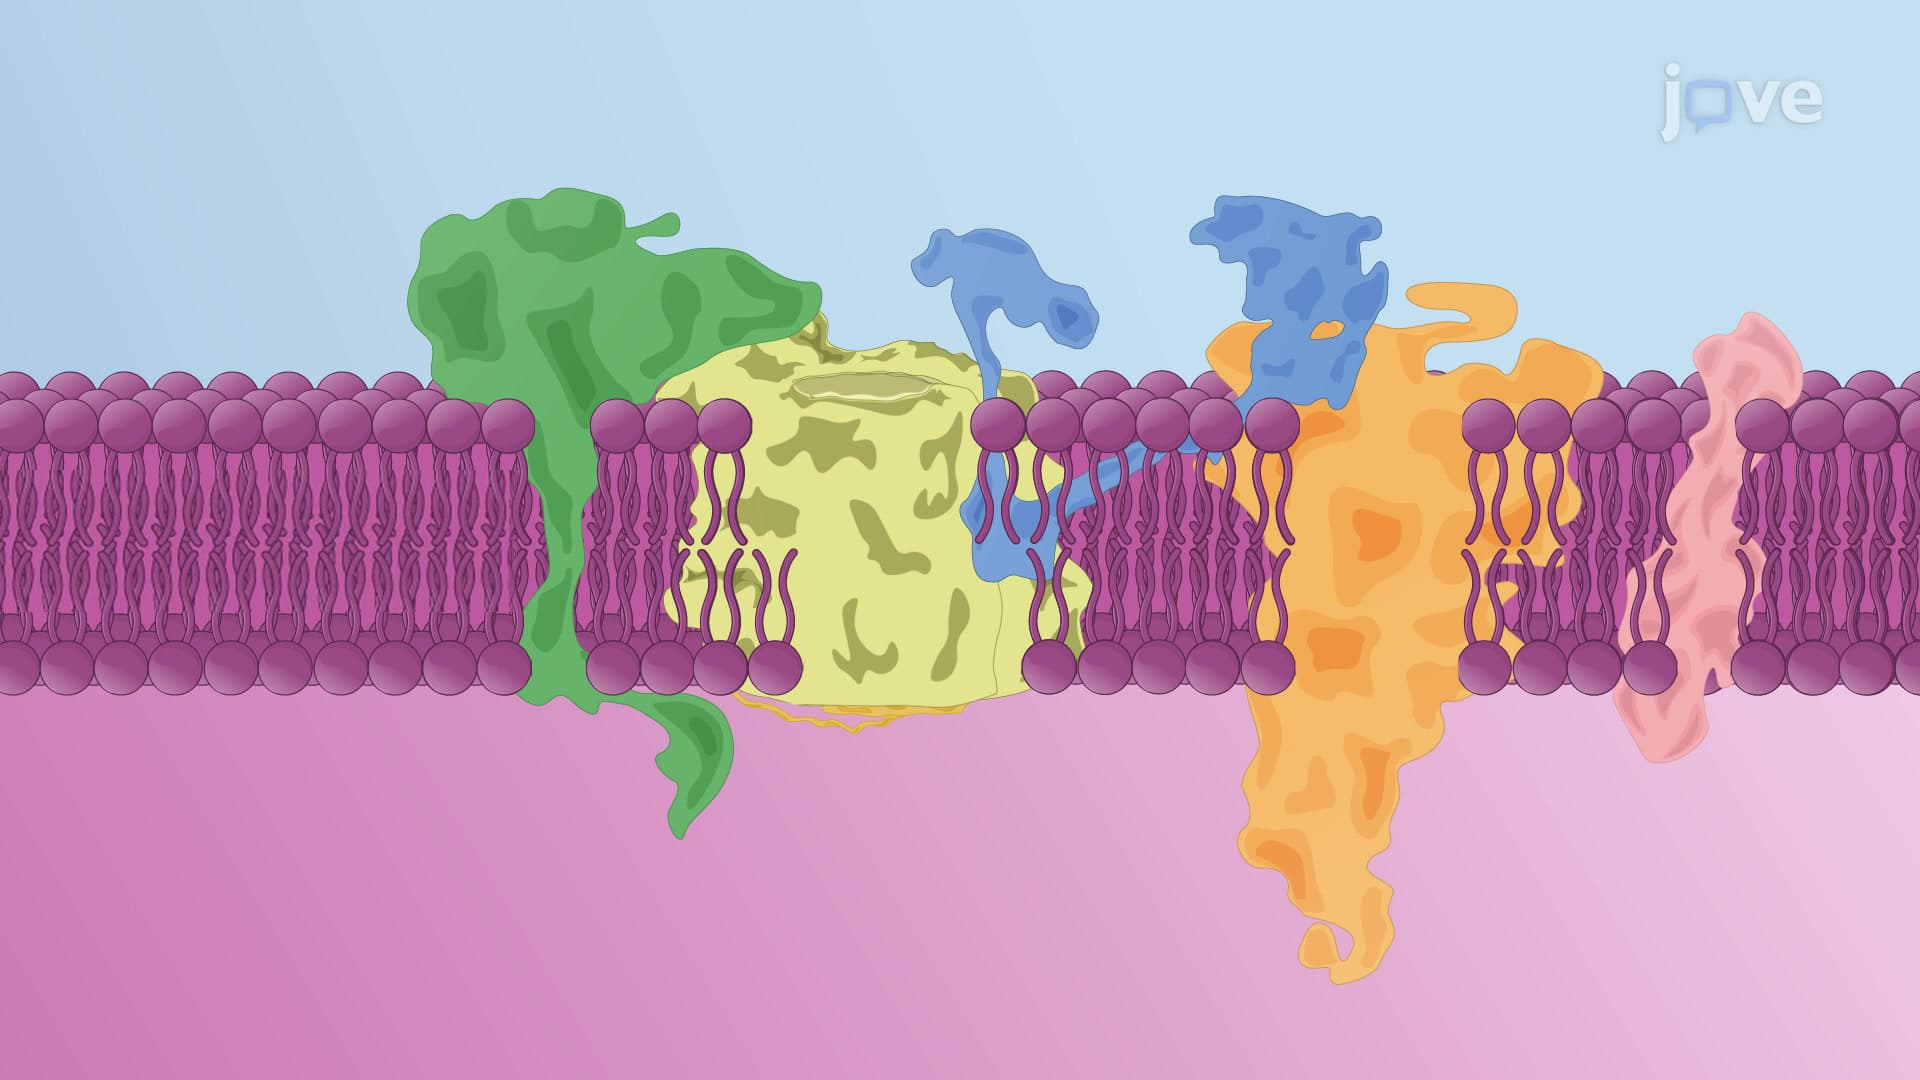 01:28
Protein Translocation Machinery on the ER Membrane
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.