
シナプトタグミン媒介による標的膜の屈曲は,Ca2+) 調節された融合における重要なステップです
Enfu Hui1, Colin P Johnson, Jun Yao
1Howard Hughes Medical Institute, USA.
Cell
|August 26, 2009

まとめ
シナプトタグミン-I (syt) タンパク質媒介の膜屈曲は,エクソサイトーシス中の膜融合を加速するために重要である. この研究は,sytがsytであることを示しています.
科学分野:
- 細胞生物学 細胞生物学
- 膜バイオフィジックス
- 分子神経科学は分子神経科学である.
背景:
- 膀がプラズマ膜と融合する過程であるエクソサイトーシスは,細胞の通信に不可欠です.
- シナプトタグミン-I (syt) がCa2+で誘発される膜曲折における役割と,その融合動力学への貢献は,依然として議論の対象となっている.
- 以前の研究では,前曲線膀または非選択的シート変異体を持つ再構成システムを使用し,膜曲線の直接的な役割に関する結論を制限しました.
研究 の 目的:
- シナプトタグミン-Iの膜曲げ活性が,直接的に標的膜の侵入を駆動して融合を加速するかどうかを調査する.
- sytの核融合促進機能に対する膜曲線の影響を決定する.
主な方法:
- シナプトタグミン-I機能をテストするために,膜の曲線度合いが異なるリポソームを使用しました.
- 管管不全のシナプトタグミンI変異体を使用し,膜曲活動を隔離しました.
- 付加されたN-BARドメインと付加されたN-BARドメインのないSNAREを含むリポソーム間の融合効率の評価.
主要な成果:
- 管管に欠陥があるシナプトタグミンI変異体が,高度に曲線のあるリポソーム間の融合を促進した.
- この変異体は,比較的平らなリポソームで,核融合活性が著しく低下したことを示した.
- 外在的なN-BARドメイン誘発の膜曲折により,平面膜における管路欠陥シナプトタグミンI変異体の融合欠陥が救出されました.
結論:
- シナプトタグミン-Iの膜曲げ能力は,エクソサイトーシス中の効率的な膜融合に不可欠です.
- 局所的な膜屈曲は,単にCa2+結合ではなく,シナプトタグミンIが融合を加速させる重要なメカニズムです.
- この発見は,膜密輸におけるシナプトタグミン-Iの役割の基礎となる生体物理的メカニズムを明確にします.
さらに関連する動画
関連する概念動画
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:43
SNAREs and Membrane Fusion
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:15
Mechanisms of Membrane-bending
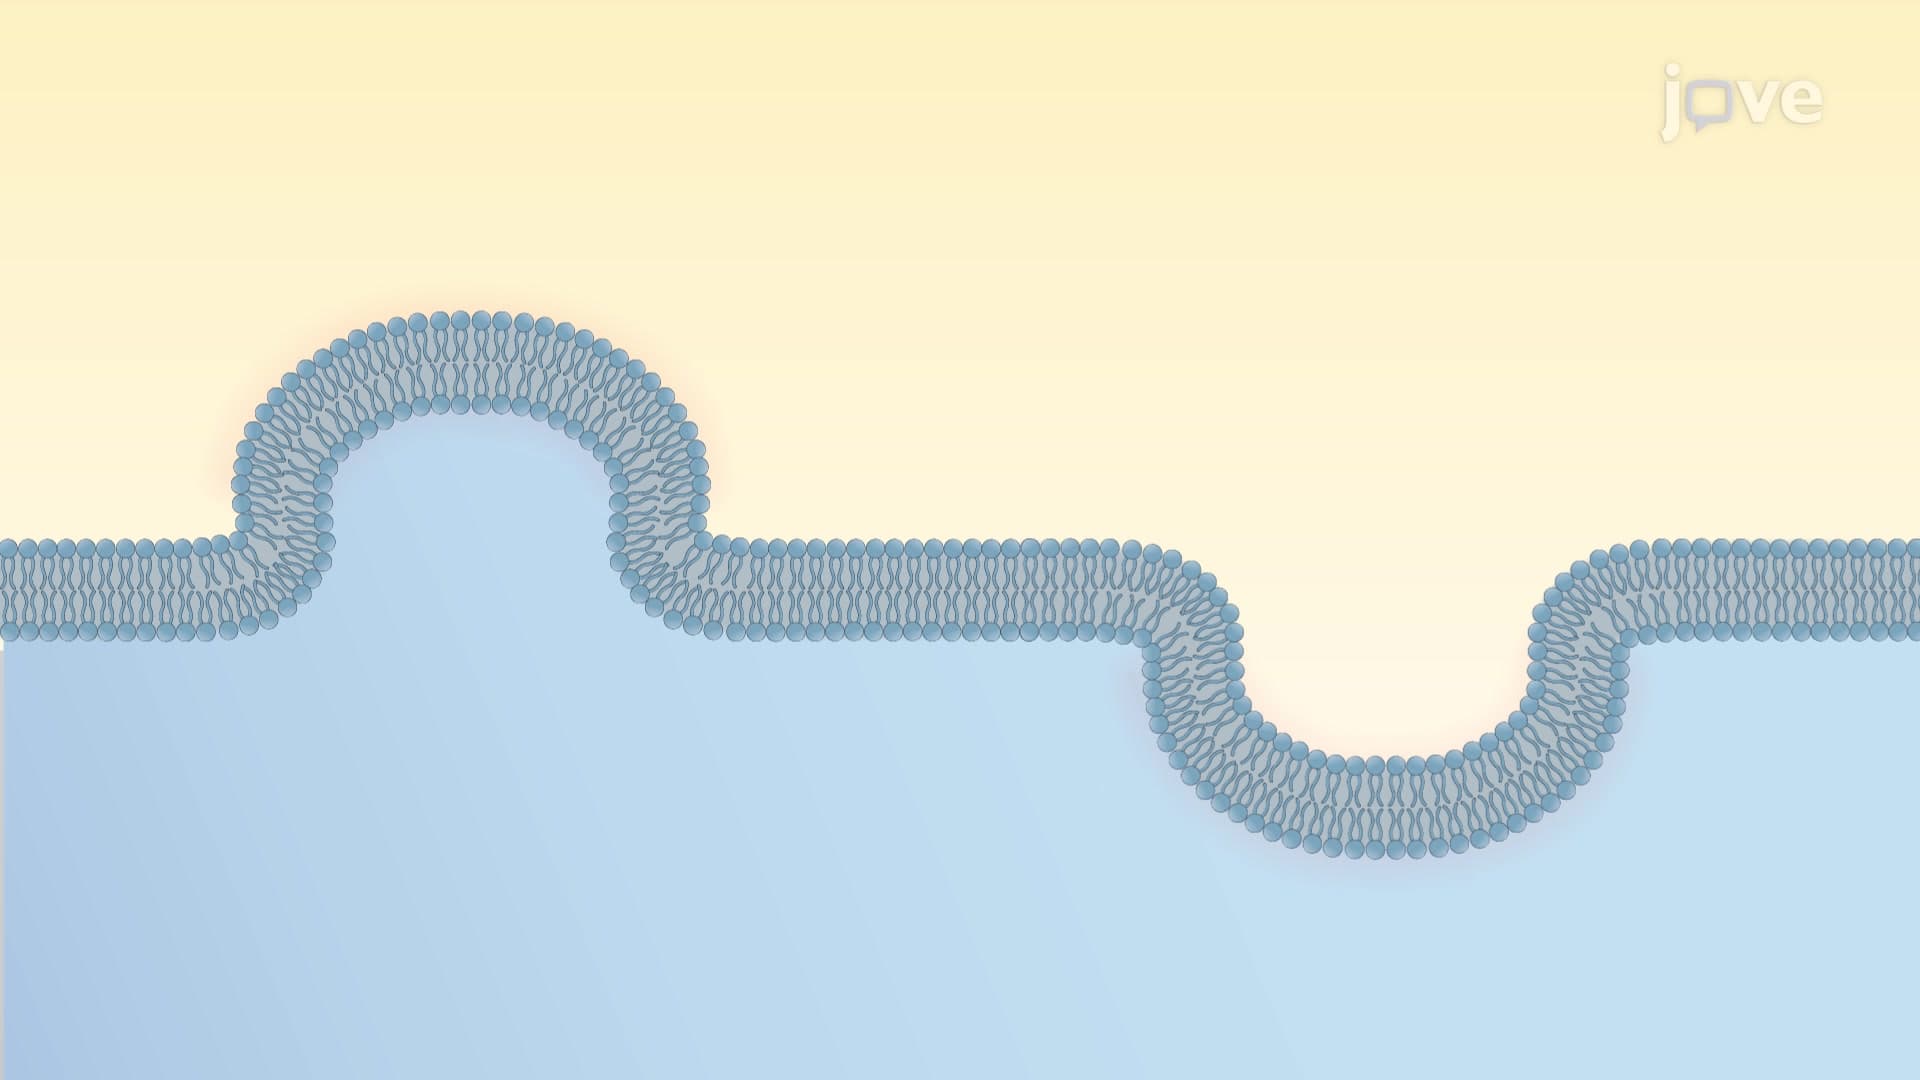
The living membranes are flexible due to their fluid mosaic nature; however, their bending into different shapes is an active process regulated by specific lipids and proteins. The membrane bending can be transient as seen in vesicles or stable for a long time as in microvilli. Cells regulate the size, location, and duration of the membrane curvature.
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:16
Calmodulin-dependent Signaling
Calmodulin (CaM) is a calcium-binding protein in eukaryotes that controls various calcium-regulated cellular processes. It has four calcium-binding sites that bind calcium to form the calcium-calmodulin ( Ca2+-CaM) complex. GPCR stimulation increases the calcium levels in the cells that bind to CaM and induces a conformational change.
The Ca2+-CaM complex does not have enzymatic activity by itself. Instead, the complex binds downstream target proteins, including membrane proteins or enzymes,...
The Ca2+-CaM complex does not have enzymatic activity by itself. Instead, the complex binds downstream target proteins, including membrane proteins or enzymes,...
 01:25
Rab Cascades
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
 01:45
Tail-anchoring of Proteins in the ER Membrane
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...