
光から独立するプロトクロロフィリド還元酵素のX線結晶構造
Norifumi Muraki1, Jiro Nomata, Kozue Ebata
1Department of Life Sciences, University of Tokyo, Komaba, Meguro-ku, Tokyo 153-8902, Japan.
Nature
|April 20, 2010

まとめ
暗闇で作用するプチリド酸化還元酵素 (DPOR) の結晶構造は,クロロフィルの合成のためのメカニズムを明らかにします. この窒素酵素のような酵素は,触媒活性のためにユニークなアスパルテート結合を使用します.
科学分野:
- バイオケミストリー バイオケミストリー
- 構造生物学 構造生物学とは
- 光合成研究 研究 光合成研究
背景:
- 光合成生物は,クロロフィルを光依存性および光依存性Pchlide oxidoreductase (DPOR) の2つの経路で合成する.
- DPORはLタンパク質とNBタンパク質からなる複雑な酵素で,構造的には窒素酵素成分に類似しています.
研究 の 目的:
- Rhodobacter capsulatusからDPORのNBタンパク質の結晶構造を決定する.
- DPORによって触媒化されたプロトクロロフィリド還元のメカニズムを解明する.
主な方法:
- 2.3Åの解像度のX線結晶学.
- 窒素酵素 MoFe タンパク質との構造比較.
主要な成果:
- NB-タンパク質の構造は,窒素酵素MoFeタンパク質に類似しており,BchN-BchBの各ユニットにはプロトクロロフィリドと鉄硫黄群 (NB-群) が含まれています.
- NB-クラスターへのユニークなアスパルテート結合は,クラスター組立だけでなく,触媒活動に不可欠です.
- 特定のプロトクロロフィリドの結合には,アルファヘリクスの解き放たれがあり,トランス固有の還元機構を容易にします.
結論:
- DPORは,安定したマルチボンドを減らすために,窒素酵素と共通のアーキテクチャを共有しています.
- C17=C18の二重結合還元のために,アスパート酸とプロトクロロフィリドC17-プロピオネートを陽子ドナーとして含む新しいメカニズムが提案されています.
- この構造的な洞察は,クロロフィール生物合成と酵素触媒の理解を前進させる.
関連する概念動画
 01:27
Photosystem I
52.8K
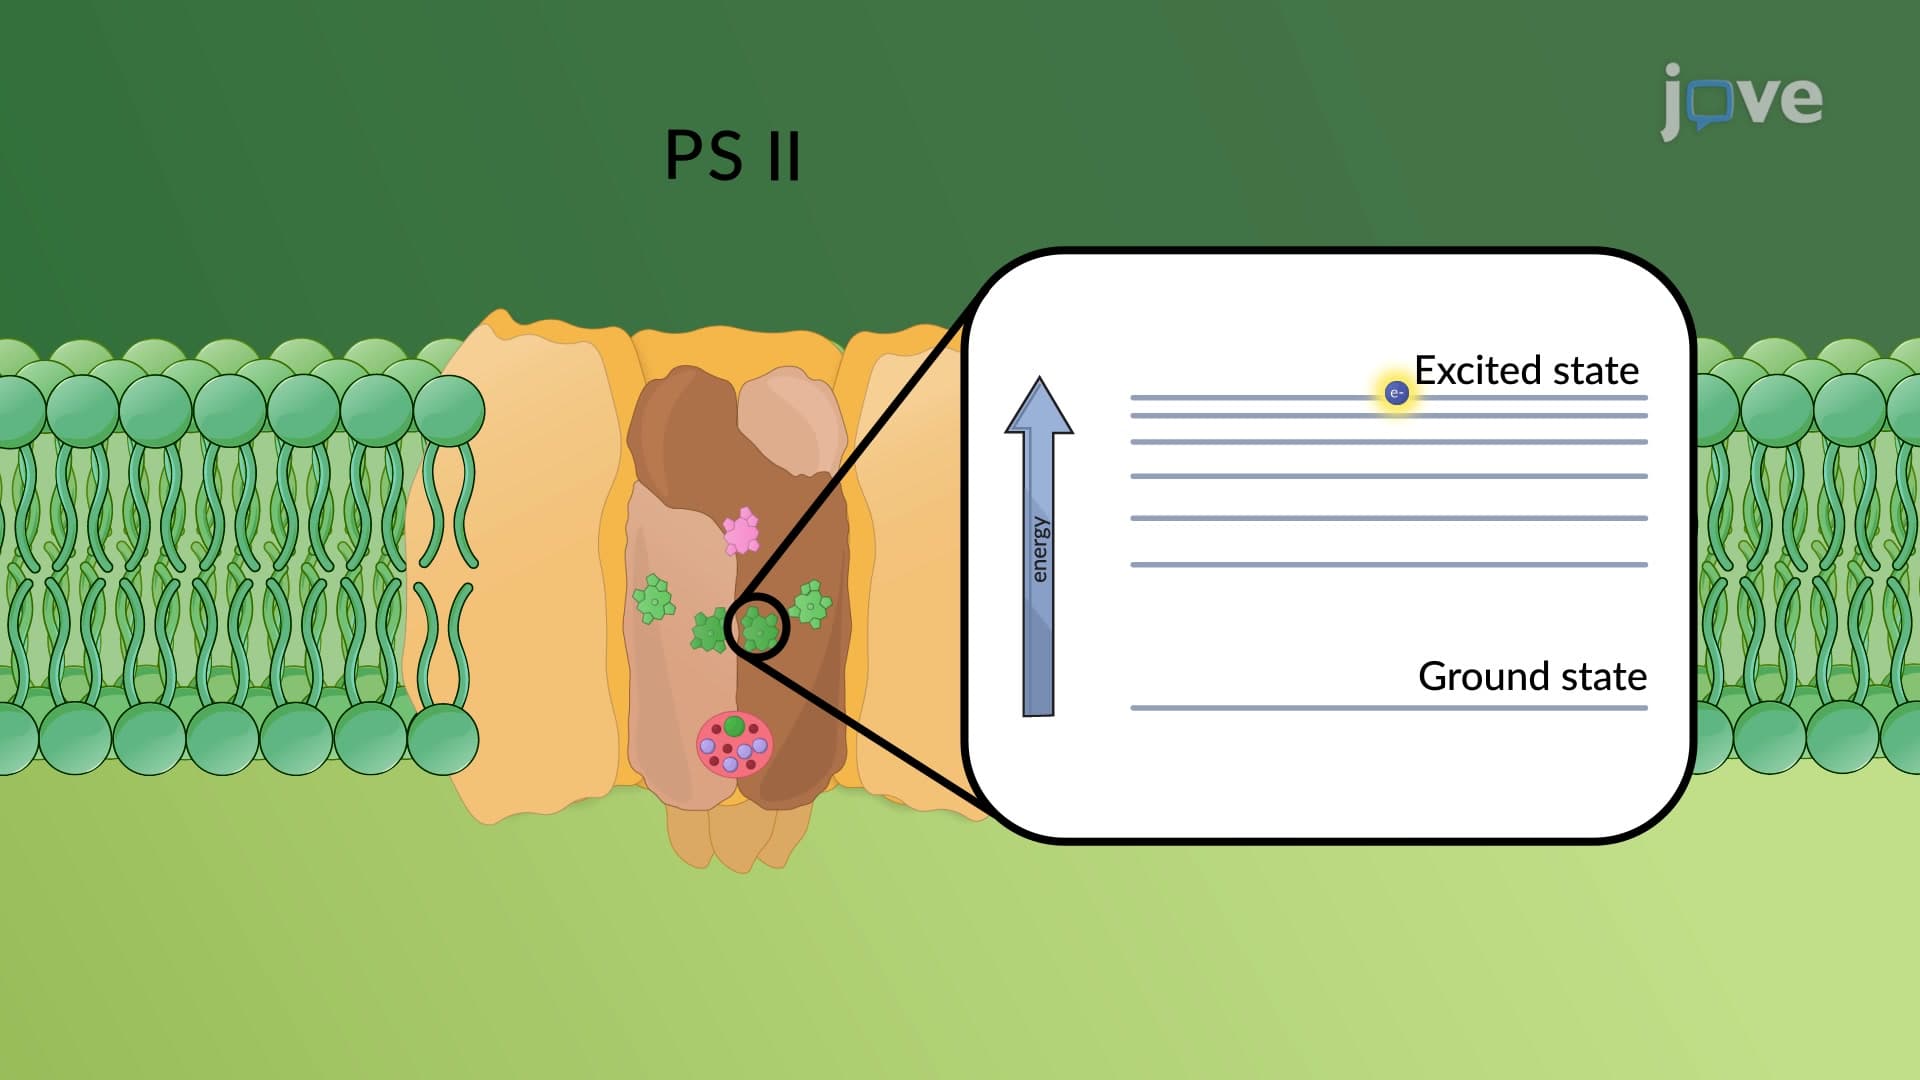
Although structurally similar to photosystem II (PSII), photosystem I (PSI) is has a different electron supplier and electron acceptor.
Both these photosystems work in concert. An excited electron from PSII is relayed to PSI via an electron transport chain in the thylakoid membrane of the chloroplast, which is comprised of the carrier molecule plastoquinone, the dual-protein cytochrome complex, and plastocyanin. As electrons move between PSII and PSI, they lose energy and must be re-energized...
Both these photosystems work in concert. An excited electron from PSII is relayed to PSI via an electron transport chain in the thylakoid membrane of the chloroplast, which is comprised of the carrier molecule plastoquinone, the dual-protein cytochrome complex, and plastocyanin. As electrons move between PSII and PSI, they lose energy and must be re-energized...
52.8K
 01:29
The Photochemical Reaction Center
4.4K
Reaction centers are pigment-protein complexes that initiate energy conversion from photons to chemical entities. Therefore, photochemical reaction center is a more appropriate term that describes these complexes. The Nobel laureates Robert Emerson and William Arnold provided the first experimental evidence of photochemical reaction centers by demonstrating the participation of nearly 2,500 chlorophyll molecules for the release of just one molecule of oxygen. Despite thousands of photosynthetic...
4.4K
 01:15
The Antenna Complex
6.9K
Plants and other photosynthetic organisms comprise pigments capable of absorption of direct sunlight. These pigments are present in the reaction center - the main site of photochemical reactions as well as in the antenna complex. Under average light conditions, the rate at which reaction center pigments absorb light is far below the electron transport chain's capacity. As a result, the reaction center alone cannot provide enough energy to drive photosynthesis. The photosynthetic efficiency can...
6.9K
 01:34
The Z-Scheme of Electron Transport in Photosynthesis
12.6K
The light reactions of photosynthesis assume a linear flow of electrons from water to NADP+. During this process, light energy drives the splitting of water molecules to produce oxygen. However, oxidation of water molecules is a thermodynamically unfavorable reaction and requires a strong oxidizing agent. This is accomplished by the first product of light reactions: oxidized P680 (or P680+), the most powerful oxidizing agent known in biology. The oxidized P680 that acquires an electron from the...
12.6K
 01:11
Channel Rhodopsins
2.5K
Most organisms use photoreceptors to sense and respond to light. Examples of photoreceptors include bacteriorhodopsins and bacteriophytochromes in some bacteria, phytochromes in plants, and rhodopsins in the photoreceptor cells of the vertebral retina. The light-sensitive property of these receptors is because of the bound chromophores, such as bilin in the phytochromes and retinal in the rhodopsins.
Rhodopsins belong to the family of cell surface proteins called G-protein coupled receptors,...
Rhodopsins belong to the family of cell surface proteins called G-protein coupled receptors,...
2.5K
 01:43
Electron Transport Chain: Complex III and IV
6.7K
During the electron transport chain, electrons from NADH and FADH2 are first transferred to complexes I and II, respectively. These two complexes then transfer the electrons to ubiquinol, which carries them further to complex III. Complex III passes the electrons across the intermembrane space to Cyt c, which carries them further to complex IV. Complex IV donates electrons to oxygen and reduces it to water. As electrons pass through complexes I, III, and IV, the energy released aids the pumping...
6.7K