
MDCK細胞からのアピカル・ベソラテラル・エンドサイト・ベシクル間の微小管およびモーター依存融合をインビトロで行う
M Bomsel1, R Parton, S A Kuznetsov
1European Molecular Biology Laboratory, Heidelberg, Federal Republic of Germany.
Cell
|August 24, 1990

まとめ
細胞内分泌の経路は,末期のエンドソームで結合する. in vitroで再構成されたこのプロセスは,小胞融合のためにマイクロチューブルとキネシンやダイネインのようなモータータンパク質を必要とします.
科学分野:
- 細胞生物学 細胞生物学
- 分子生物学は分子生物学である.
- エピテル細胞生物学 エピテル細胞生物学
背景:
- 皮質細胞は,異なるアピカルとベースラテラルエンドサイトーシス経路を利用します.
- これらの経路は,細胞内の末端エンドソームに収束することが知られている.
- この収束を理解することは,細胞の取引と機能にとって極めて重要です.
研究 の 目的:
- 末期エンドソームとアピカルおよびベースラテラル内細胞小胞の in vitro 融合を復元し,分析する.
- 細胞のないシステムにおける内細胞経路の収束のための分子要件を特定する.
- この過程における微小管および関連するタンパク質の役割を調査する.
主な方法:
- 後期エンドソームとの膀融合を測定するための細胞フリーアッセイの開発.
- マディン・ダービー犬腎臓 (MDCK) 細胞を用いて,上皮内分細胞を研究する.
- 微小管に依存するタンパク質の必要性の生化学的分析.
主要な成果:
- 末期エンドソームによる内細胞胞融合の in vitro 再構成は成功しました.
- ポリマー化されたマイクロチューブルは,この in vitro 融合プロセスに不可欠であることが判明しました.
- キネシンやサイトプラズミックダイネインを含むマイクロチューブル結合タンパク質は,重要な成分として特定されました.
結論:
- 頂点と底辺のエンドサイトーシス経路の収束は,微小管に依存するメカニズムに依存しています.
- 機械化学モーターであるキネシンとダイネインは,末期エンドソームの膀融合を媒介する重要な役割を果たします.
- この細胞のないシステムは,内細胞経路収束の分子機構を解剖するための貴重なツールを提供します.
関連する概念動画
 01:38
Intralumenal Vesicles and Multivesicular Bodies
3.9K
Intraluminal vesicles (ILVs) are small vesicles 50-80 nm in diameter formed during the maturation of early endosomes. A specialized endosome containing numerous ILVs is called a multivesicular body (MVB). ILVs contain internalized molecules such as antigens, nucleic acids, proteins, and metabolites. Some of these molecules are released from the MVBs inside exosomes and are transported to other cells. Other MVBs contain molecules that are retained in the ILVs and are later degraded within the...
3.9K
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
15.8K
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
15.8K
 01:32
Microtubule Associated Motor Proteins
9.9K
Eukaryotic cells have different motor proteins for transporting various cargo within the cell. These motor proteins differ based on the filament they associate with, the direction they move within the cell, and the type of cargo they transport. Motor proteins that associate with microtubules are known as microtubule-associated motor proteins. There are two families of microtubule-associated motor proteins —Kinesins and Dyneins. Both these proteins assist in the transport of cellular...
9.9K
 01:43
The Movement of Organelles and Vesicles
5.3K
In eukaryotic cells, cytoskeletal filaments such as actin, microtubules, and intermediate filaments form a mesh-like cytoskeletal network. These filaments serve as tracks for transporting cellular cargo. Specialized motor proteins use the chemical energy stored in adenosine triphosphate (ATP) for this transport. During interphase, microtubules are polarized, with the plus-end towards the cell periphery and the minus-end towards the cell center. Two microtubule-associated motor proteins,...
5.3K
 01:45
Vesicular Tubular Clusters
2.4K
After budding out from the ER membrane, some COPII vesicles lose their coat and fuse with one another to form larger vesicles and interconnected tubules called vesicular tubular clusters or VTCs. These clusters constitute a compartment at the ER-Golgi interface known as ERGIC (Endoplasmic Reticulum Golgi Intermediate Compartment). The ERGIC is a mobile membrane-bound cargo transport system that sorts proteins secreted from ER and delivers them to the Golgi.
With the help of motor proteins such...
With the help of motor proteins such...
2.4K
 01:39
Anaphase A and B
4.3K
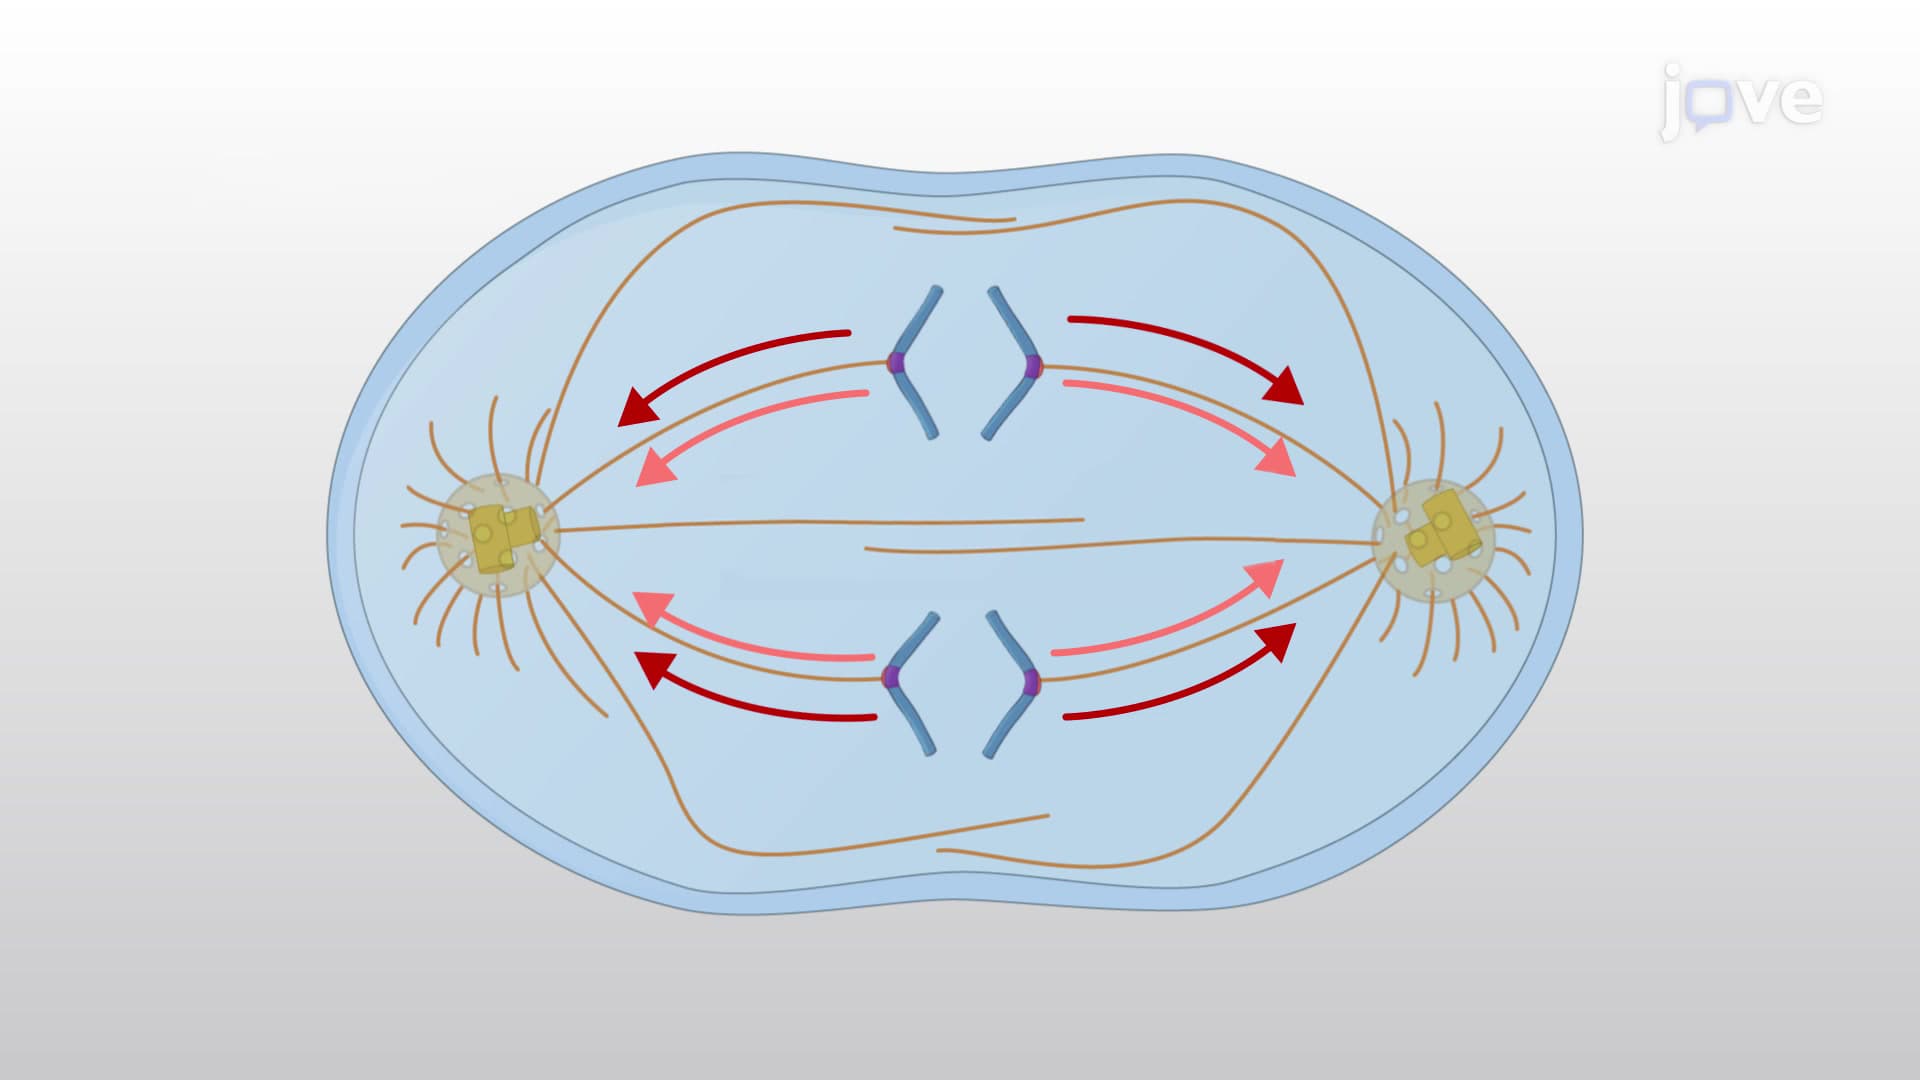
Microtubules form through the end-to-end polymerization of tubulin heterodimers. Kinetochore microtubules originate from the spindle poles, and their plus-ends connect with the kinetochores on sister-chromatids. Ndc80 protein complexes, present on the kinetochore, form low-affinity links with the plus end of these kinetochore microtubules.
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
4.3K