カーディオリピンに結合したシトクロームCの構造的異質性の起源
Yuning Hong1, Julia Muenzner, Sebastian K Grimm
1Department of Chemistry, Dartmouth College, Hanover, New Hampshire 03755, United States.
Journal of the American Chemical Society
|October 17, 2012

まとめ
サイトクロームc (cytc) がカルディオリピン (CL) に結合すると,部分的な展開が誘発され,その過酸化酵素の機能が活性化されます. 2つの異なるCL-bound cytokine形状,拡張型とコンパクト型が均衡状態にあり,アポトーシスの実行に影響を与えます.
科学分野:
- バイオケミストリー バイオケミストリー
- 分子生物学は分子生物学である.
- 細胞生物学 細胞生物学
背景:
- サイトクロームc (cyt c) はアポトーシスにおいて重要な役割を果たします.
- カーディオリピン (CL) との相互作用は,アポトーシスの重要なイベントであるcyt cの過酸化作用を誘発する.
- アセンブル平均化方法は,異質なタンパク質構成の理解を制限する.
研究 の 目的:
- カーディオリピン (CL) 結合時のシトクロームc (cytc) の構造的動態を特徴づける.
- 異なる細胞構造の間の機能的分割を解明する.
- 静電相互作用と結合メカニズムが細胞構造の変化における役割を理解する.
主な方法:
- 時間分解のフォースター共鳴エネルギー伝送 (TR-FRET) で,距離分布を分析する.
- 光相関スペクトロスコーピー (FCS) は,分子動力学を研究するためのものです.
- バイオレイヤインターフェロメトリーで,結合運動とコンフォーマーション交換を評価する.
主要な成果:
- 2つの異なるCL結合型細胞構造を特定した:拡張型とコンパクト型.
- これらのサブ集団間のサブミリ秒コンフォメーション交換が実証されています.
- CLとの静電相互作用が,細胞結合と適合運動力学に著しく影響することを示した.
- 深層膜挿入ではなく,周辺結合機構を示した.
結論:
- カーディオリピンの結合は,サイトクロームcの部分的な展開と機能的活性化を誘導する.
- CL-bound cytcの2つの異なる相互変換構成が存在し,そのアポプトティックな役割に影響を与えています.
- 脂質表面への周辺結合は,細胞の展開と過酸化酵素の活性化を説明し,タンパク質の折り畳みダイナミクスに関する洞察を提供します.
関連する概念動画
 01:35
Asymmetric Lipid Bilayer
Biological membranes show uneven distribution of different types of lipids in the inner and outer layers, resulting in transverse asymmetric membranes. The treatment of the erythrocyte membrane with the enzyme phospholipase confirmed the asymmetric nature of the lipid bilayer. The enzyme hydrolyzes lipids into fatty acids and hydrophilic groups. The phospholipase acts only on the outer layer of the membrane, while the inner layer remains intact. The phospholipase treatment resulted in 80%...
 01:28
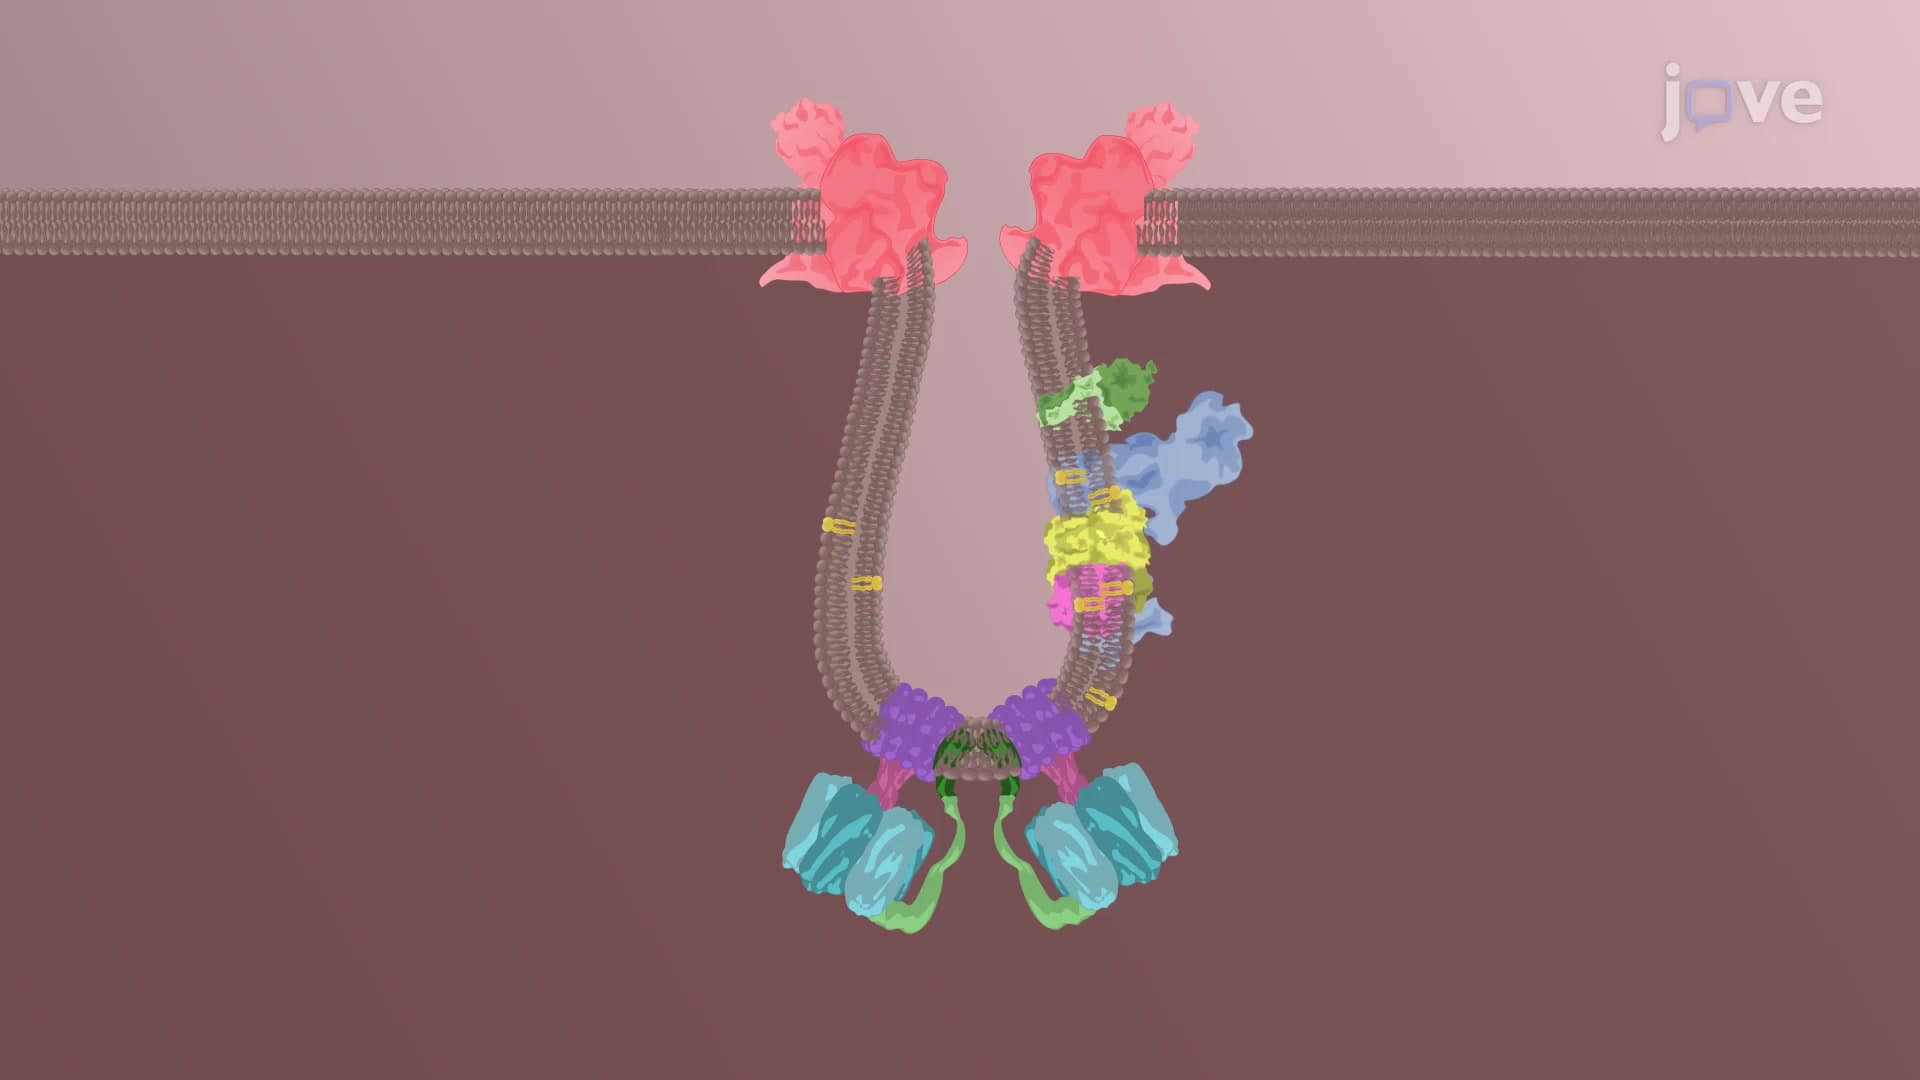
The Inner Mitochondrial Membrane
The inner mitochondrial membrane is the primary site of ATP synthesis. The inner membrane domain that forms a smooth layer adjacent to the outer membrane is called the inner boundary membrane. This domain contains membrane transporters that drive metabolites in and out of the mitochondria. In contrast, the inner membrane network that invaginates into the matrix space is called the cristae membrane. This domain accounts for principle mitochondrial function as it accommodates the protein...
 01:41
The Supercomplexes in the Crista Membrane
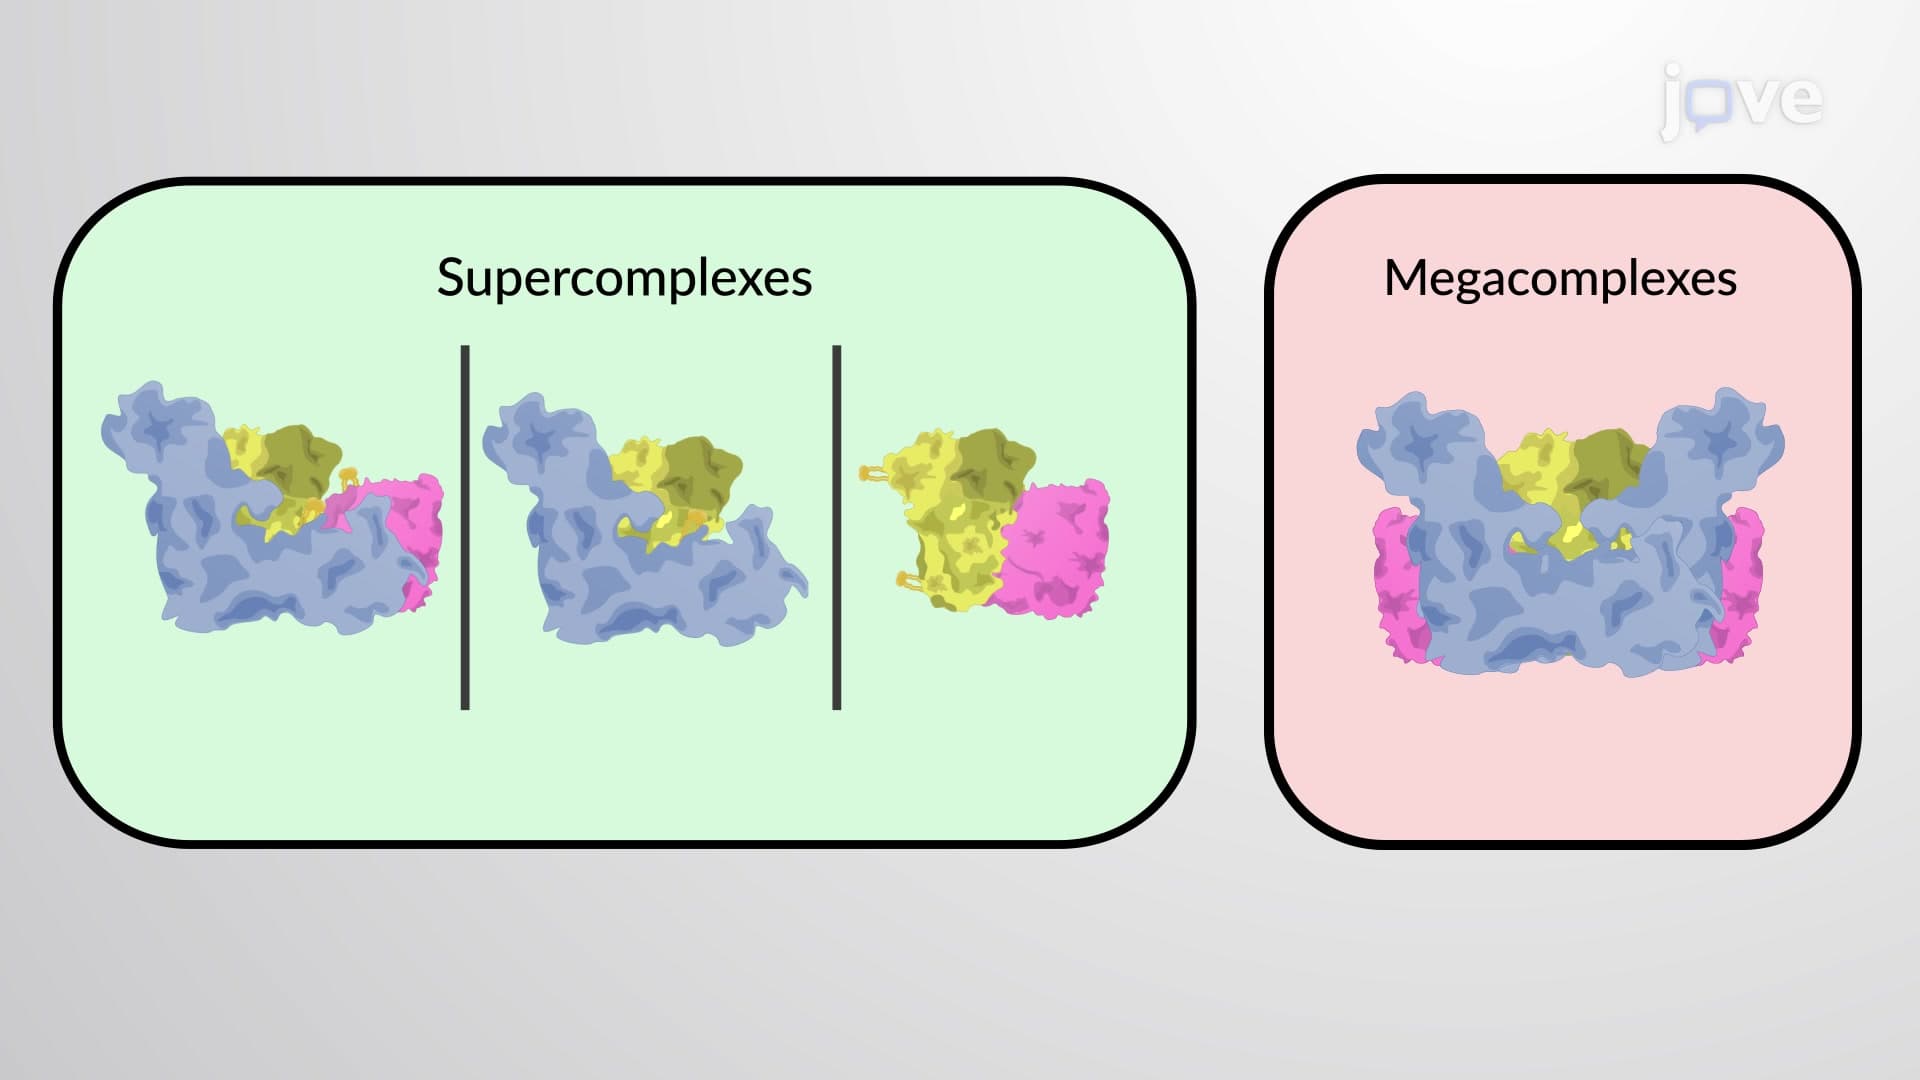
The mitochondrial cristae membrane is the primary site for the oxidative phosphorylation (OXPHOS) process of energy conversion mediated through respiratory complexes I to V. These complexes have been widely studied for decades, and it has been proven that they form supramolecular structures called respiratory supercomplexes (SC). These higher-order complexes may be crucial in maintaining the biochemical structure and improving the physiological activity of the individual complexes while...
 01:43
Electron Transport Chain: Complex III and IV
During the electron transport chain, electrons from NADH and FADH2 are first transferred to complexes I and II, respectively. These two complexes then transfer the electrons to ubiquinol, which carries them further to complex III. Complex III passes the electrons across the intermembrane space to Cyt c, which carries them further to complex IV. Complex IV donates electrons to oxygen and reduces it to water. As electrons pass through complexes I, III, and IV, the energy released aids the pumping...
 01:26
Transport Across the Golgi
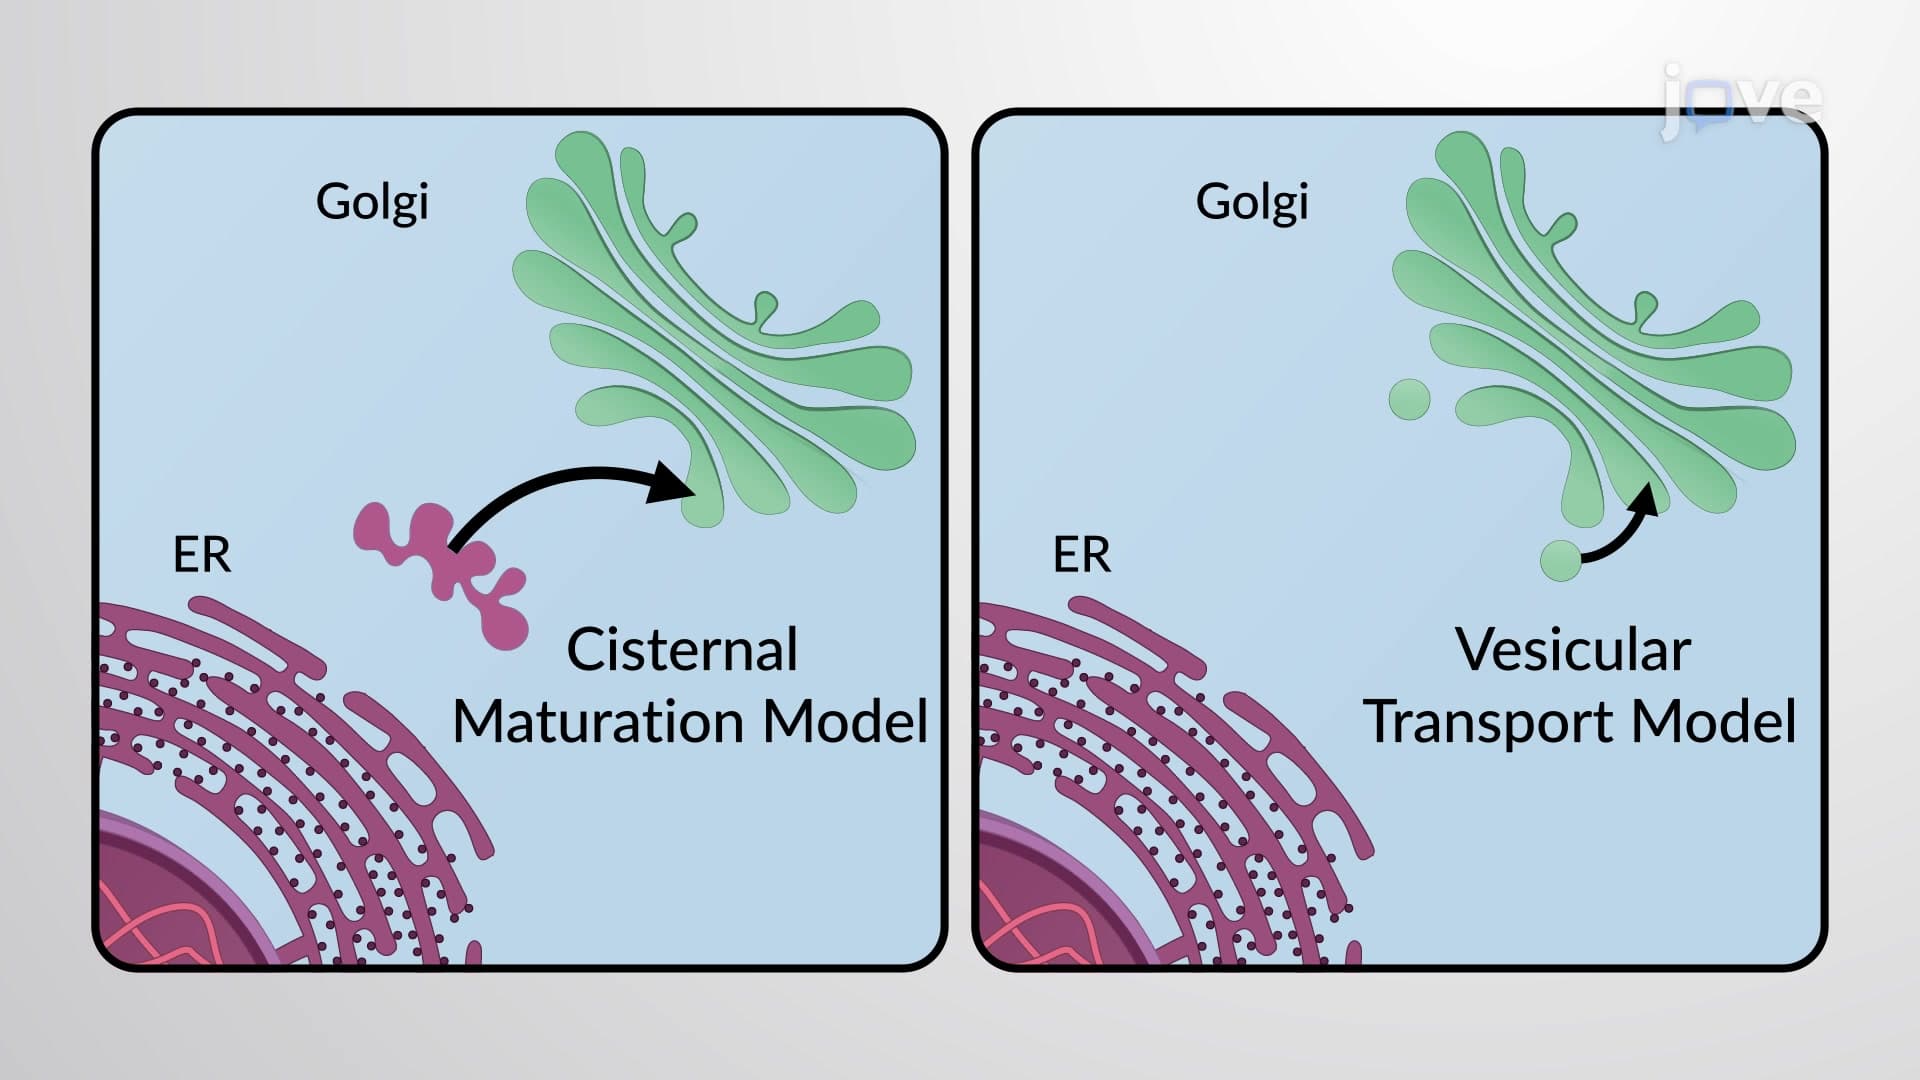
While it is unclear how molecules move between adjacent Golgi cisternae, it is apparent that the molecules move from cis- cisterna, the entry face, to the trans- cisterna, the exit face. Experiments initially suggested vesicles that bud from one cisterna and fuse with the next cisterna to transport proteins between the cisternae. This vesicular transport model describes the Golgi apparatus as a relatively static structure with a unique enzyme composition in each cisterna. Molecules are...
 01:28
Assembly of the Lipid Bilayer in the ER
Biological membranes are more than just a barrier separating cell cytoplasm from the outside environment. They are highly dynamic and help maintain the integrity and physiological stability of the cells as well as membrane-bound organelles. Membranes also play vital roles in cell-to-cell and intracellular communication.
A large chunk of any biological membrane is composed of phospholipids. These lipids have a heterogeneous distribution across different subcellular organelles and even between...
A large chunk of any biological membrane is composed of phospholipids. These lipids have a heterogeneous distribution across different subcellular organelles and even between...