
統合膜の結晶構造であるダイアシルグリセロールキナーゼは,
Dianfan Li1, Joseph A Lyons, Valerie E Pye
1School of Biochemistry and Immunology & School of Medicine, Trinity College Dublin, Dublin 2, Ireland.
Nature
|May 17, 2013

まとめ
膜酵素のモデルであるダイアシルグリセロールキナーゼは,構造的に特徴づけられました. 結晶構造は,そのホモトリメア形と活性部位を明らかにし,以前のモデルとは異なる.
科学分野:
- バイオケミストリー バイオケミストリー
- 構造生物学 構造生物学とは
- 膜タンパク質酵素学 膜タンパク質酵素学
背景:
- ダイアシルグリセロールキナーゼ (DGK) は,グラム陰性細菌の細胞包膜合成に不可欠であり,ダイアシルグリセロールのリン酸化をリン酸酸酸性酸に触媒する.
- この121の残留酵素は,膜タンパク質の酵素学,折り畳み,組み立て,安定性を研究するための長年のモデルです.
研究 の 目的:
- ダイアシルグリセロールキナーゼの3つの機能形態の高解像度結晶構造を提示する.
- 酵素のホモトリミラー構造,活性部位,および基板/共因子結合の解明.
主な方法:
- X線結晶学を用いて,野生型および変異性ダイアシルグリセロールキナーゼの構造を決定した.
- 構造分析は,活性部位,トランスメブランドメイン,オリゴメリック状態を特定することに焦点を当てました.
主要な成果:
- 3つの結晶構造はホモトリメア型ダイアシルグリセロールキナーゼを明らかにし,各モノメアは3つのトランスメブランヘリックスとN端のアンフィパシーヘリックスを有する.
- 構造は,結合された脂質基質とドッキングされたATPと共有された複合活性部位を識別します.
- これらの結晶構造は,ドメイン交換に関する公開されたソリューションNMRモデルと矛盾しています.
結論:
- 結晶構造は,ダイアシルグリセロールキナーゼの機能とメカニズムを理解するための詳細な分子基礎を提供します.
- この発見は,このモデル酵素に関する広範な既存の生化学および生理学的データを合理化します.
- 観測された構造は,以前のソリューション状態モデルと矛盾しており,構造的文脈の重要性を強調しています.
関連する概念動画
 01:11
IP3/DAG Signaling Pathway
Membrane lipids such as phosphatidylinositol (PI) are precursors for several membrane-bound and soluble second messengers. Specific kinases phosphorylate PI and produce phosphorylated inositol phospholipids. One such inositol phospholipids are the phosphatidylinositol-4,5 bisphosphate [PI(4,5)P2], present in the inner half of the lipid bilayer. Upon ligand binding, GPCR stimulates Gq proteins to turn on phospholipase Cꞵ. Activated phospholipase Cꞵ cleaves PI(4,5)P2 and produces two-second...
 01:22
Activation and Inactivation of G Proteins
Heterotrimeric G proteins are guanine nucleotide-binding proteins. As the name suggests, heterotrimeric G proteins are composed of three subunits: alpha, beta, and gamma. They remain GDP-bound or GTP-bound inside the cells and switch between inactive/active states. The Gα subunit possesses the nucleotide-binding pocket that binds guanine nucleotides and switches between GDP or GTP-bound states. In contrast, the Gꞵ and Gγ subunits are always bound together with high affinity and are together...
 01:32
Pinching-off of Coated Vesicles
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
 01:32
Lipids as Anchors
In the plasma membrane, the lipids forming the bilayer can also act as an anchor to tether proteins to the membrane. The three main types of lipid anchors found in eukaryotes are – prenyl groups, fatty acyl groups, and glycosylphosphatidylinositol or GPI groups. Prenyl and fatty acyl groups act as anchors on the cytosolic surface of the membrane, whereas GPI anchors proteins on the extracellular side.
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains the...
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains the...
 01:30
Assembly of Signaling Complexes
Multiprotein signaling complexes are formed in a dynamic process involving protein-protein interactions at the cytoplasmic domain of transmembrane receptors or enzymatic and non-enzymatic proteins associated with the receptor. These complexes ensure the activation and propagation of intracellular signals that regulate cell functions.
Interaction domains in cell signaling
Interaction domains recognize exposed features of their binding partners containing post-translationally modified sequences,...
Interaction domains in cell signaling
Interaction domains recognize exposed features of their binding partners containing post-translationally modified sequences,...
 01:18
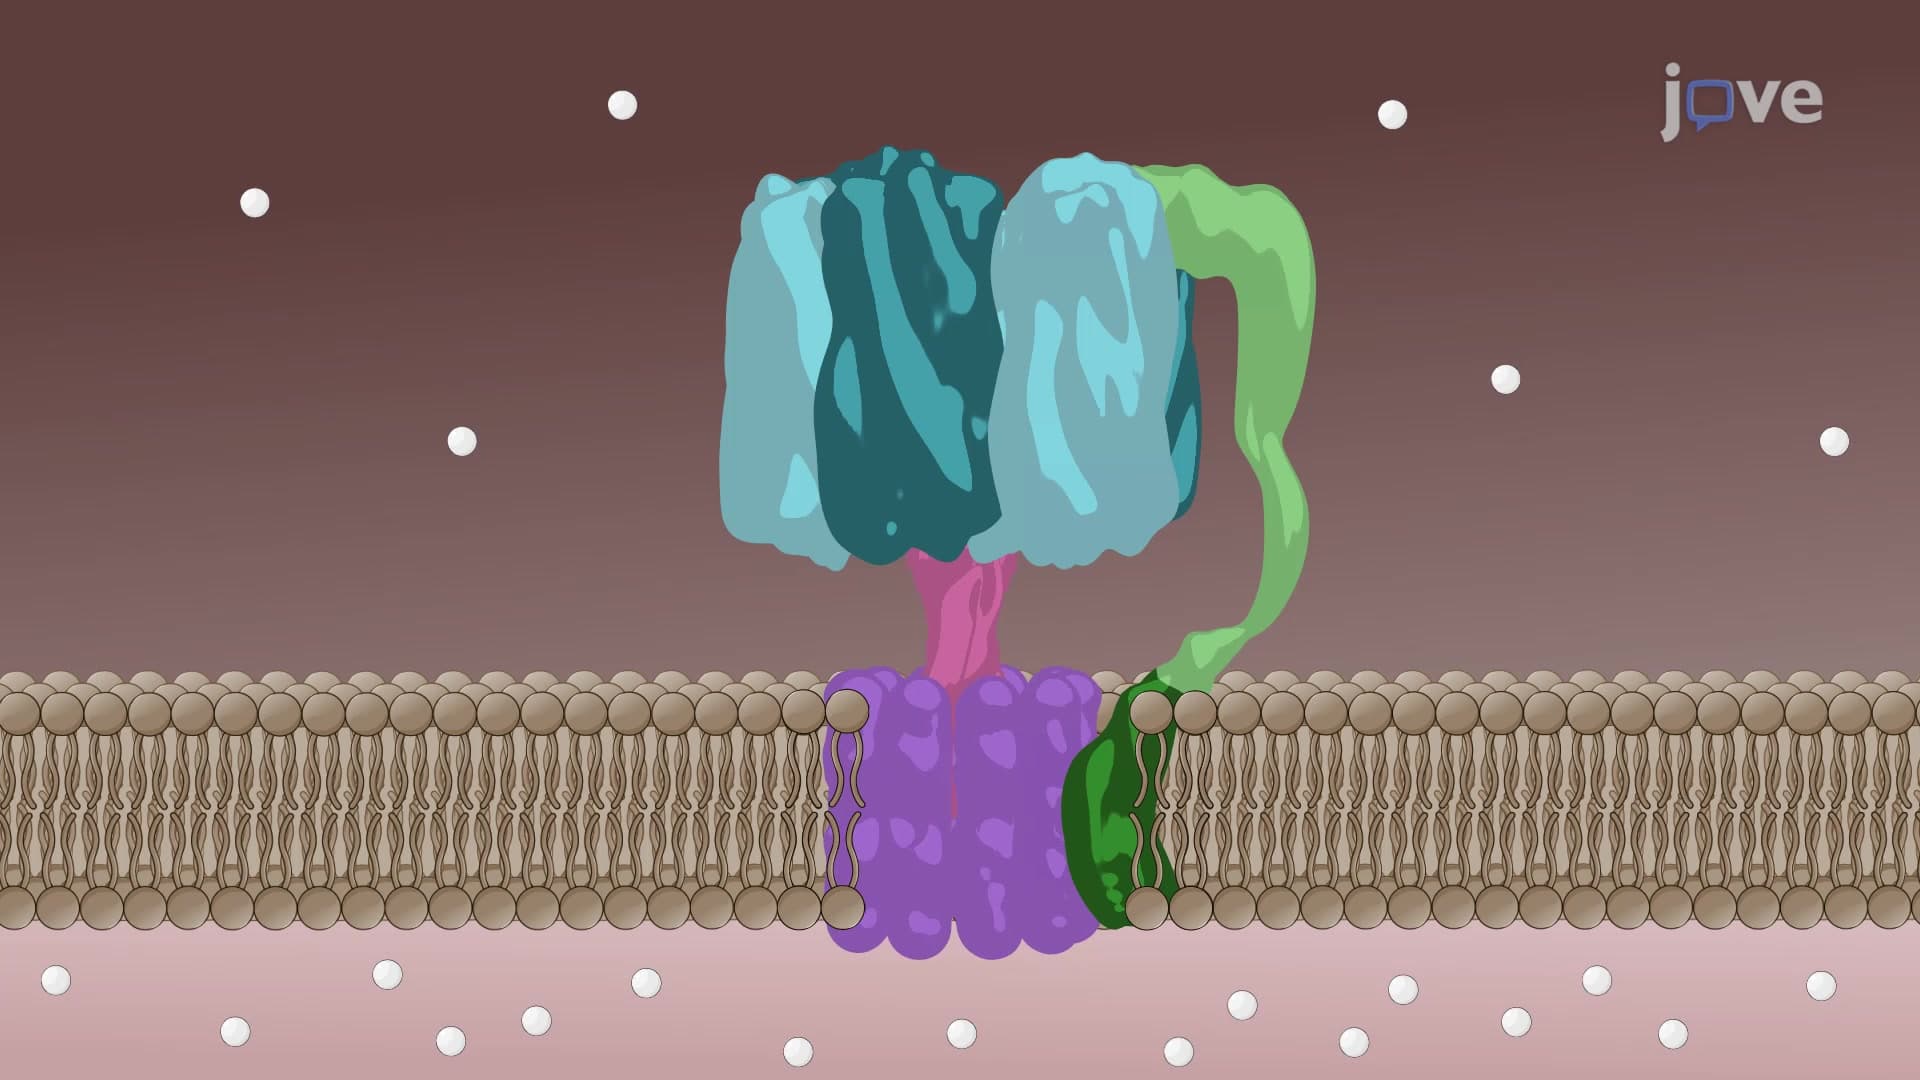
ATP Synthase: Structure
ATP synthase or ATPase is among the most conserved proteins found in bacteria, mammals, and plants. This enzyme can catalyze a forward reaction in response to the electrochemical gradient, producing ATP from ADP and inorganic phosphate. ATP synthase can also work in a reverse direction by hydrolyzing ATP and generating an electrochemical gradient. Different forms of ATP synthases have evolved special features to meet the specific demands of the cell. Based on their specific feature, ATP...