
精製した成分で管状エンドプラズマ網の復元
Robert E Powers1,2, Songyu Wang1,2, Tina Y Liu1,2
1Howard Hughes Medical Institute, Harvard Medical School, 240 Longwood Avenue, Boston, Massachusetts 02115, USA.
Nature
|February 23, 2017

まとめ
細胞の臓器の形状は タンパク質の小さなセットによって維持されます このダイナミックな管状ネットワークには,連続した膜融合とエネルギー依存の安定状態プロセスが必要です.
科学分野:
- 細胞生物学
- 分子生物学
- バイオ物理学
背景:
- 臓器細胞の形状は細胞の機能に不可欠ですが,臓器細胞の形成のメカニズムはほとんど不明です.
- エンドプラズマ網 (ER) は,形成が完全に理解されていない複雑でダイナミックな管状のネットワークを特徴としています.
- いくつかの膜タンパク質がERネットワーク形成に関与しているが,その正確な役割と必要性は不明である.
研究 の 目的:
- エンドプラズマ網管網の形成と維持の基礎となる分子機構を調査する.
- Sey1p と Yop1p のような特定の膜タンパク質が ER 構造を形作る役割を決定する.
- 精製したタンパク質を使って ERネットワークの形成を再構成し,分析する.
主な方法:
- プロテオリポソームで精製されたエンドプラズマ網膜タンパク質 (Sey1pとYop1p) を使用してダイナミックな管状膜ネットワークを再構成する.
- ネットワーク形成を開始するためにGTP添加を使用し,ネットワーク維持を研究するためにGTP水解を阻害します.
- Sey1pの他の曲線安定化タンパク質 (レチクロン,REEPs) とその脊椎動物のオートログであるAtlastinとの相互作用を試験する.
主要な成果:
- セイ1p (膜融合GTPase) とYop1p (曲線安定タンパク質) を含むプロテオリポソームは,GTPを添加するとチューブ状のネットワークを形成する.
- Sey1pのGTP水解の阻害は迅速な管の断片化をもたらし,継続的な膜融合の必要性を示した.
- Sey1pは様々な曲線安定化タンパク質とネットワークを形成し,Atlastinは独立してGTP水解に依存するネットワークを形成しました.
結論:
- 臓器細胞の形,特にER管状のネットワークは,最小限のタンパク質で生成できます.
- ネットワークのメンテナンスはエネルギーに依存するプロセスで,膜融合と分解の間の安定状態を表します.
- Sey1pとAtlastinは,ERネットワークの構造とダイナミクスの重要なレギュレータとして機能します.
関連する概念動画
 01:43
The Endoplasmic Reticulum
22.4K
The endoplasmic reticulum or ER makes up for more than half of the membranes in a cell and accounts for 10% of total cell volume. It is also the primary protein and lipid synthesis factory for most cell organelles, such as the Golgi apparatus, lysosomes, secretory vesicles, and the plasma membrane. Despite being the most extensive and functionally complex subcellular organelle, ER was the last to be discovered. After years of deliberation, Keith Porter and George Palade in the year 1954,...
22.4K
 01:39
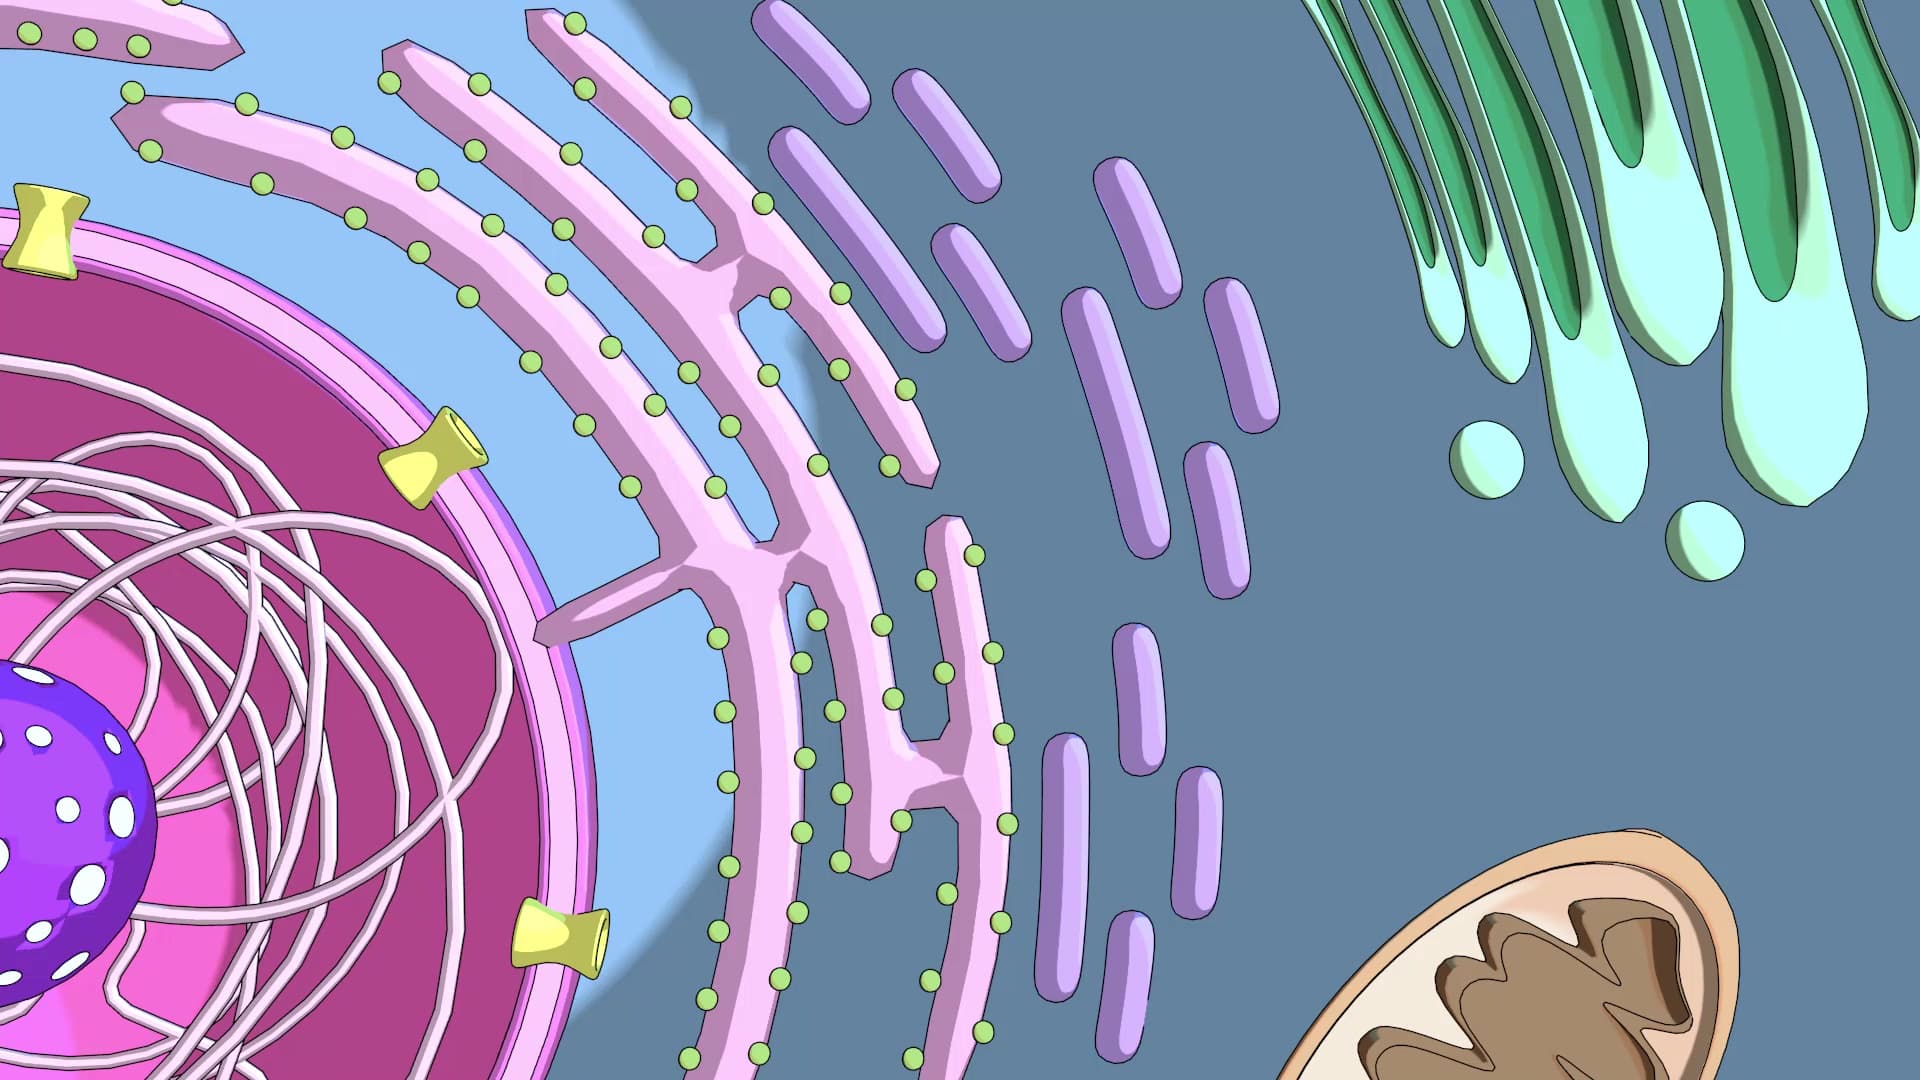
Endoplasmic Reticulum
116.3K
The Endoplasmic Reticulum (ER) in eukaryotic cells is a substantial network of interconnected membranes with diverse functions, from calcium storage to biomolecule synthesis. A primary component of the endomembrane system, the ER manufactures phospholipids critical for membrane function throughout the cell. Additionally, the two distinct regions of the ER specialize in the manufacture of specific lipids and proteins.
116.3K
 01:32
Export of Misfolded Proteins out of the ER
5.4K
After folding, the ER assesses the quality of secretory and membrane proteins. The correctly folded proteins are cleared by the calnexin cycle for transport to their final destination, while misfolded proteins are held back in the ER lumen. The ER chaperones attempt to unfold and refold the misfolded proteins but sometimes fail to achieve the correct native conformation. Such terminally misfolded proteins are then exported to the cytosol by ER-associated degradation or ERAD pathway for...
5.4K
 01:45
Vesicular Tubular Clusters
3.3K
After budding out from the ER membrane, some COPII vesicles lose their coat and fuse with one another to form larger vesicles and interconnected tubules called vesicular tubular clusters or VTCs. These clusters constitute a compartment at the ER-Golgi interface known as ERGIC (Endoplasmic Reticulum Golgi Intermediate Compartment). The ERGIC is a mobile membrane-bound cargo transport system that sorts proteins secreted from ER and delivers them to the Golgi.
With the help of motor proteins such...
With the help of motor proteins such...
3.3K
 01:45
Tail-anchoring of Proteins in the ER Membrane
4.0K
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
4.0K
 01:28
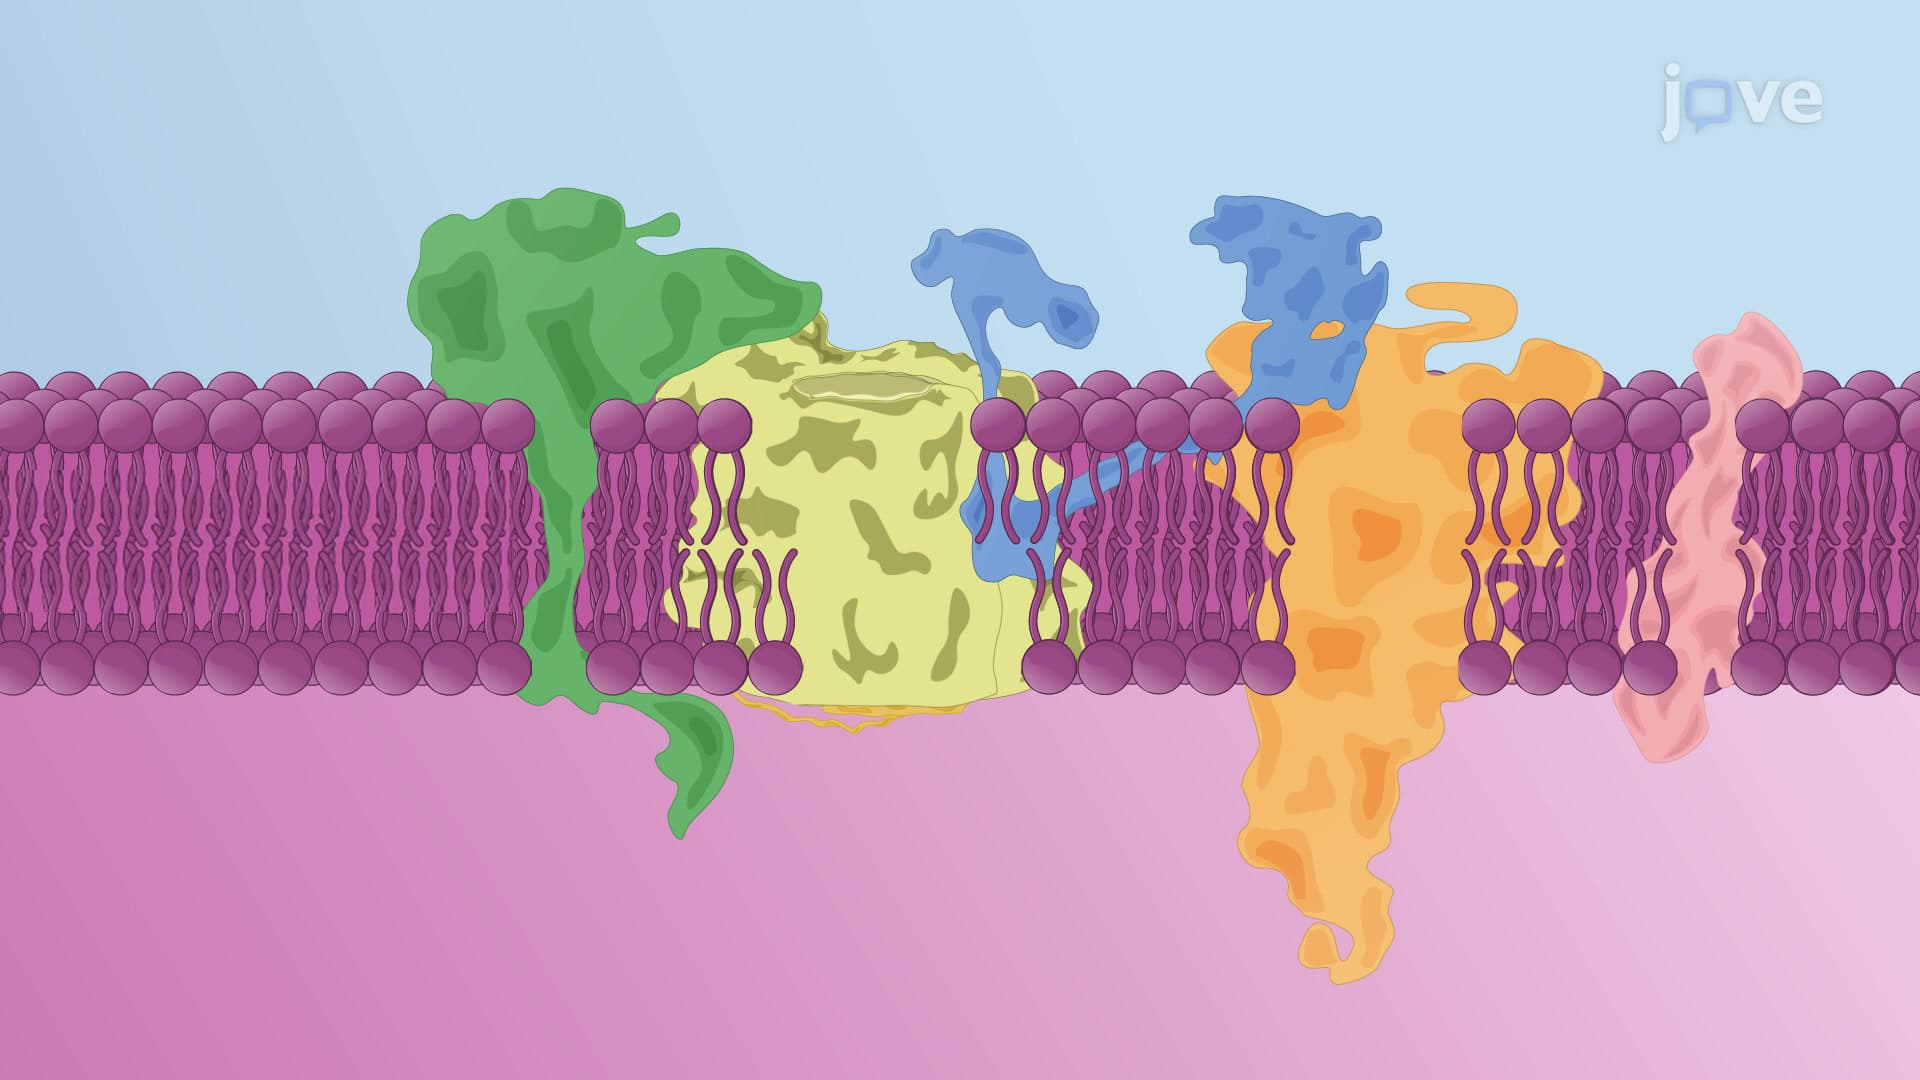
Protein Translocation Machinery on the ER Membrane
7.1K
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
7.1K