関連する実験動画
Updated: Feb 28, 2026
07:17

Purification of Hsp104, a Protein Disaggregase
Published on: September 30, 2011
17.8K
AAA+分解酵素Hsp104のラチェット型ポリペプチド転位機構
Stephanie N Gates1,2, Adam L Yokom1,2, JiaBei Lin3
1Department of Biological Chemistry, Life Sciences Institute, University of Michigan, Ann Arbor, MI 48109, USA.
Science (New York, N.Y.)
|June 17, 2017

まとめ
Hsp104タンパク質分解剤は,毒性タンパク質を展開する回転メカニズムを使用します. Cryo-EM構造は,毛穴に保存されたチロシンが基板と相互作用し,転位を促し,プロテオスタシスを維持することを明らかにします.
科学分野:
- 分子生物学
- 構造生物学
- 生物化学
背景:
- Saccharomyces cerevisiaeのHsp104を含むHsp100タンパク質は,プロテオスタシスの維持に不可欠なAAA+ ATPaseである.
- これらの分子機械は 異常なタンパク質を展開し 再折りや分解を ターゲットにします
- Hsp104は特にストレス誘発の無形積分とアミロイドを溶解させるが,基板相互作用と転位のメカニズムは不明である.
研究 の 目的:
- Hsp104による基質認識と転位の構造的基礎を解明する.
- 原子に近い解像度でHsp104媒介分解のメカニズムを理解する.
主な方法:
- Hsp104の構造を決定するために,冷凍電子顕微鏡 (cryo-EM) が使用されました.
- 近原子解像度構造はモデル基質であるカゼインを用いて得られた.
- 分析は,異なった転位状態のHsp104に焦点を当てた.
主要な成果:
- 構造は,80アングストロムの長さの展開されたポリペプチドと接触する保存された孔ループチロシンによって媒介された基板相互作用を明らかにした.
- 2つのプロトメアのラッチのような形状の変化は,2つのアミノ酸による毛穴ループ-基板の相互作用を進める.
- これらの形状の変化は,核酸水解と結合し,六合体周りに伝達され,プロセッシブな回転転移転機構を示します.
結論:
- Hsp104は,分断のためのプロセッシブローター転位メカニズムを使用しています.
- 基板に反応する柔軟性は,Hsp104の機能の重要な特徴です.
- この発見は,Hsp104が有毒なタンパク質の集積を分解することによって,タンパク質静止をどのように維持するかについての構造的な洞察を提供します.
さらに関連する動画
関連する概念動画
 01:37
Energy to Drive Translocation
2.9K
Mitochondrial protein import is powered by two distinct energy sources: ATP hydrolysis and electrochemical potential across the inner membrane. Newly synthesized precursors are bound by cytosolic chaperones of the Hsp70 family, which guide them to the import receptors on the mitochondrial surface. Utilizing the energy of ATP hydrolysis, Hsp70 chaperones transfer these precursors to the TOM receptors on the mitochondrial outer membrane.
Generally, polypeptides are unfolded by two distinct...
Generally, polypeptides are unfolded by two distinct...
2.9K
 01:19
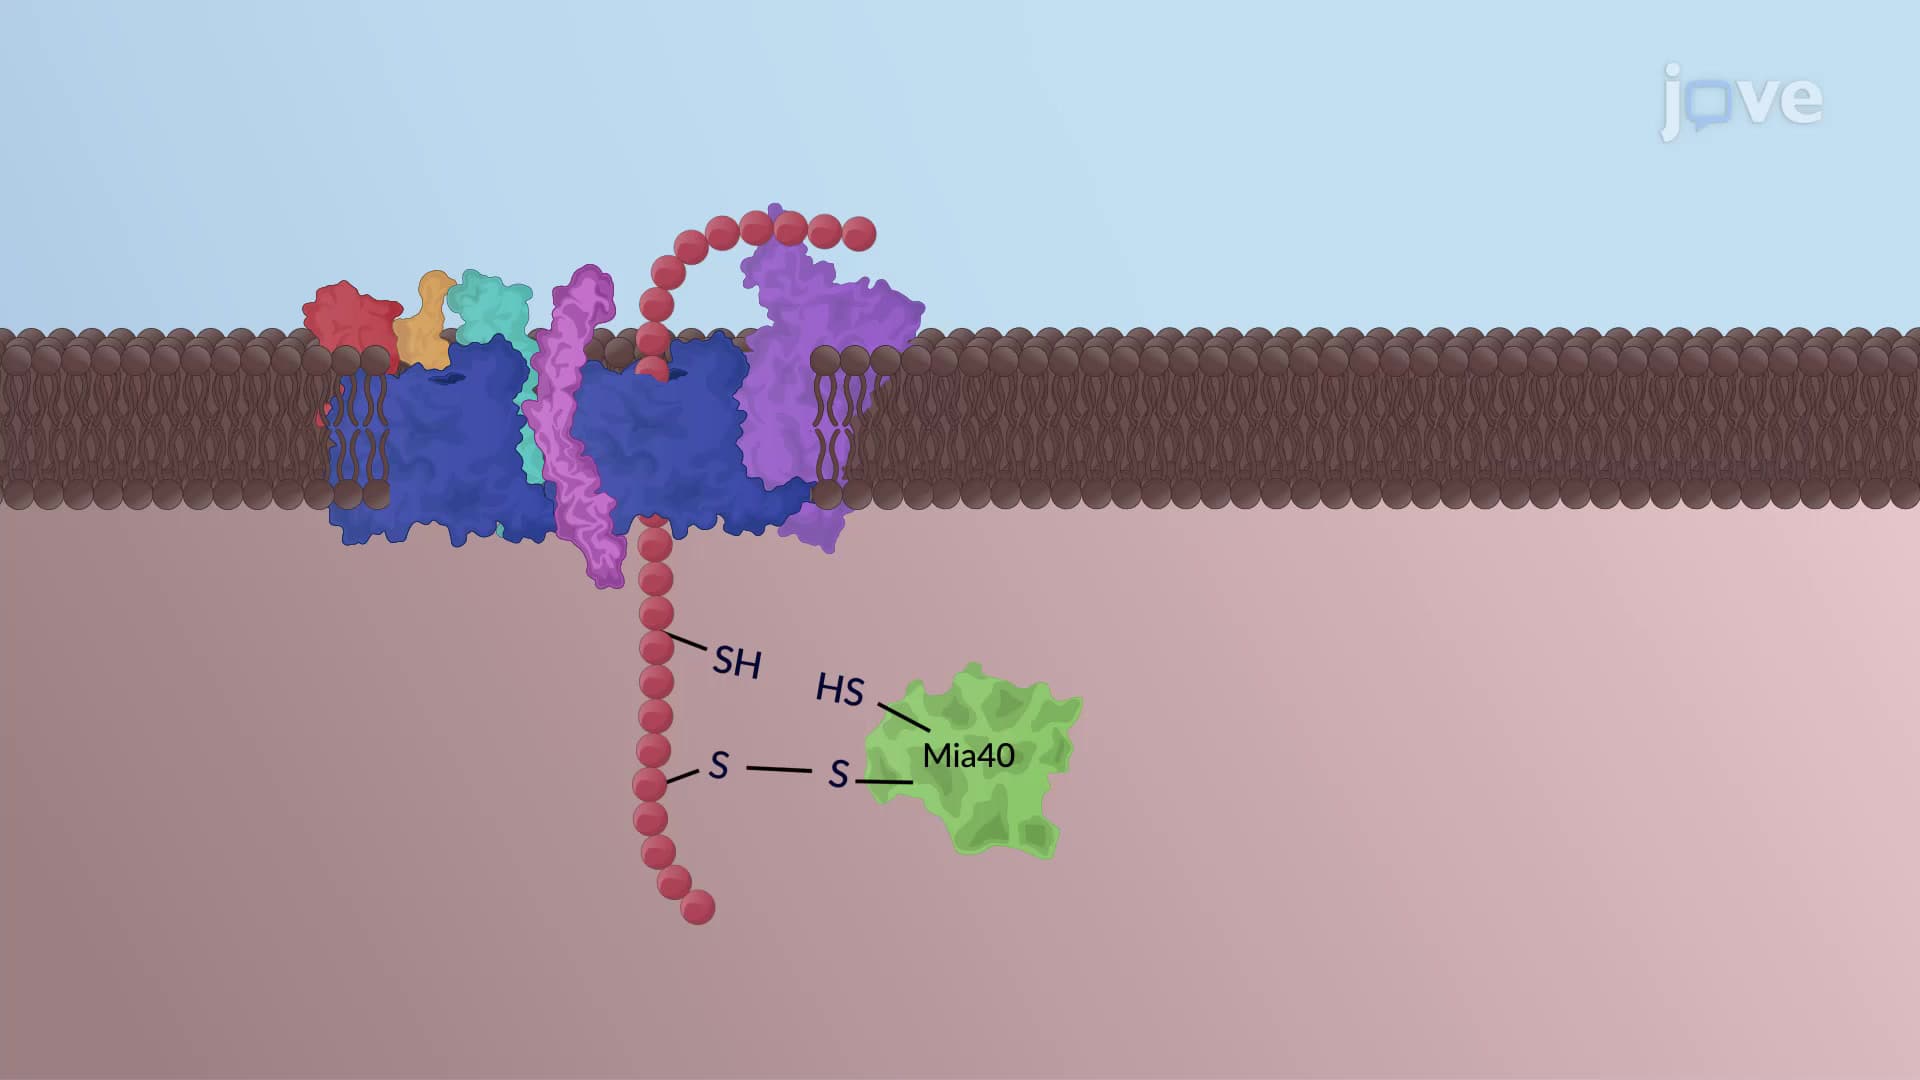
Translocation of Proteins into the Mitochondria
13.5K
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
13.5K
 01:27
Post-translational Translocation of Proteins to the RER
7.9K
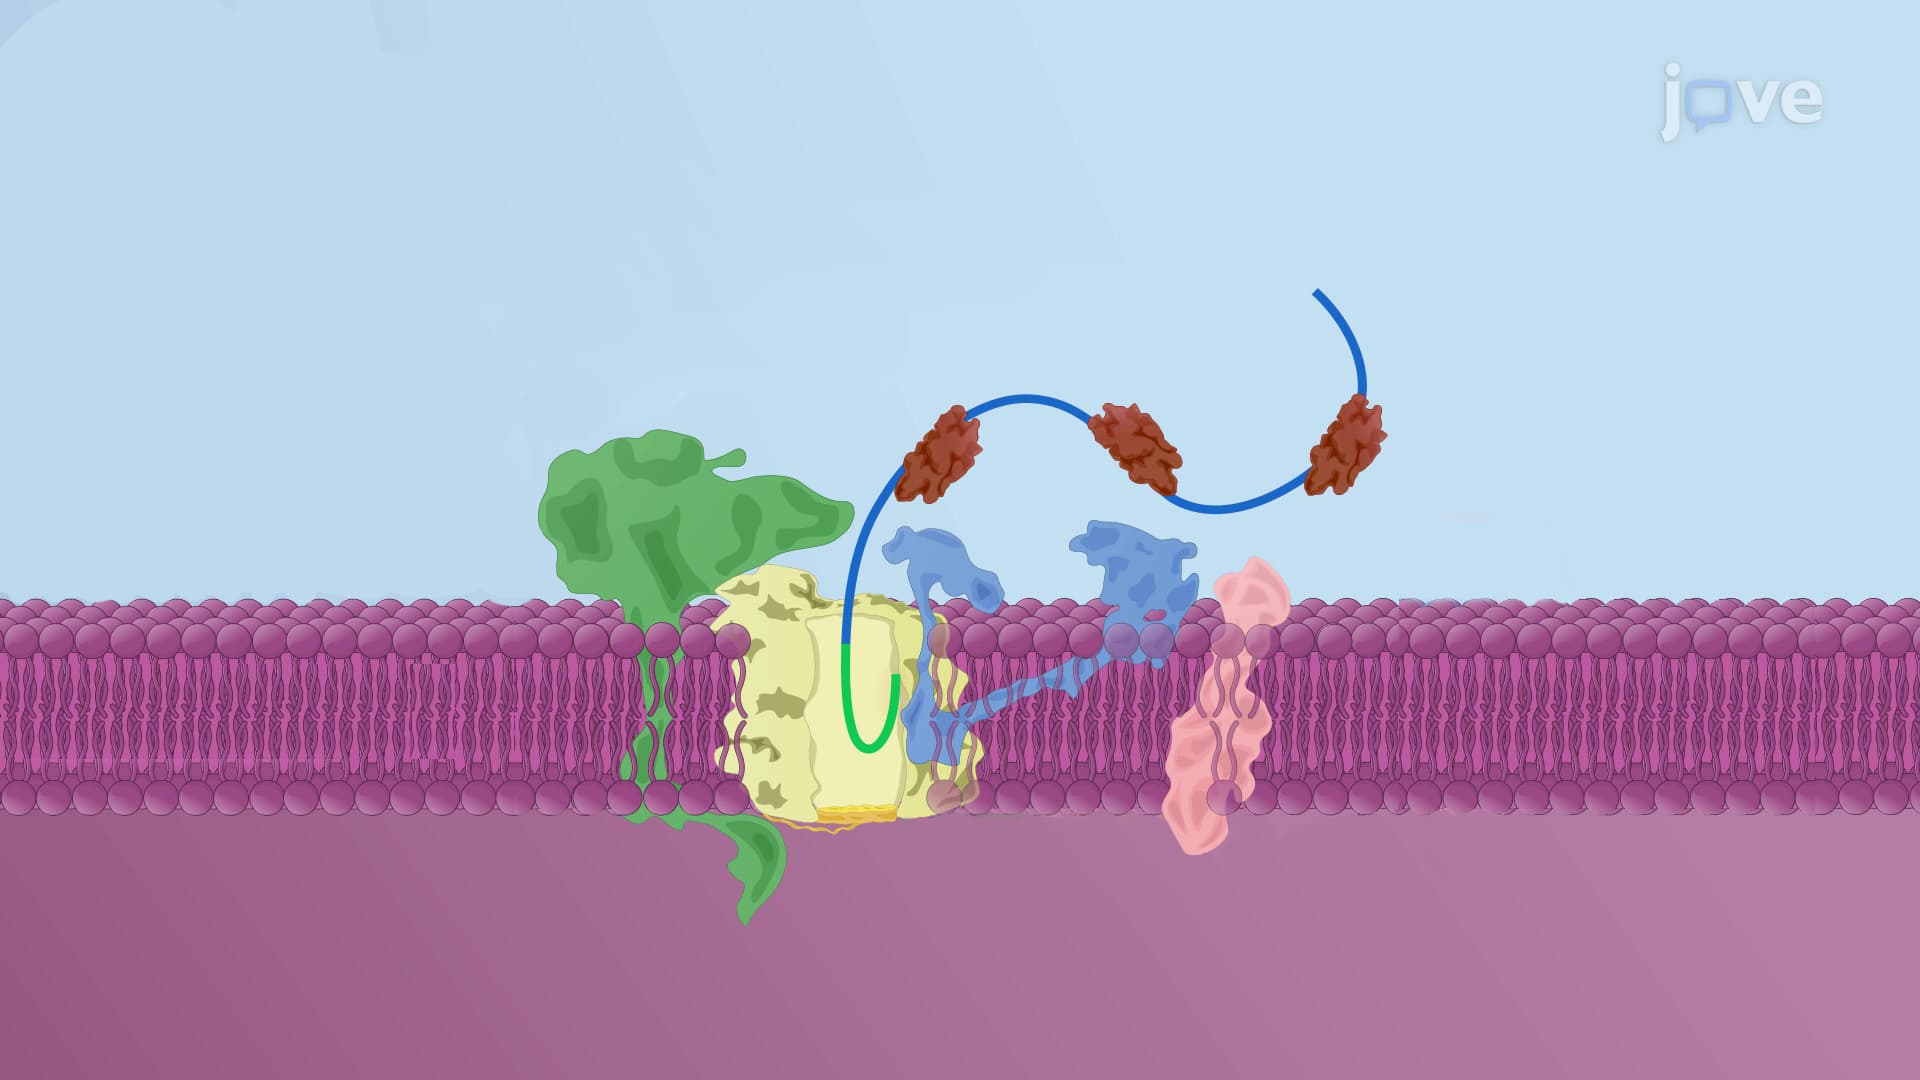
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
7.9K
 01:32
Export of Misfolded Proteins out of the ER
5.4K
After folding, the ER assesses the quality of secretory and membrane proteins. The correctly folded proteins are cleared by the calnexin cycle for transport to their final destination, while misfolded proteins are held back in the ER lumen. The ER chaperones attempt to unfold and refold the misfolded proteins but sometimes fail to achieve the correct native conformation. Such terminally misfolded proteins are then exported to the cytosol by ER-associated degradation or ERAD pathway for...
5.4K
 01:20
Cotranslational Protein Translocation
10.6K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
10.6K
 01:25
Rab Cascades
3.7K
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
3.7K