
RVFVのクラスII融合タンパク質のグリセロフォスホリピド特有のポケットは,標的膜の挿入を駆動する
P Guardado-Calvo1,2, K Atkovska3, S A Jeffers4,2
1Institut Pasteur, Département de Virologie, Unité de Virologie Structurale, 75724 Paris Cedex 15, France. pablo.guardado-calvo@pasteur.fr jhub@gwdg.de felix.rey@pasteur.fr.
Science (New York, N.Y.)
|November 4, 2017

まとめ
リフトバレー熱ウイルスの融合タンパク質 Gc は脂質に結合し,膜挿入メカニズムを明らかにします. この発見は 蚊媒介のウイルス病を理解し 対抗するために 極めて重要です
科学分野:
- ウイルス学
- 構造生物学
- 分子生物物理学
背景:
- リフトバレー熱ウイルス (RVFV) は,蚊によって感染し,アフリカにおける人間と家畜の健康に重大な脅威をもたらしています.
- ウイルスの侵入の分子メカニズムを理解することは,効果的な抗ウイルス戦略の開発に不可欠です.
研究 の 目的:
- 融合後の状態のRVFVクラスII融合タンパク質Gcの構造的基礎を解明する.
- ウイルス融合プロセスと膜相互作用におけるグリセロフォスホリピド (GPL) の役割を調査する.
主な方法:
- GPLと複合したRVFV Gcの構造を決定するために,X線結晶学を用いた.
- 結合機構と膜相互作用を分析するために,サイト指向型変異および分子動力学シミュレーションが使用されました.
主要な成果:
- RVFV Gcの融合後の構造は,融合ループの隣接するGPLを結合する保存された空洞を示した.
- 新しいモチーフは,核融合ループを標的膜にブロックで挿入することを容易にする.
- 特定の極性および非極性相互作用は,脂質ヘッド群とアリファティック部分の認識を統制する.
結論:
- 特定されたGPL結合部位と挿入モチーフは,RVFV膜融合に不可欠です.
- このメカニズムは,ジカウイルスやチクングンヤウイルスなどの他の重要なアーボウイルスの融合タンパク質に保存されています.
- RVFV Gcに関する構造的な洞察は,関連する新興ウイルスに対する広範囲の抗ウイルス薬の開発のための基盤を提供します.
関連する概念動画
 01:43
SNAREs and Membrane Fusion
13.0K
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
13.0K
 01:29
GPI Anchoring of Proteins in the ER Membrane
5.6K
GPI-anchoring is a post-translational, reversible protein modification that is ubiquitous in eukaryotes. Such proteins are primarily present on the exoplasmic leaflet of the plasma membrane.
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
5.6K
 01:12
Clathrin Coated Vesicles
9.6K
Clathrin-coated vesicles use endocytosis to transport receptors and lysosomal hydrolases from the Golgi to the lysosome in the late secretory pathway. Clathrin-mediated endocytosis was the first described endocytic process, and Clathrin-coated vesicles remain one of the most well-studied transport vesicles. The molecular machinery that generates clathrin-coated vesicles comprises over 50 proteins that precisely coordinate vesicle formation. Cell surface receptors concentrated in indented sites...
9.6K
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
18.3K
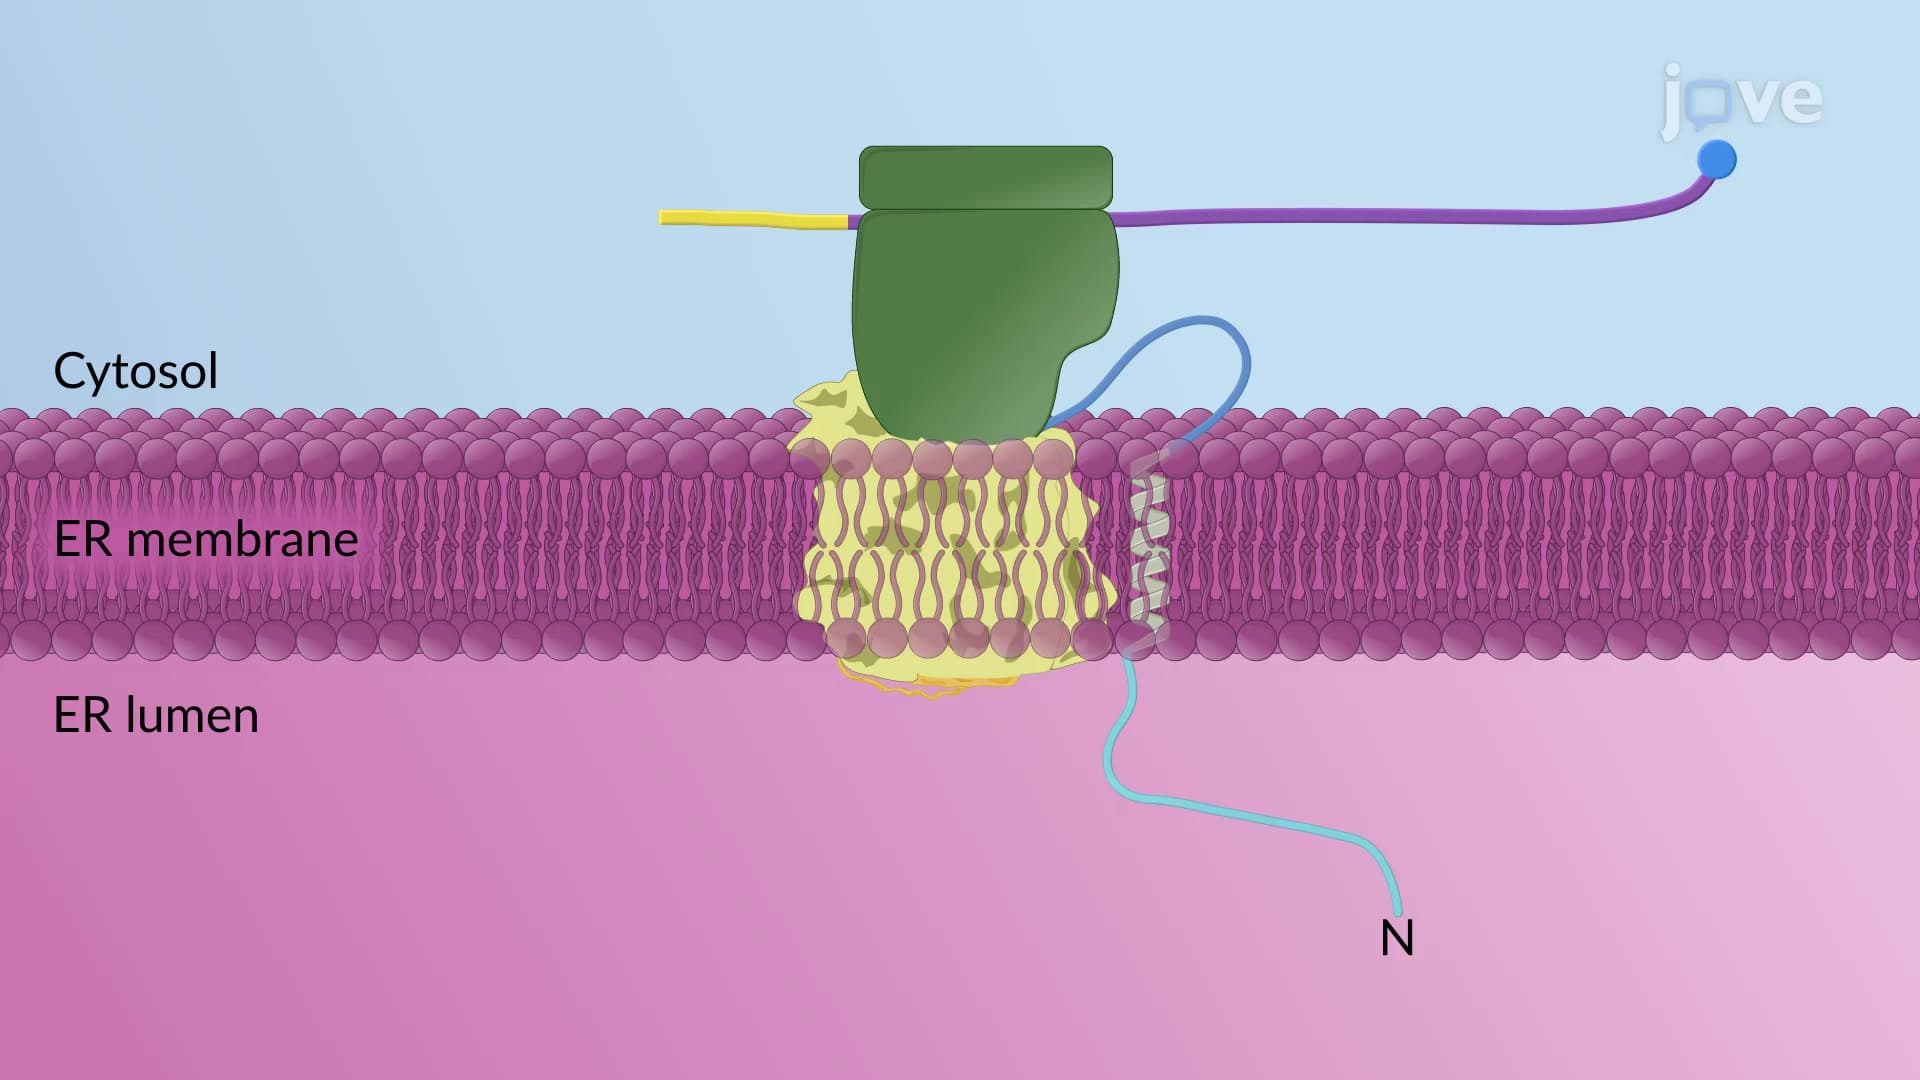
Integral membrane proteins are proteins adhered to the lipid bilayer of a cell organelle or membrane. They can be of two types: transmembrane integral proteins that span the lipid bilayer and monotopic proteins that are attached to either side of the membrane but do not pass through it.
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
18.3K
 01:14
Rab Proteins
5.2K
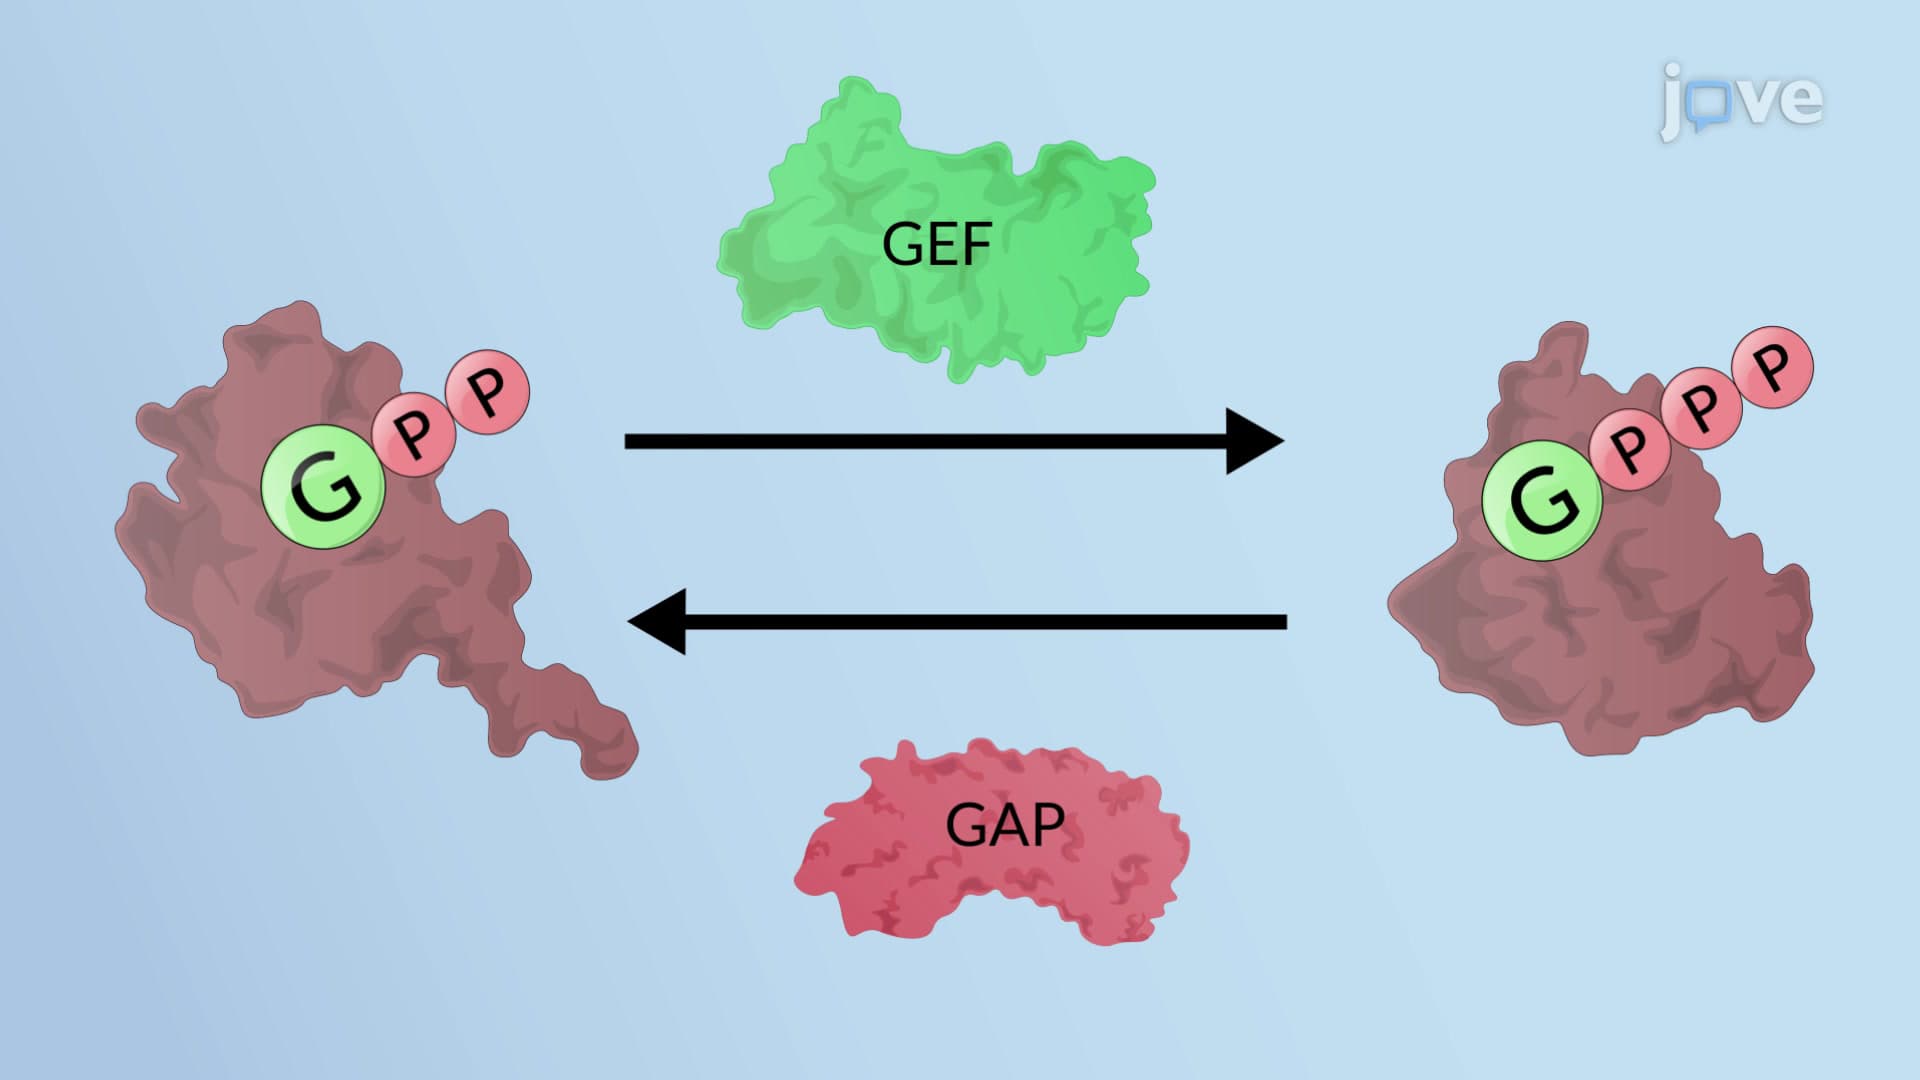
Rab proteins constitute the largest family of monomeric GTPases, of which 70 members are present in humans. Rab proteins and their effectors regulate consecutive stages of vesicle transport such as vesicle transport, docking, and fusion to the correct recipient membrane.
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
5.2K
 01:25
Rab Cascades
3.6K
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
3.6K