関連する実験動画
Updated: May 5, 2026
06:45

Transmembrane Domain Oligomerization Propensity determined by ToxR Assay
Published on: May 26, 2011
14.6K
外来型トランスメブランペプチドは,トランスフェリン受容体の内部信号配列を代替し,その転位と膜結合を可能にします
Cell
|January 16, 1987

まとめ
トランスファーリン受容体 (TR) のトランスメブランセグメントは,その機能にとって極めて重要です. 特定のアミノ酸ではなく,水嫌性の性質が,鎖の転位と,TRがER膜に挿入されるための膜の固定を促します.
科学分野:
- 細胞生物学 細胞生物学
- 分子生物学は分子生物学である.
- 膜タンパク質生物学 膜タンパク質生物学
背景:
- 人間のトランスファーリン受容体 (TR) は,鉄の吸収に不可欠なトランスメブランタンパク質です.
- 各TRサブユニットは,細胞質のN端でエンドプラズマ網膜 (ER) 膜に挿入されます.
- TRのトランスメブランセグメントは,タンパク質転位のためのシグナル伝達と,タンパク質を膜内に固定するという二重な役割を果たします.
研究 の 目的:
- タンパク質転位と膜固定における二重機能のためのTRトランスメブランセグメントの特殊な構造的要件を調査する.
- 超膜セグメントのアミノ酸配列か,あるいは,その水害性の性質が,その活性にとって重要かどうかを判断する.
主な方法:
- TRトランスメブランセグメントの突然変異.
- 本来のTRトランスメブランペプチドを,他のタンパク質または人工ペプチドのセグメントに置き換える.
- 変異したTR分子の機能を評価するためのインビトロ転位アッセイ.
主要な成果:
- 変異したトランスメブランセグメント (人工の未充電ペプチドを含む) を含む変異TR分子は,in vitroで効率的に転位されました.
- TRトランスメブランペプチドを水性ペプチドに置き換えることで,検出可能な転位活動が廃止されました.
- これらの発見は,水害性の性質がトランスメブランセグメントの機能に不可欠であることを示しています.
結論:
- トランスフェリン受容体のトランスメブランセグメントの水性性は,鎖転位と膜結合におけるその役割に極めて重要です.
- このセグメントの特定のアミノ酸配列は,これらの機能のためにその全体的な水性よりも重要ではありません.
- この研究では,トランスメブランタンパク質の挿入と機能を制御する重要な特徴を明らかにしています.
関連する概念動画
 01:28
The Early Endosome: Endocytosis of Transferrin
4.1K
Essential proteins such as insulin or low-density lipoprotein (LDL) and micronutrients such as iron enter a eukaryotic cell through receptor-mediated endocytosis. Subsequently, the early endosomes fuse with the vesicles containing such receptor-ligand complexes and play a vital role in sorting the incoming ligands and receptors. While the ligands are either degraded inside the vesicle or released into the cytosol, their receptors are returned to the plasma membrane for further rounds of...
4.1K
 01:19
Translocation of Proteins into the Mitochondria
8.8K
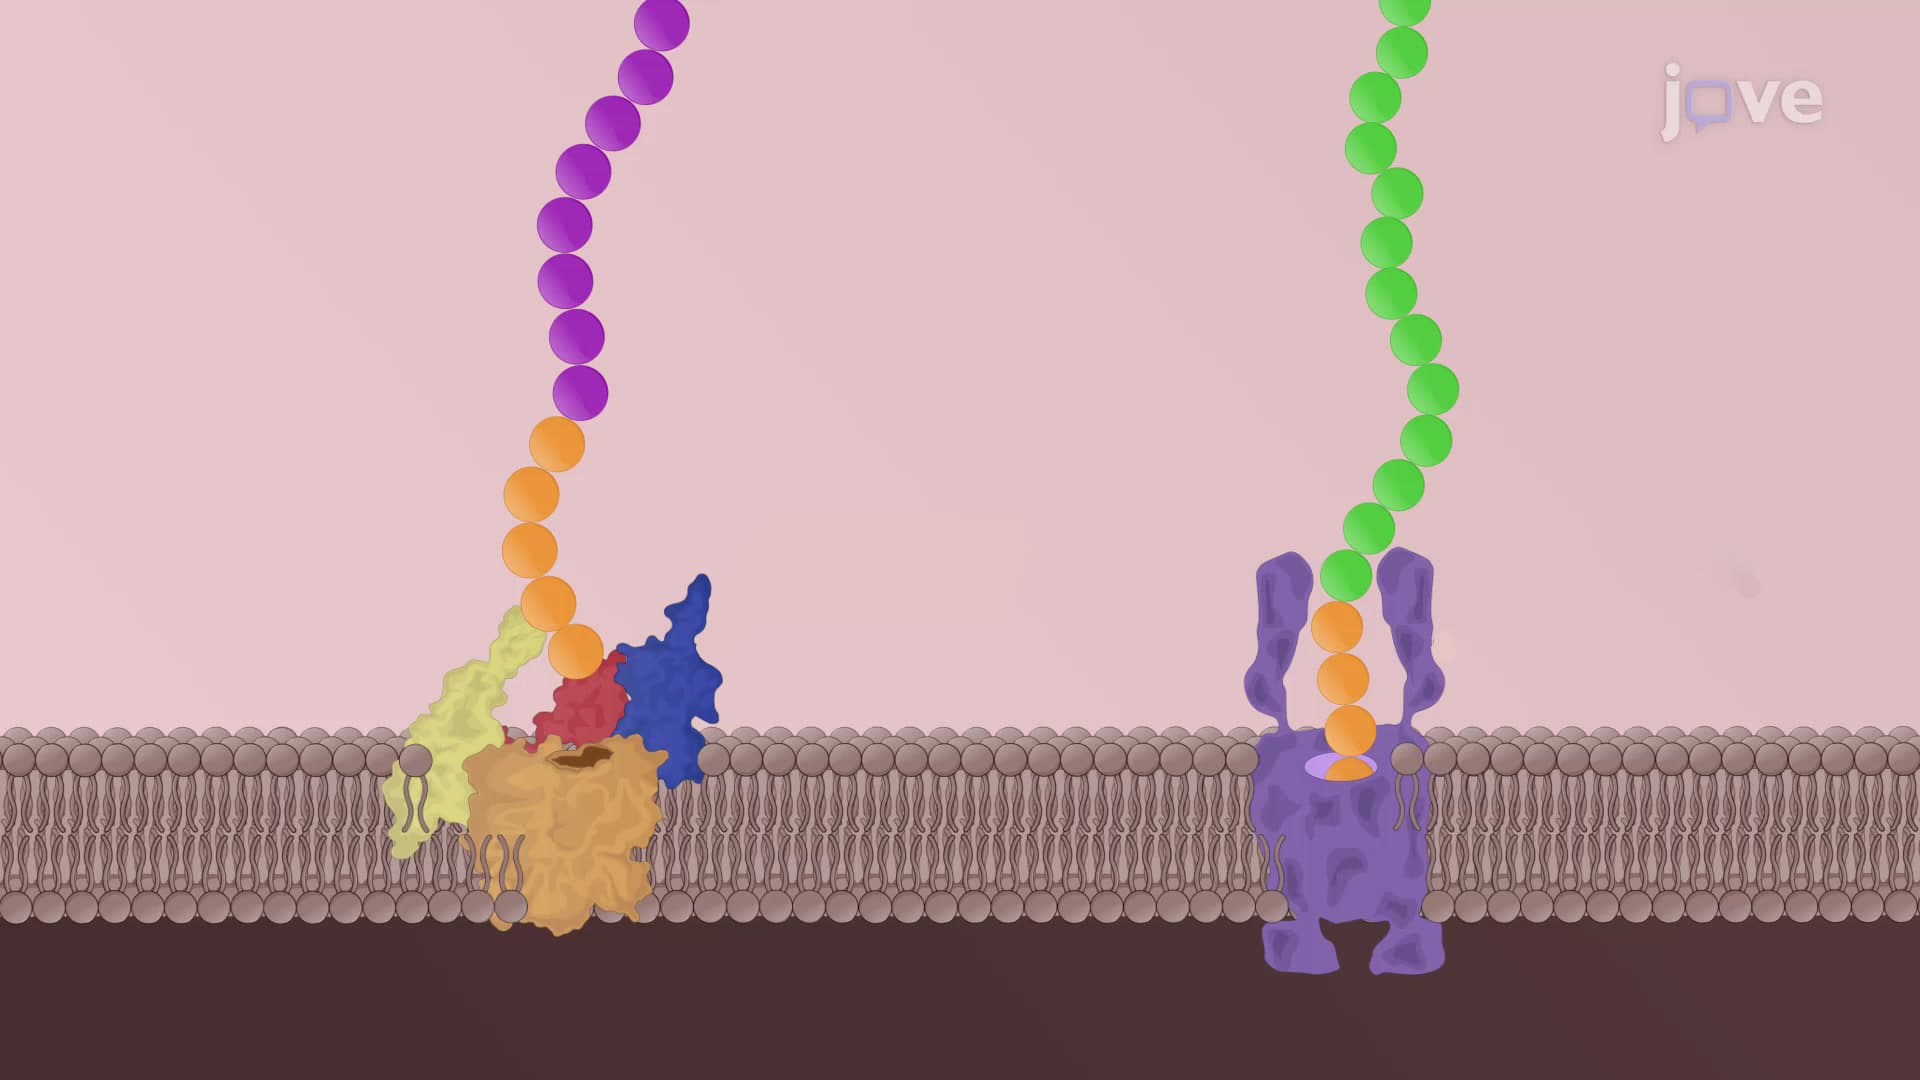
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
8.8K
 01:34
Protein Transport into the Inner Mitochondrial Membrane
3.5K
Nuclear encoded mitochondrial precursors are imported to the inner membrane in a multistep process involving two separate translocons, TIM22 and TIM23. TIM23 is a cation-selective pore that remains closed by the N terminal segment of the protein. Negative charges on the TIM23 act as a receptor for the incoming precursor, pulling the positively charged matrix-targeting sequence for peptide insertion and translocation.
Transport of mitochondrial precursors across the TIM23 channel is driven by...
Transport of mitochondrial precursors across the TIM23 channel is driven by...
3.5K
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
13.0K
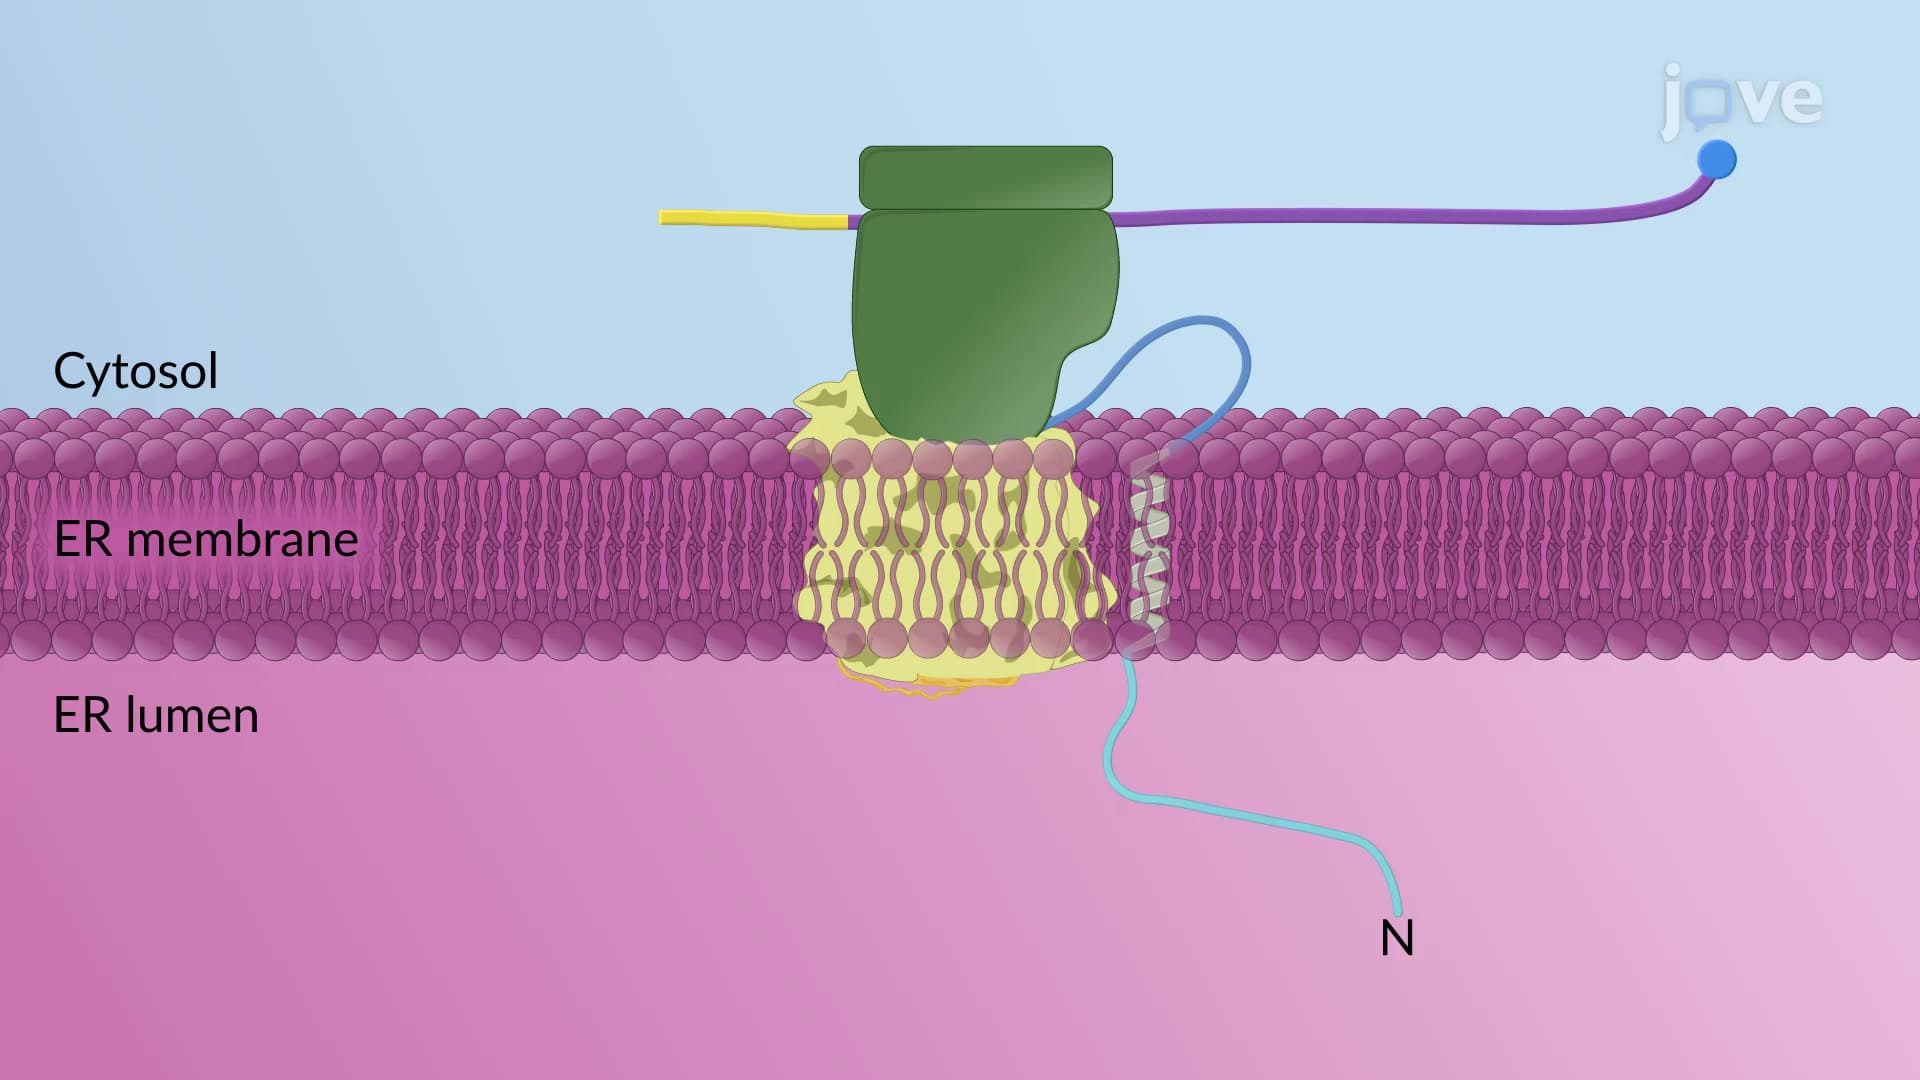
Integral membrane proteins are proteins adhered to the lipid bilayer of a cell organelle or membrane. They can be of two types: transmembrane integral proteins that span the lipid bilayer and monotopic proteins that are attached to either side of the membrane but do not pass through it.
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
13.0K
 01:29
Insertion of Multi-pass Transmembrane Proteins in the RER
13.5K
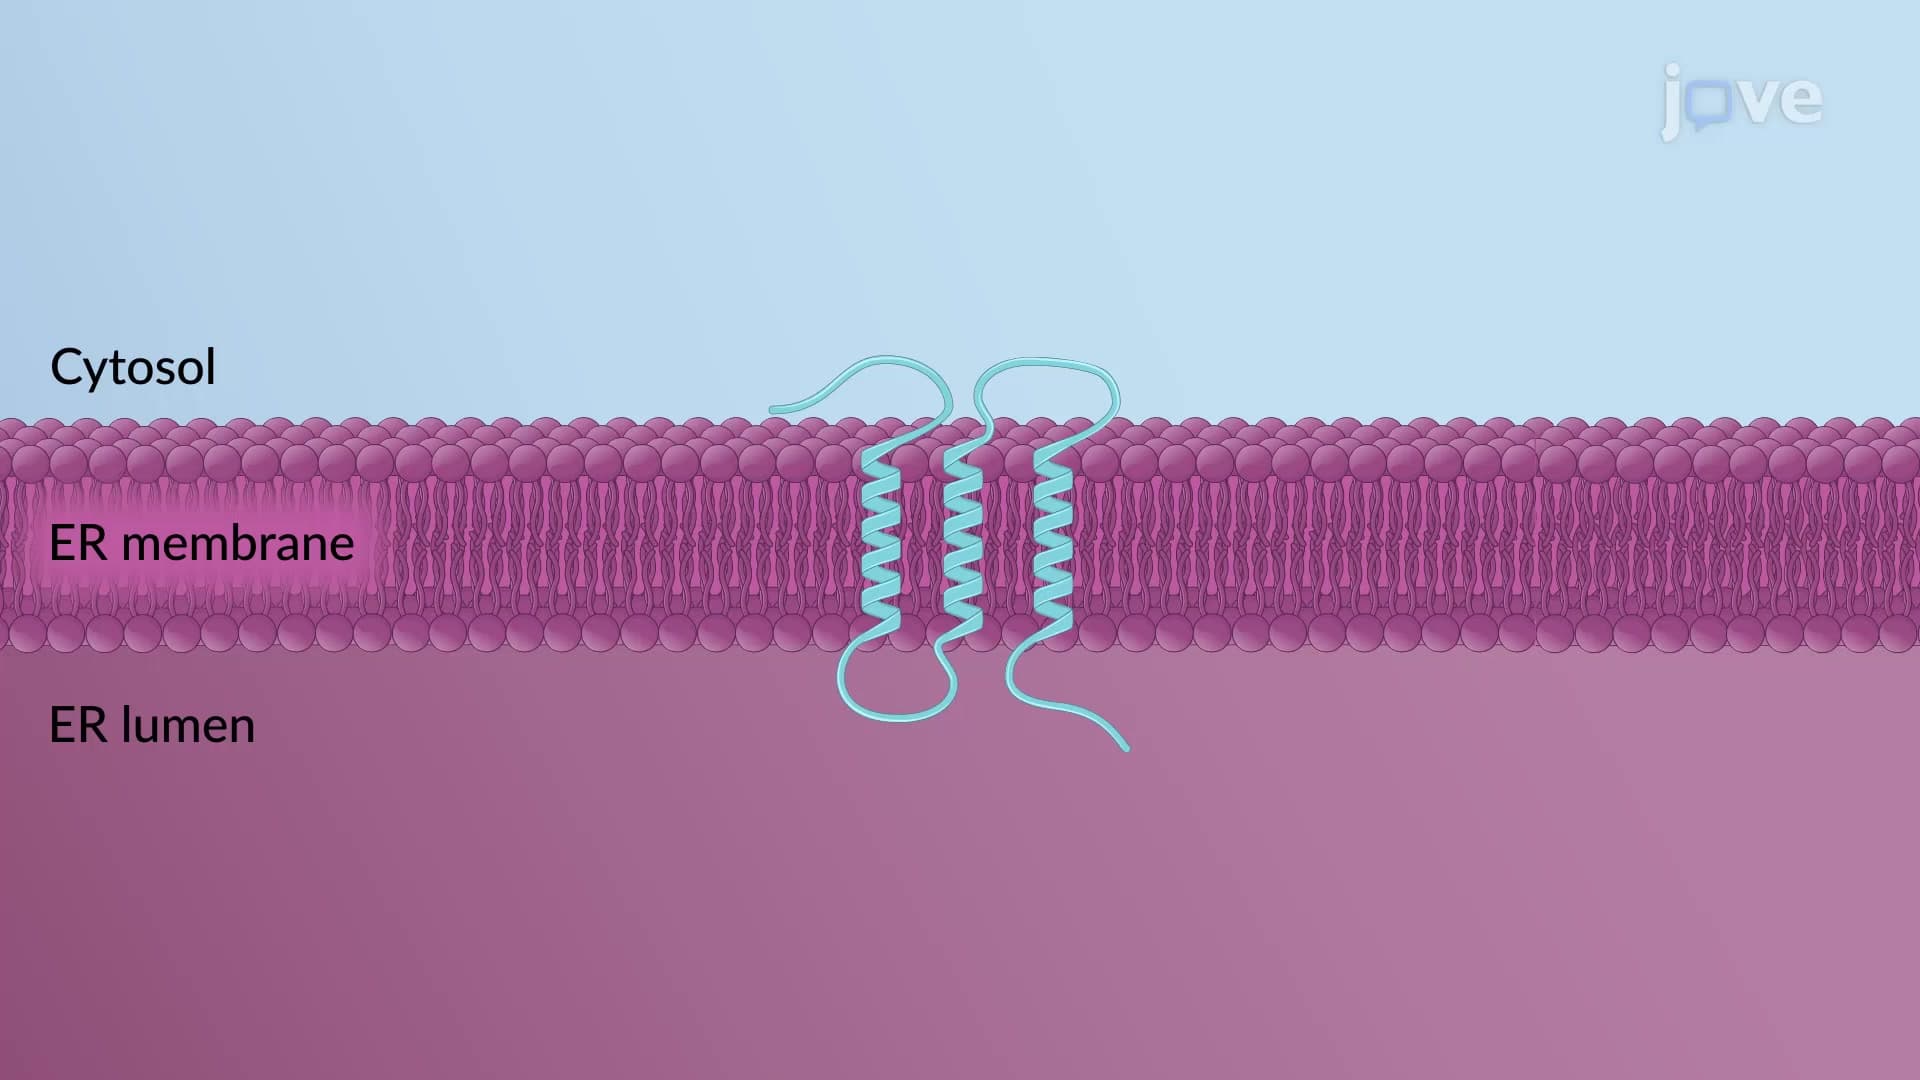
The rough ER membrane synthesizes, assembles, and embeds transmembrane proteins in diverse topologies. These proteins function as transporters or channels and can remain in the ER membrane or are sent to the Golgi complex, lysosome, and cell membrane.
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
13.5K
 01:27
Post-translational Translocation of Proteins to the RER
5.6K
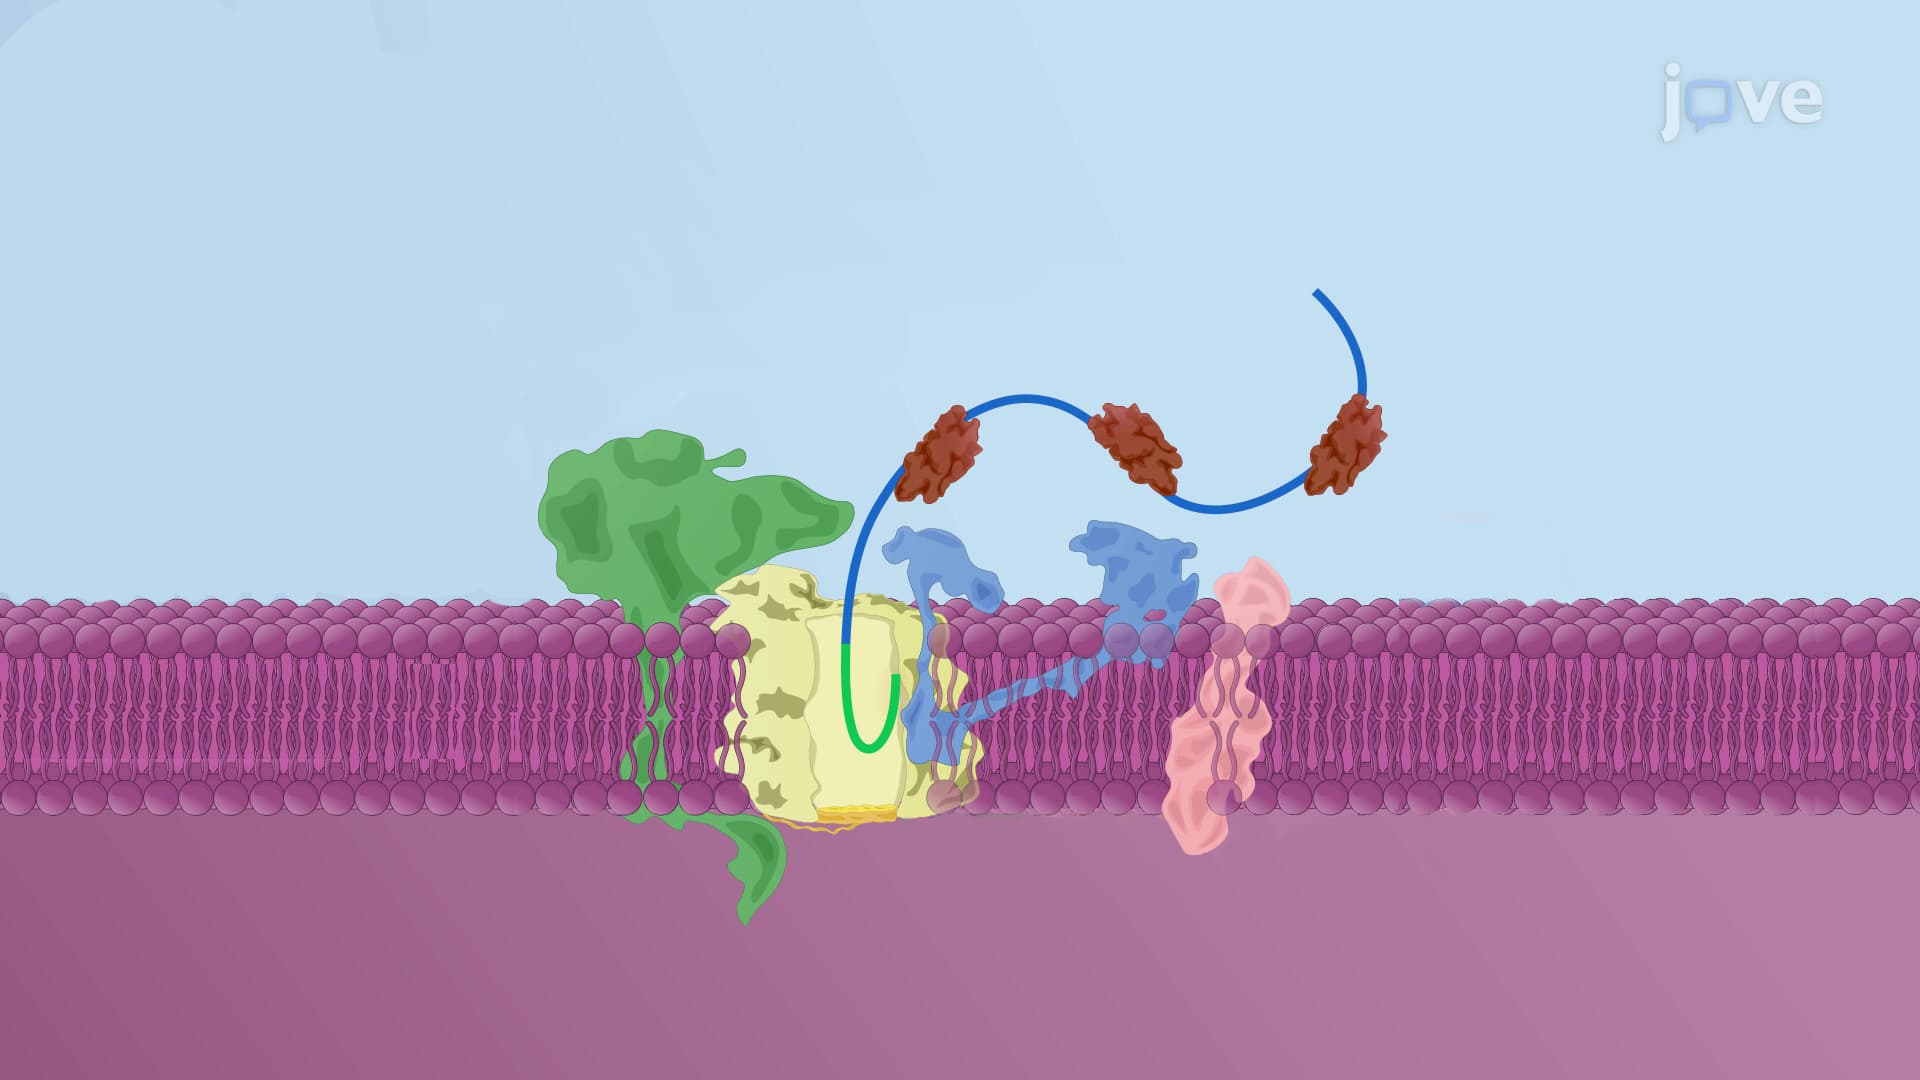
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
5.6K