
UFM1 E3リガゼは,ERトランスロコンから60Sリボソームを認識して放出する
Linda Makhlouf1, Joshua J Peter2, Helge M Magnussen2
1Astbury Centre for Structural Molecular Biology, School of Molecular and Cellular Biology, Faculty of Biological Sciences, University of Leeds, Leeds, UK.
Nature
|February 21, 2024

まとめ
UFM1リボソームE3リガゼ (UREL) 複合体は,停止したリボソームを修正し,ER膜から放出を促進します. このUFMylationプロセスは,タンパク質ホメオスタシスに不可欠であり,リボソームをSEC61トランスロコンから分離することによってリサイクルします.
科学分野:
- 分子生物学
- 細胞生物学
- 構造生物学
背景:
- エンドプラズマ網膜 (ER) での停止したリボソームは,60Sリボソームサブユニット (RPL26) のユビキチンのようなタンパク質UFM1によって改変される.
- このUFMylationと呼ばれるプロセスは,UFL1,UFBP1,CDK5RAP3で構成されるUFM1リボソームE3リガゼ (UREL) 複合体によって媒介されます.
- URELの正確な触媒メカニズムとUFMylationの機能的結果は,大部分が未決定のままである.
研究 の 目的:
- URELの基板特異性の構造的基礎を明らかにする.
- ERにおけるリボソームリサイクルとタンパク質ホメオスタシスにおけるUFMylationの機能的影響を理解する.
- SEC61トランスロコンからのリボソームの解離におけるUFMylationの役割を調査する.
主な方法:
- 60Sリボソームに結合したUREL複合体の構造を決定するために,冷凍電子顕微鏡 (cryo-EM) が使用された.
- 60SサブユニットからSEC61を放出するためにUFMylationの必要性を評価するために生化学的測定法を使用した.
- URELの構造的特徴と機能的状態 ("ライター"と"リーダー"モジュール) の分析が行われました.
主要な成果:
- クリオ-EM構造は,URELが60Sサブユニット周りにC形のクランプを形成し,tRNA結合部位とペプチド出口トンネルを阻害することを明らかにします.
- UREL内のUFL1ループはペプチジルトランスファーゼセンターを再構成し,リボソームの放出とリサイクルにおける役割を示唆しています.
- 機能的研究では,UFMylationは,SEC61トランスロコンから60Sサブユニットを分離するために不可欠であり,ER膜での蓄積を防止します.
結論:
- URELのクランプのような構造とペプチジルトランスファーゼセンターとの相互作用は,リボソーム放出におけるその機能の鍵です.
- UFMylationは,ER膜から停滞したリボソームを解放し,効率的なタンパク質ホメオスタシスを確保する重要なステップです.
- URELは,UFMylationの"ライター"と"リーダー"の両方として機能し,リボソームリサイクルのためのユニークな規制メカニズムを強調します.
関連する概念動画
 01:28
Protein Translocation Machinery on the ER Membrane
4.6K
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
4.6K
 01:20
Cotranslational Protein Translocation
7.4K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
7.4K
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.3K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.3K
 01:27
Post-translational Translocation of Proteins to the RER
5.7K
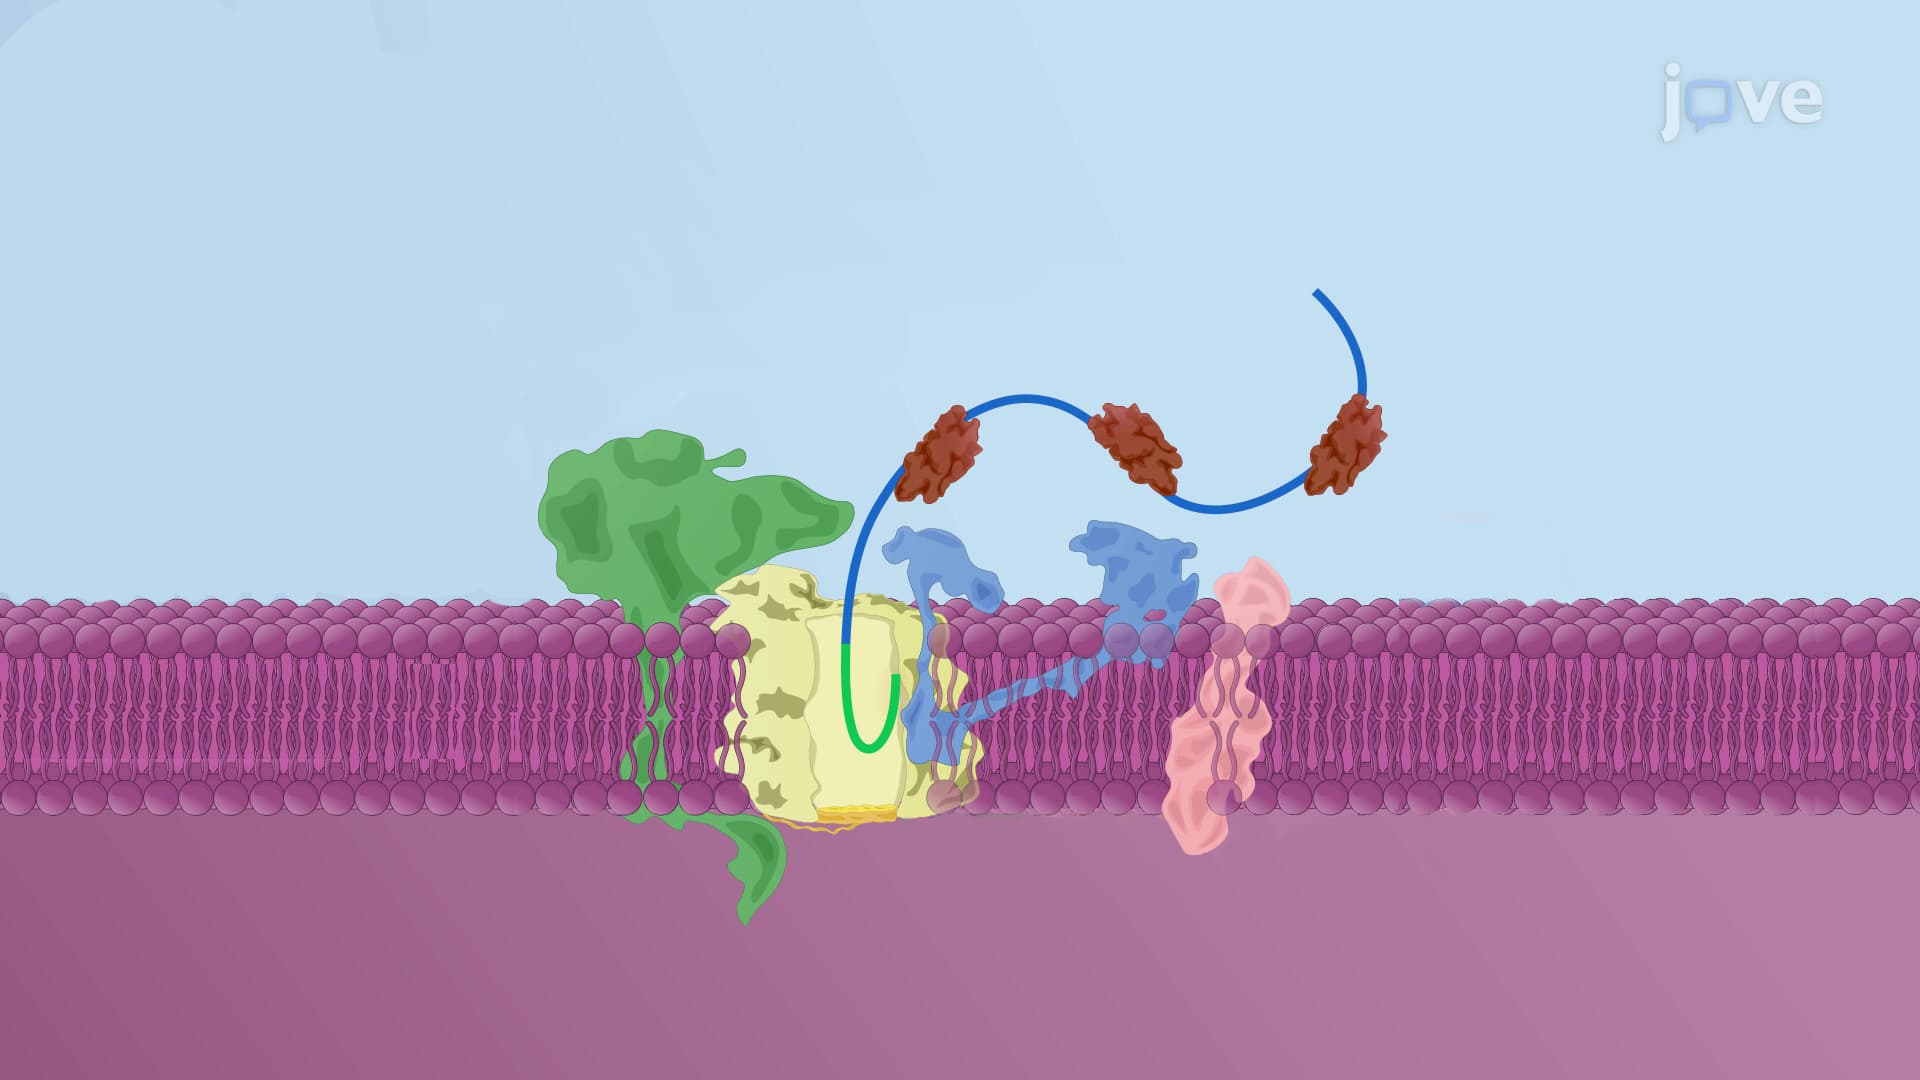
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
5.7K
 02:07
Improving Translational Accuracy
10.4K
Base complementarity between the three base pairs of mRNA codon and the tRNA anticodon is not a failsafe mechanism. Inaccuracies can range from a single mismatch to no correct base pairing at all. The free energy difference between the correct and nearly correct base pairs can be as small as 3 kcal/ mol. With complementarity being the only proofreading step, the estimated error frequency would be one wrong amino acid in every 100 amino acids incorporated. However, error frequencies observed in...
10.4K
 01:27
Ribosomes
7.6K
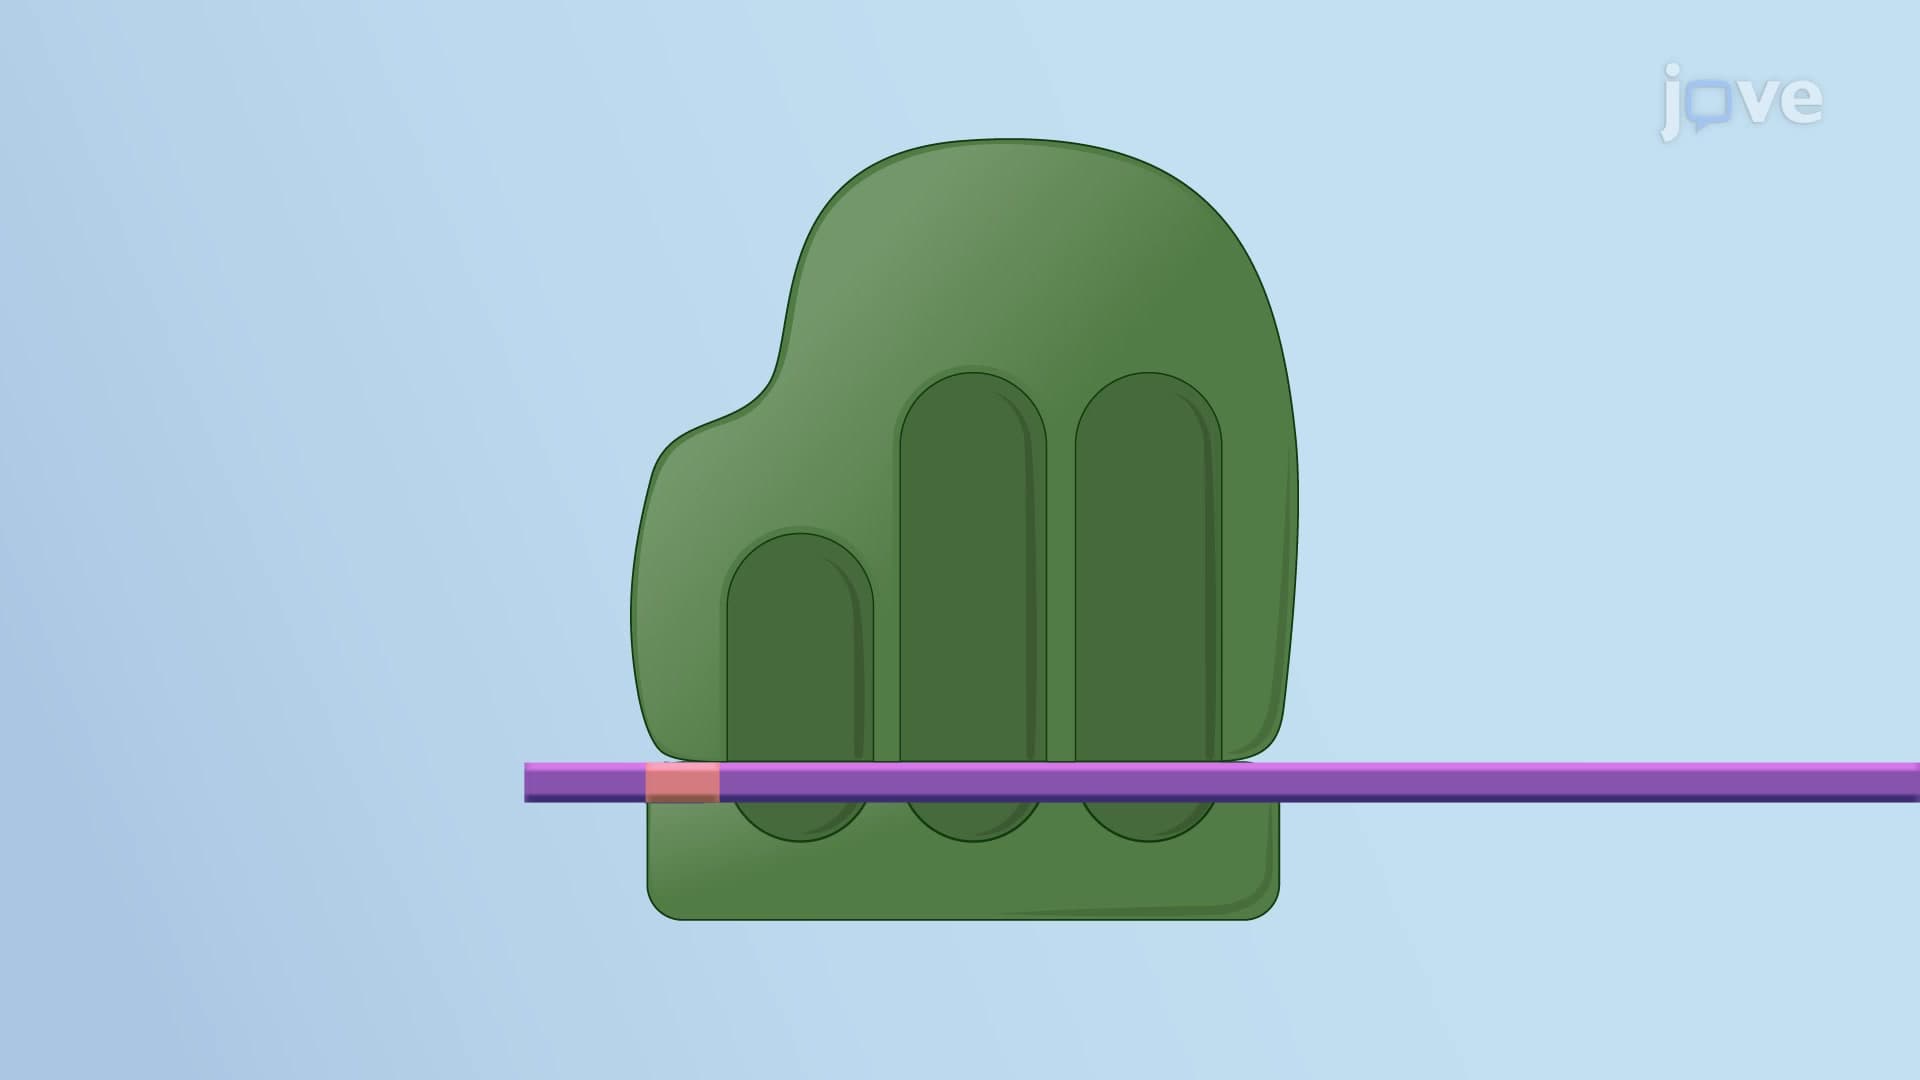
Ribosomes translate genetic information encoded by messenger RNA (mRNA) into proteins. Both prokaryotic and eukaryotic cells have ribosomes. Cells that synthesize large quantities of protein—such as secretory cells in the human pancreas—can contain millions of ribosomes.
Ribosome Structure and Assembly
Ribosomes are composed of ribosomal RNA (rRNA) and proteins. In eukaryotes, rRNA is transcribed from genes in the nucleolus—a part of the nucleus that specializes in ribosome...
Ribosome Structure and Assembly
Ribosomes are composed of ribosomal RNA (rRNA) and proteins. In eukaryotes, rRNA is transcribed from genes in the nucleolus—a part of the nucleus that specializes in ribosome...
7.6K