関連する実験動画
Updated: Jun 11, 2025
06:26

Pulling Membrane Nanotubes from Giant Unilamellar Vesicles
Published on: December 7, 2017
10.9K
生物分子の凝縮物は,エンドソーム膜の折り畳みと分裂を媒介する
Yanning Wang1, Shulin Li1, Marcel Mokbel2
1School of Life Sciences, Tsinghua University, Beijing, China.
Nature
|October 9, 2024

まとめ
植物タンパク質のFREE1は,多胞体における膜分裂を誘発する液体状の凝縮物を形成する. このコンデンサ媒介メカニズムは,ESCRT機械とは独立しており,植物のオスモティックストレス耐性にとって不可欠です.
科学分野:
- 細胞生物学
- バイオ物理学
- 分子植物学
背景:
- 多細胞体 (MVB) は,細胞の品質管理に不可欠な内分体である.
- ESCRT (輸送に必要な内分体分類複合体) 機械は,通常,MVB内の貨物の飲み込みと内分体胞 (ILV) の形成を媒介する.
- ESCRTに依存するILV形成はATPを必要とし,膜の侵入と分裂を伴う.
研究 の 目的:
- 植物のESCRT成分FREE1が内小胞の形成に果たす役割を調査する.
- MVBの生殖過程における膜分裂の基礎となる生理学的メカニズムを解明する.
- 凝縮物媒介と機械媒介による分裂の相互作用を in vivo で探求する.
主な方法:
- 最小限の物理モデリング
- インビトロ溶解実験
- シリコンシミュレーションで
- ユカリオットのESCRT経路の遺伝子操作
主要な成果:
- 植物のESCRTコンポーネントFREE1は,膜と結合する液体状の凝縮物を形成する.
- FREE1コンデンサは,コンデンサを濡らすことによる力によって,内小胞の形成を促します.
- 膜分裂は,ESCRT機械とATP消費から独立して,コンデンサート媒介メカニズムによって起こる.
- コンデンサ媒介による分裂は,植物におけるオスモティックストレス耐性にとって不可欠である.
結論:
- 凝縮物媒介による分裂は,MVBの生体形成における膜ダイナミクスの新しいメカニズムである.
- このプロセスは,凝縮物と膜の湿潤現象の物理化学的性質に依存しています.
- コンデンサとESCRT媒介による分裂の相互作用は,プラントのストレス適応に極めて重要です.
- 湿った現象は細胞内組織と 流通プロセスにおいて根本的な役割を果たします
関連する概念動画
 01:15
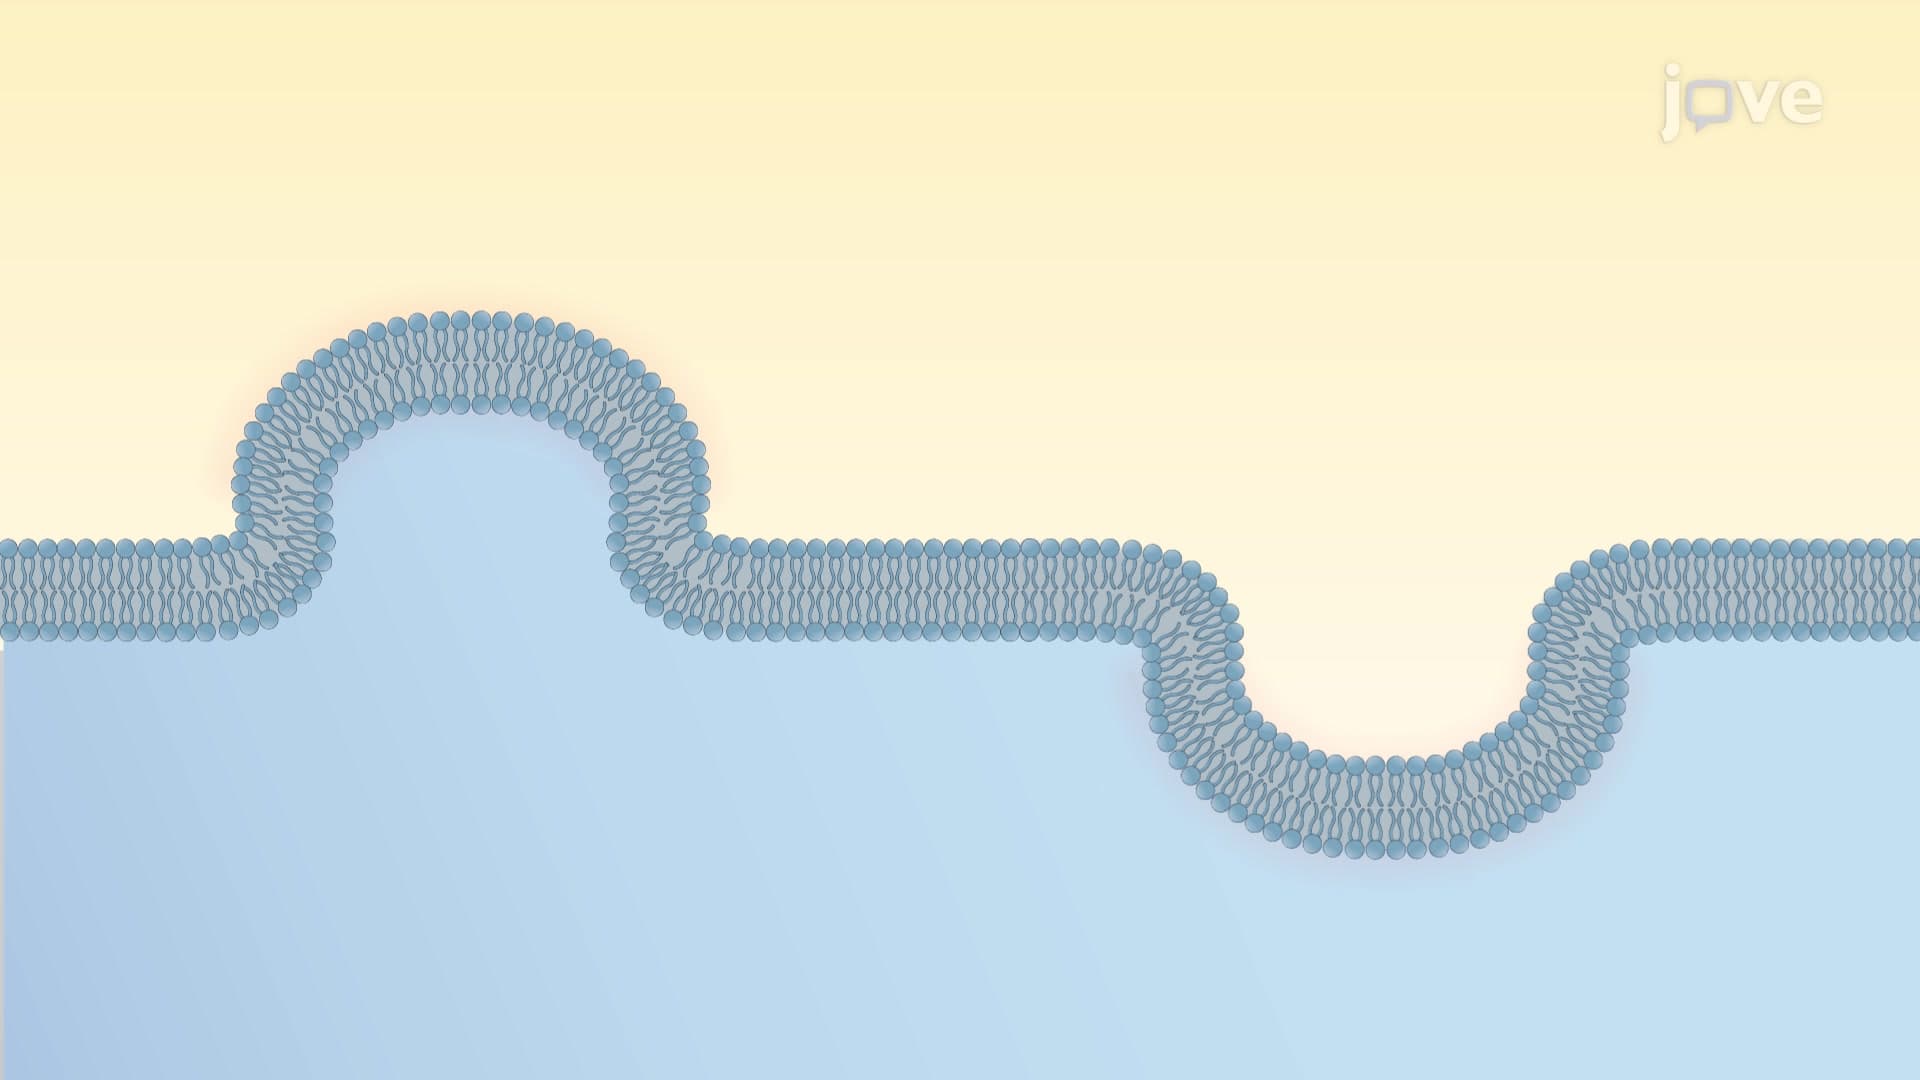
Mechanisms of Membrane-bending
2.6K
The living membranes are flexible due to their fluid mosaic nature; however, their bending into different shapes is an active process regulated by specific lipids and proteins. The membrane bending can be transient as seen in vesicles or stable for a long time as in microvilli. Cells regulate the size, location, and duration of the membrane curvature.
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
2.6K
 01:43
SNAREs and Membrane Fusion
10.8K
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
10.8K
 01:32
Pinching-off of Coated Vesicles
3.1K
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
3.1K
 01:38
Intralumenal Vesicles and Multivesicular Bodies
3.4K
Intraluminal vesicles (ILVs) are small vesicles 50-80 nm in diameter formed during the maturation of early endosomes. A specialized endosome containing numerous ILVs is called a multivesicular body (MVB). ILVs contain internalized molecules such as antigens, nucleic acids, proteins, and metabolites. Some of these molecules are released from the MVBs inside exosomes and are transported to other cells. Other MVBs contain molecules that are retained in the ILVs and are later degraded within the...
3.4K
 00:59
Mechanisms of Membrane Domain Formation
3.0K
Different physical properties of lipids and proteins allow them to localize and form distinct islands or domains in the membrane. Some membrane domains are formed due to protein-protein interactions, whereas others are formed due to the presence of specific lipids such as sphingolipids and sterols—for example, large proteins, such as bacteriorhodopsin, aggregate and create distinct domains.
Another mechanism for membrane domain formation involves membrane proteins interacting with...
Another mechanism for membrane domain formation involves membrane proteins interacting with...
3.0K
 02:15
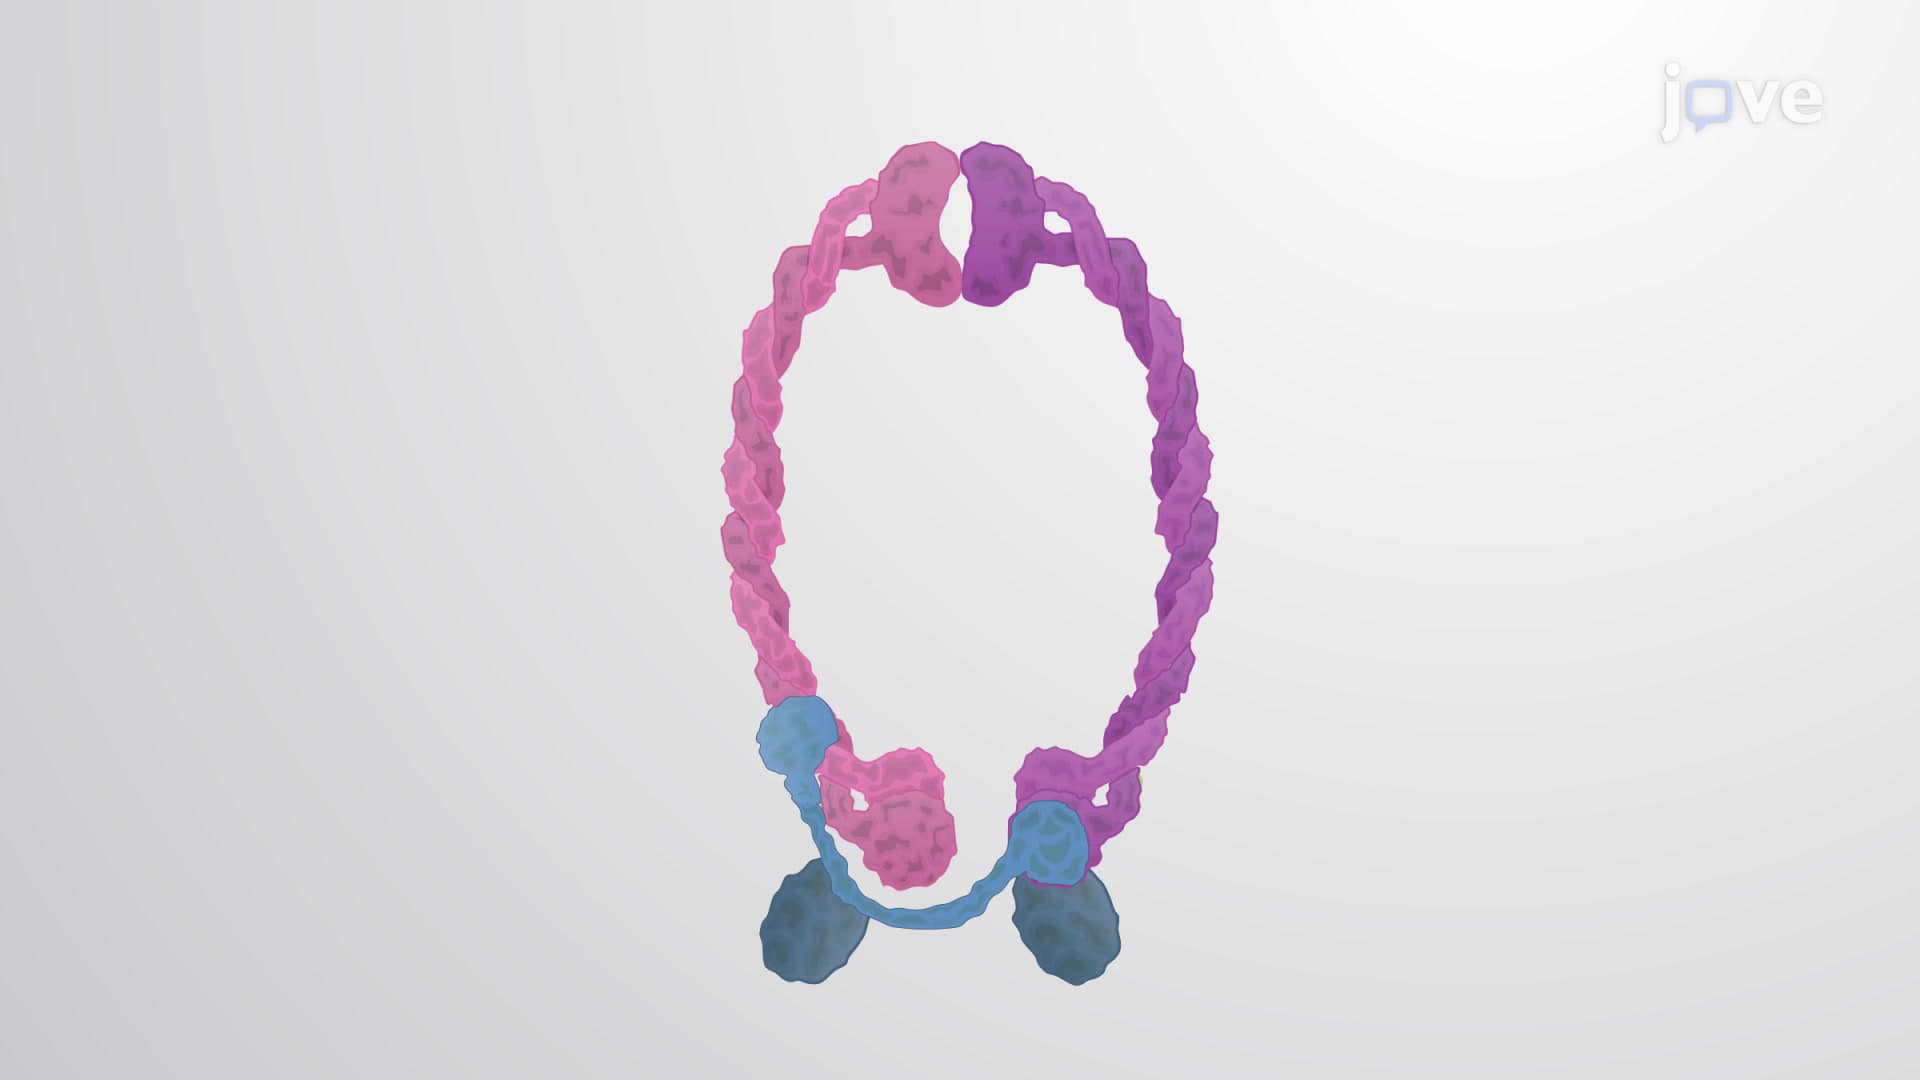
Condensins
3.4K
Condensins are large protein complexes that use ATP to fuel the assembly of chromosomes during mitosis. They transform the tangled, shapeless mass of post-interphase DNA into individualized chromosomes by compacting, organizing, and segregating chromosomal DNA.
The plant and animal cells contain two types of condensin complexes—condensin I and condensin II. Both complexes have five subunits: two SMC (Structural Maintenance of Chromosomes) subunits, a kleisin subunit, and two HEAT-repeat...
The plant and animal cells contain two types of condensin complexes—condensin I and condensin II. Both complexes have five subunits: two SMC (Structural Maintenance of Chromosomes) subunits, a kleisin subunit, and two HEAT-repeat...
3.4K