コロナウイルスのスパイクHR2ドメイン: 膜融合で注目される謎のプレイヤー?
Elena T Aliper1, Roman G Efremov2
1Shemyakin-Ovchinnikov Institute of Bioorganic Chemistry, Russian Academy of Sciences, 16/10 Miklukho-Maklaya St., Moscow 117997, Russian Federation.
Biochimica et biophysica acta. Biomembranes
|August 21, 2025

まとめ
コロナウイルスのスパイクタンパク質
科学分野:
- ウイルス学
- バイオ物理学
- コンピュータ生物学
背景:
- コロナウイルスのスパイクタンパク質は,膜融合を媒介することでウイルスの侵入を容易にします.
- HR1とHR2は,再折りや膜融合に関与するスパイクタンパク質内の重要なドメインです.
- 膜相互作用におけるHR2の正確な役割を理解することは,ウイルスの融合メカニズムを解読する上で極めて重要です.
研究 の 目的:
- SARS-CoV-2のスパイクHR2ドメインとモデル膜の相互作用を調査する.
- 異なる文脈でHR2の構造的行動と膜結合特性を解明する.
- HR2の膜活性に対するモジュラー構造と制御の可能性を探る.
主な方法:
- 分子ダイナミクスシミュレーションを含む計算手法
- 脂質二層モデルによるシミュレーション
- 分子防水力 (MHP) のマッピング
主要な成果:
- HR2だけでは,モデル膜との相互作用は最小でした.
- 膜域 (TMD) と/またはHR2前断片との共発は,HR2の膜結合を著しく強化した.
- HR2はすべてのシミュレーション条件下でトライメリックコイルドコイル構造を維持しました.
- MHPマッピングは,HR2内の膜活性モチーフを明らかにした.
- 活性モチーフのみを含む切断されたHR2は,膜親和性が増加した.
結論:
- HR2の膜活動は,側面の領域によって制御され,潜在的にマスクされ,モジュール構造を示唆します.
- TMDとpreHR2のような隣接ドメインは,分割後の因子とともに,HR2の機能を強化する可能性があります.
- このモジュール式設計は,ウイルスの融合時にHR2の膜活性を正確に制御することを可能にします.
さらに関連する動画
 07:53
A Fluorogenic Peptide Cleavage Assay to Screen for Proteolytic Activity: Applications for coronavirus spike protein activation
Published on: January 9, 2019
33.3K
 06:39
High-throughput Confocal Imaging of Quantum Dot-Conjugated SARS-CoV-2 Spike Trimers to Track Binding and Endocytosis in HEK293T Cells
Published on: April 21, 2022
3.2K
関連する概念動画
 01:43
SNAREs and Membrane Fusion
11.0K
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
11.0K
 00:59
Mechanisms of Membrane Domain Formation
3.1K
Different physical properties of lipids and proteins allow them to localize and form distinct islands or domains in the membrane. Some membrane domains are formed due to protein-protein interactions, whereas others are formed due to the presence of specific lipids such as sphingolipids and sterols—for example, large proteins, such as bacteriorhodopsin, aggregate and create distinct domains.
Another mechanism for membrane domain formation involves membrane proteins interacting with...
Another mechanism for membrane domain formation involves membrane proteins interacting with...
3.1K
 01:18
Membrane Domains
5.7K
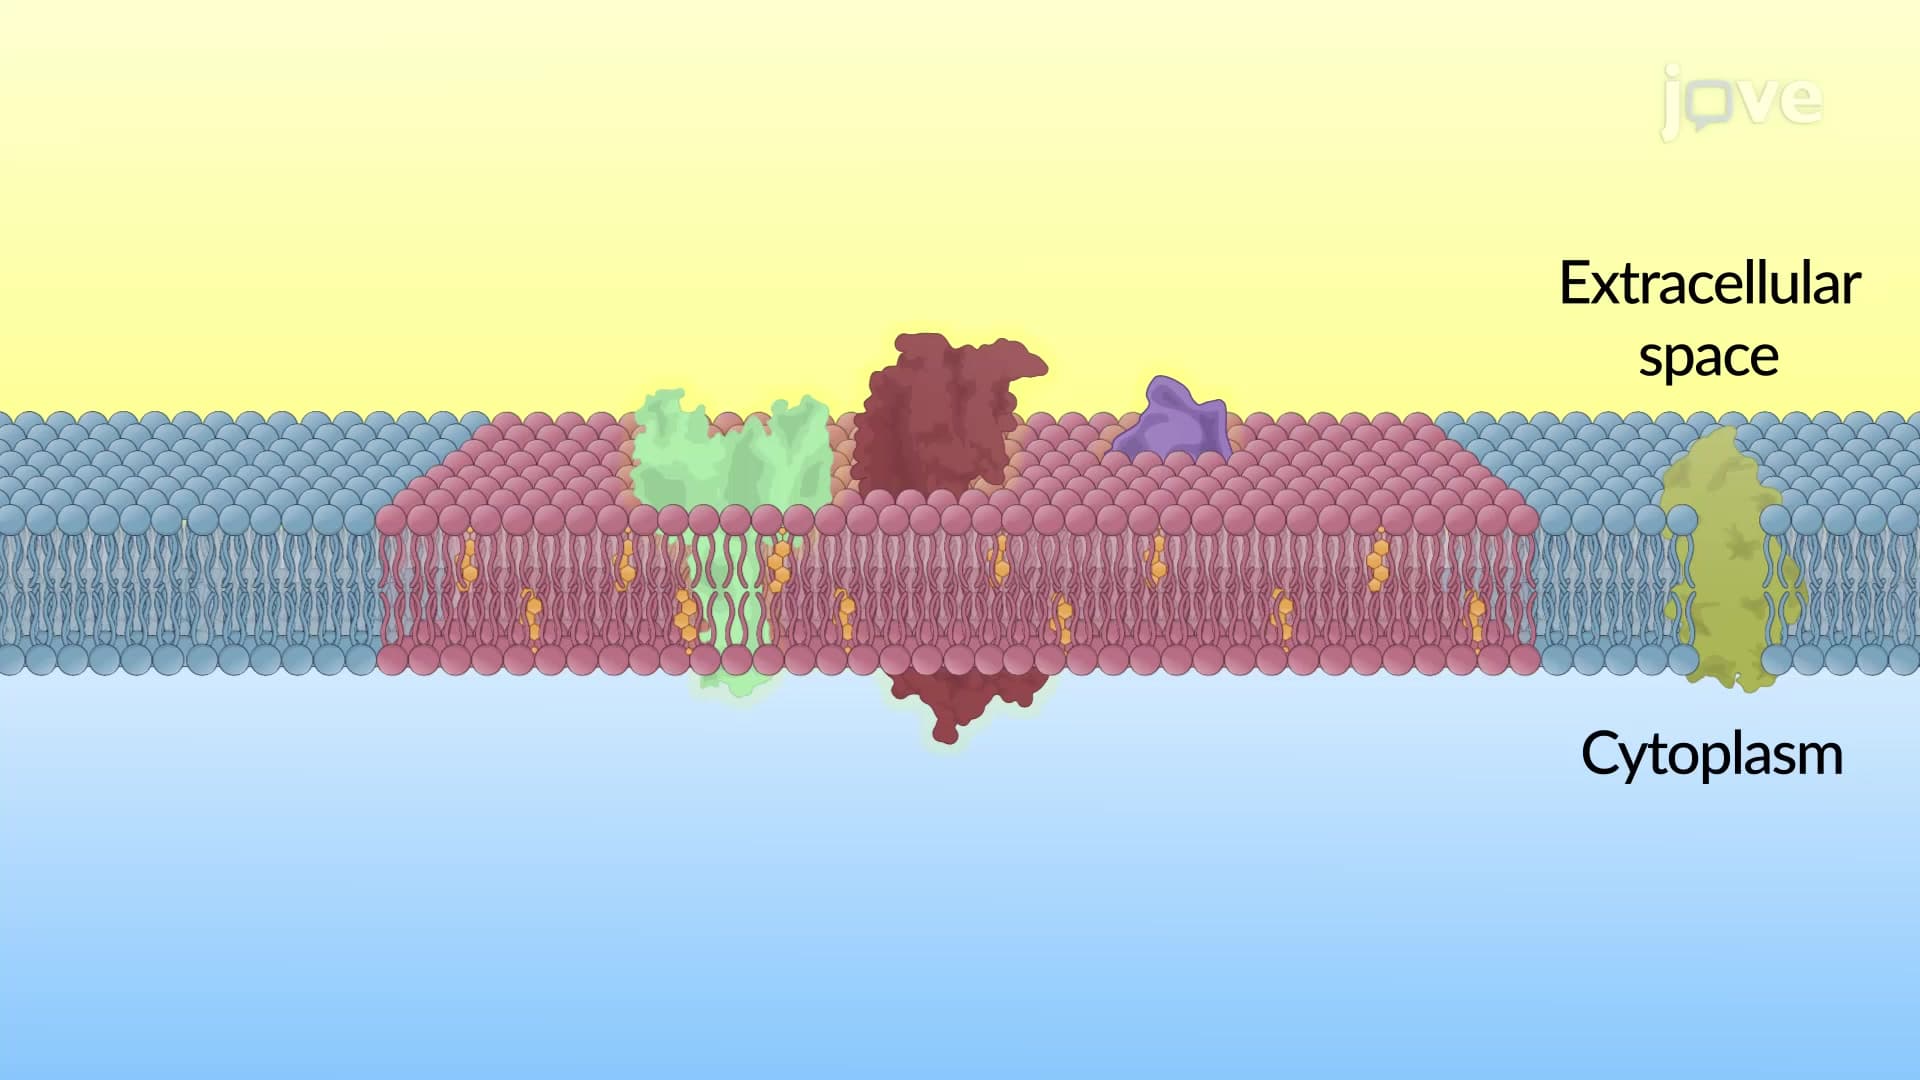
The membrane domains concentrate specific lipids and proteins at one place within the membrane, which helps in cell signaling, adhesion, and other critical cellular processes. These domains can differ in size, composition, function, and lifespan.
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the...
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the...
5.7K
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
11.7K
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
11.7K
 01:28
Protein Translocation Machinery on the ER Membrane
4.9K
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
4.9K
 01:25
Rab Cascades
2.7K
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
2.7K