
キネシン-1 自動阻害チューン モーター・アンサンブルによる貨物輸送
Brandon M Bensel1, Samantha B Previs1, Patricia M Fagnant1
1Department of Molecular Physiology and Biophysics, University of Vermont Larner College of Medicine, Burlington, VT 05405.
Biophysical journal
|September 3, 2025

まとめ
キネシン-1モーターは,微小管の交差点を通じた細胞内膀輸送を調節する負荷を運ぶときに部分的な自己抑制を示します. この微調整は 細胞機能に影響を及ぼし 適切な膀配送を保証します
科学分野:
- 細胞生物学
- 分子モーター
- バイオ物理学
背景:
- 細胞内輸送はキネシン-1のようなモータータンパク質に依存し マイクロチューブルに沿って貨物を移動させます
- キネシン-1の活動は自己抑制によって調節されていることが知られているが,複雑なマイクロチューブルネットワークを通じて貨物輸送におけるその役割は不明であった.
研究 の 目的:
- 貨物に結合したときに,キネシン-1が自己抑制を示すかどうかを調査する.
- この自己抑制が,3D微小管の交差点を通じた膀輸送を制御するかどうかを in vitro で決定する.
主な方法:
- 結合KLC (KinΔC) のキネシン-1モーターによるリポソーム輸送と構成的に活性なキネシン-1 (K543) の比較
- 3D微小管の交差点における膀の行動 (終結,直進,回転) の分析
- 両方のエンジンの走行長,脱離力,およびマイクロチューブル着陸率の測定.
- 小分子自己抑制剤のキネソールによるシリコモデリングと実験で
主要な成果:
- 3D微小管の交差点では,アクティブキネシン-1 (K543,12%) に比べて,カーゴ・バインドキネシン-1 (KinΔC) の終結率が著しく高かった.
- KinΔCは走行距離,脱離力,および微小管着陸率の減少を示し,微小管の関与を減少させた.
- キネソール治療は,KinΔCに対する微小管の関与を回復させ,自己抑制の役割を確認した.
結論:
- 荷物に結合したキネシン-1モーターの部分的自己抑制は,膀輸送の調節に重要な役割を果たします.
- 微小管の交差点での生理学的要求に適応することを可能にします
- キネシン-1の調節を理解することは,細胞内輸送効率と忠誠性を理解する鍵です.
関連する概念動画
 01:43
The Movement of Organelles and Vesicles
4.7K
In eukaryotic cells, cytoskeletal filaments such as actin, microtubules, and intermediate filaments form a mesh-like cytoskeletal network. These filaments serve as tracks for transporting cellular cargo. Specialized motor proteins use the chemical energy stored in adenosine triphosphate (ATP) for this transport. During interphase, microtubules are polarized, with the plus-end towards the cell periphery and the minus-end towards the cell center. Two microtubule-associated motor proteins,...
4.7K
 01:32
Microtubule Associated Motor Proteins
8.5K
Eukaryotic cells have different motor proteins for transporting various cargo within the cell. These motor proteins differ based on the filament they associate with, the direction they move within the cell, and the type of cargo they transport. Motor proteins that associate with microtubules are known as microtubule-associated motor proteins. There are two families of microtubule-associated motor proteins —Kinesins and Dyneins. Both these proteins assist in the transport of cellular...
8.5K
 01:45
Destabilization of Microtubules
2.8K
The destabilization of microtubules can occur during different stages of the microtubule lifecycle, such as nucleation or elongation. It can take place at either end of the microtubule or in the microtubule lattices as a whole. The lifespan of individual microtubules within a cell varies according to the cell type and stage of the cell cycle. During interphase, the lifespan of the microtubule is about 30 minutes, while during cell division, it is about 15 minutes. In axonal microtubules of...
2.8K
 01:33
Coat Assembly and GTPases
3.6K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.6K
 01:39
Anaphase A and B
4.2K
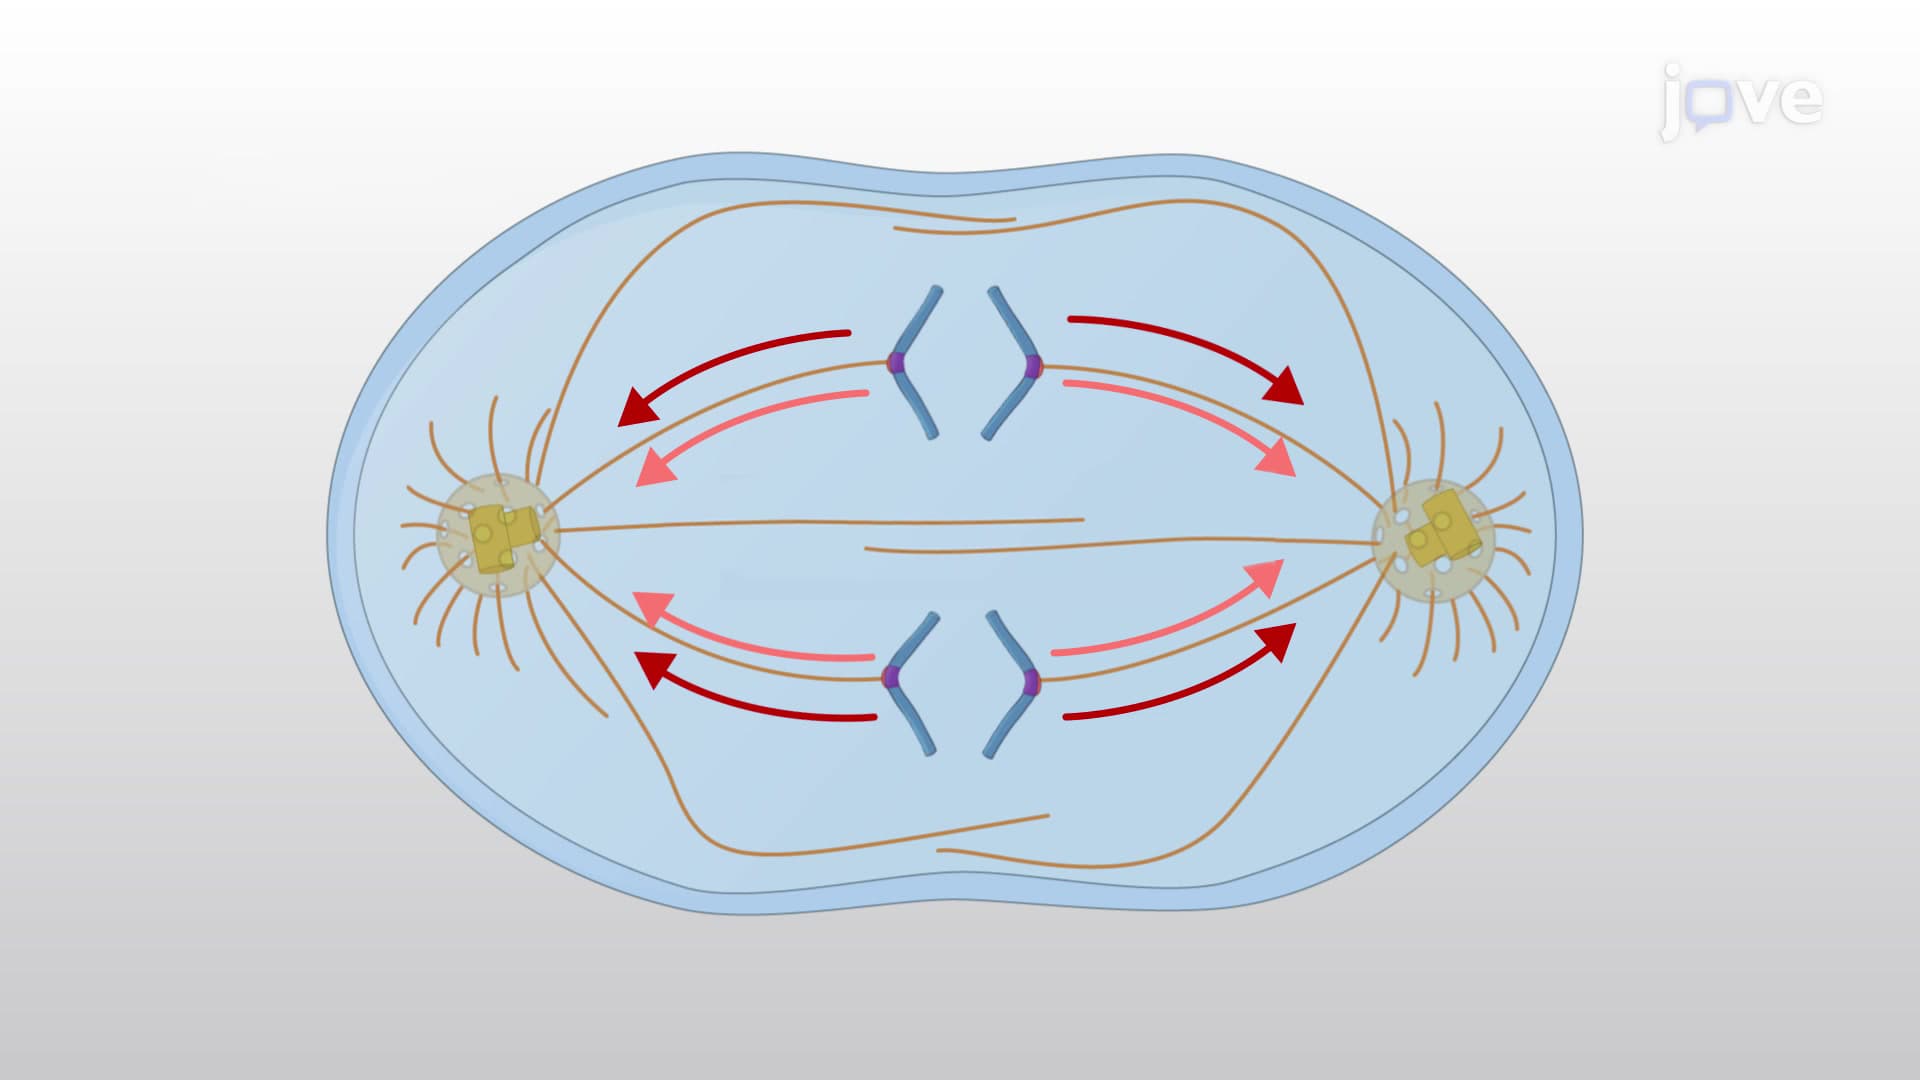
Microtubules form through the end-to-end polymerization of tubulin heterodimers. Kinetochore microtubules originate from the spindle poles, and their plus-ends connect with the kinetochores on sister-chromatids. Ndc80 protein complexes, present on the kinetochore, form low-affinity links with the plus end of these kinetochore microtubules.
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
4.2K
 01:05
Mechanism of Ciliary Motion
3.9K
The ciliary structures were first seen in 1647 by Antonie Leeuwenhoek while observing the protozoans. In lower organisms, these appendages are responsible for cell movement, while in higher organisms, these appendages help in the movement of the extracellular fluids within the body cavities.
The cilia are made up of microtubules in a 9+2 arrangement, with nine microtubule doublet ring bundles, surrounding a pair of central singlet microtubule bundles. The doublet microtubule bundles are...
The cilia are made up of microtubules in a 9+2 arrangement, with nine microtubule doublet ring bundles, surrounding a pair of central singlet microtubule bundles. The doublet microtubule bundles are...
3.9K