関連する実験動画
Updated: Sep 9, 2025
20:28
A Toolkit to Enable Hydrocarbon Conversion in Aqueous Environments
Published on: October 2, 2012
14.2K
C. reinhardtii の低炭素誘導2/脂肪酸不飽和4ロクスは,プラスティド過酸化物の位置とトランス脂肪酸の産生を制御する
Timothy J Nicodemus1, Stefan Schmollinger1,2, John E Froehlich1,2
1MSU-DOE Plant Research Laboratory.
Plant physiology
|September 3, 2025

まとめ
植物と藻類は,脂質ベースのメカニズムを使用して,光合成膜の損傷を感知し,それに反応することができます. これは低炭素誘導性2 (LCI2) タンパク質と脂肪酸不飽和酵素4 (FAD4) 遺伝子を含み,膜修復と反応性酸素種緩和に不可欠です.
科学分野:
- 植物生物学
- 分子生物学
- 生物化学
背景:
- 脂質膜の光合成複合体はエネルギー変換に不可欠であるが,反応性酸素種 (ROS) から損傷を受けやすい.
- 環境的ストレスにより ROSの蓄積が増加し,光合成機能が損なわれる可能性があります.
- 植物と藻類は,光合成膜の損傷を検出し,それに反応するために,脂質ベースのセンサーメカニズムが提案されています.
研究 の 目的:
- クラミドモナス・レインハーディの脂質ベースのセンサーメカニズムの分子基礎を調査し,光合成膜の損傷について調べる.
- 低炭素誘導体2 (LCI2) と脂肪酸不飽和酵素4 (FAD4) の作用をこの感知および応答経路で調査する.
- LCI2とFAD4のユニークな転写調節と機能的リンクを理解する.
主な方法:
- Chlamydomonas reinhardtiiにおけるLCI2/FAD4の位置とその差異的なスプライシングの分析
- FAD4によって生成される脂肪酸の特徴とその局所化.
- LCI2による酵素活性の調査
主要な成果:
- LCI2とFAD4は,共通のN末端を共有し,差分スプライシングで同じ場所から派生しています.
- FAD4は,クロロプラストのフォスファティジルグリセロールにのみ存在するトランス二重結合を持つユニークな16炭素脂肪酸を合成します.
- LCI2はペロキシダースの活性を膜に誘導し,ROSの緩和に役立ちます.
結論:
- LCI2 / FAD4ロクスは,光合成膜損傷を感知するための規制インターフェースを提供します.
- この位置は,独特の膜脂肪酸の生物合成とROS緩和酵素の生成を調整する.
- このメカニズムは 細胞が環境ストレスに反応し 光合成機能を維持することを可能にします
関連する概念動画
 01:27
C4 Pathway and CAM
46.2K
Most plants use the C3 pathway for carbon fixation. However, some plants, such as sugar cane, corn, and cacti that grow in hot conditions, use alternative pathways to fix carbon and conserve energy loss due to photorespiration. Photorespiration is the process that occurs when the oxygen concentration is high. Under such conditions, the rubisco enzyme in the Calvin cycle binds O2 instead of CO2, which halts photosynthesis and consumes energy.
C4 Pathway
The C4 pathway is used by plants such as...
C4 Pathway
The C4 pathway is used by plants such as...
46.2K
 01:46
The Calvin Benson Cycle
4.7K
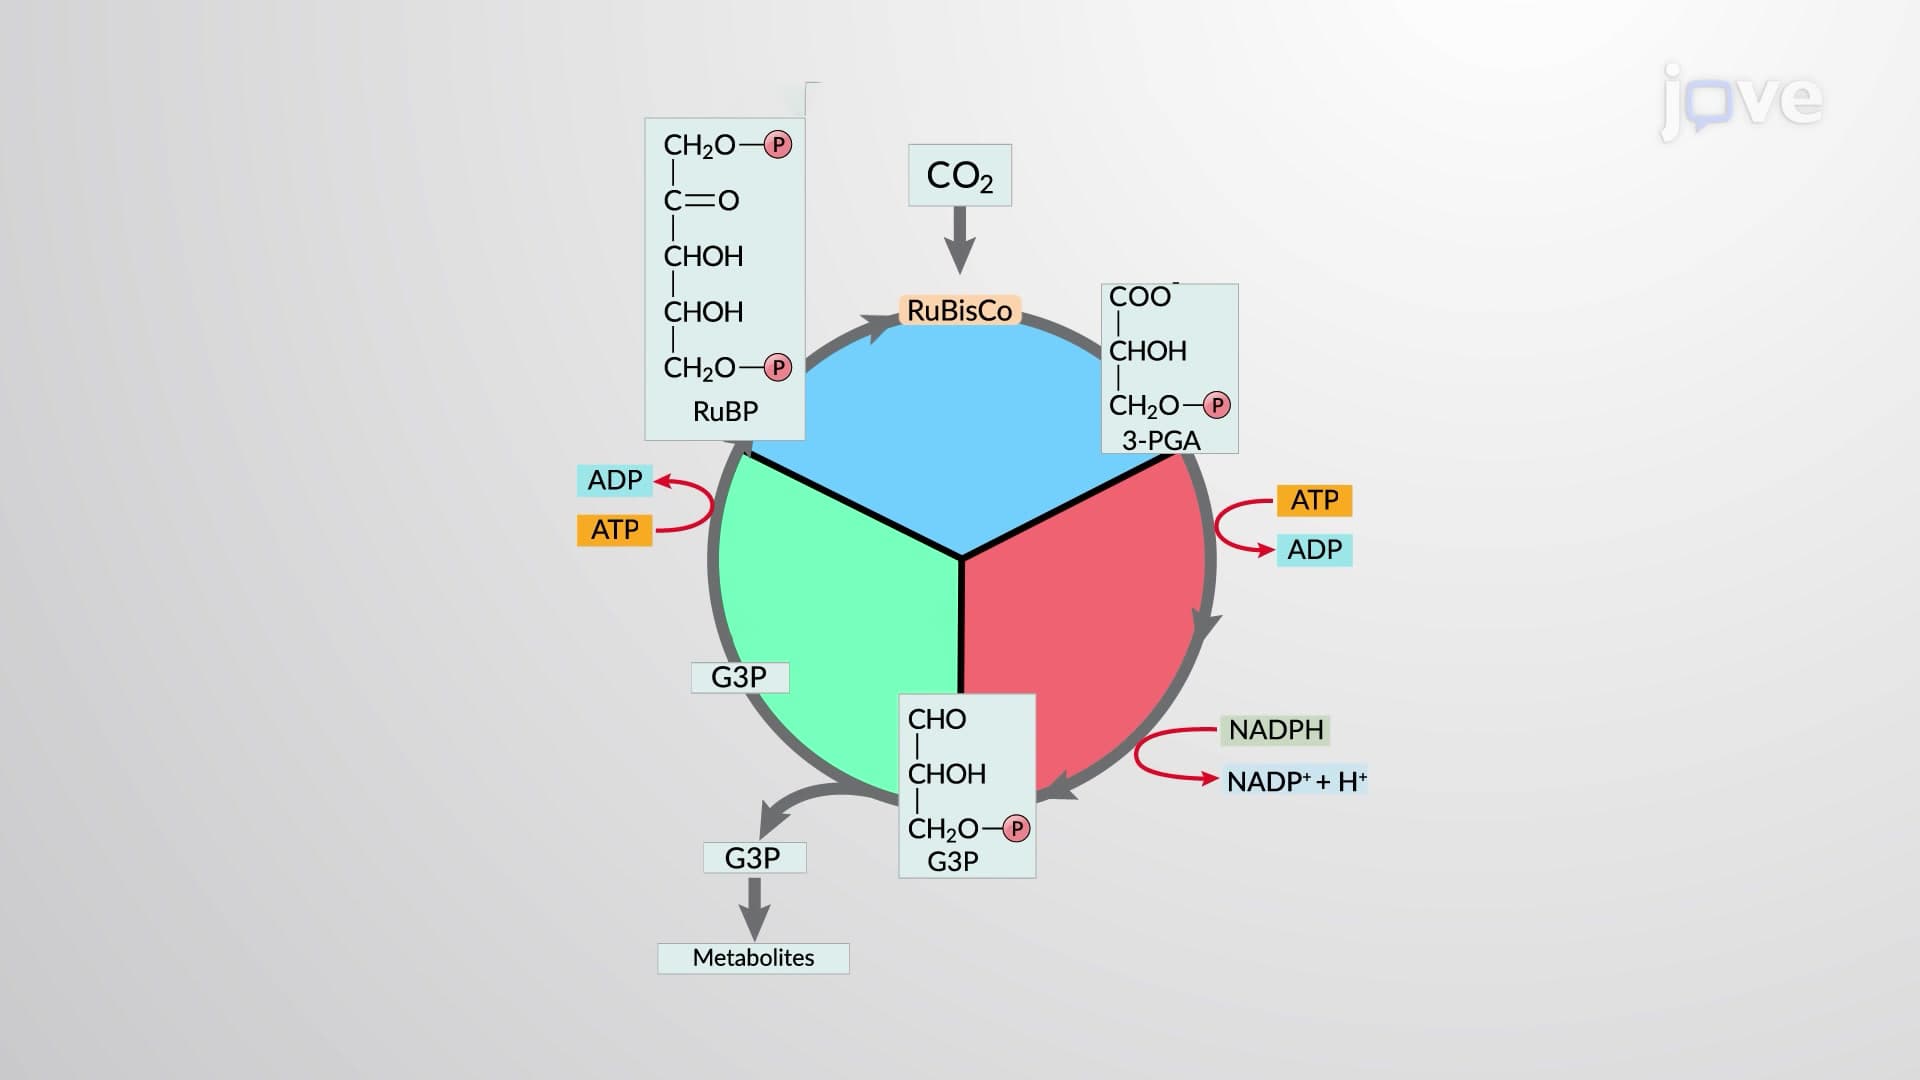
Ribulose 1,5- bisphosphate carboxylase/oxygenase (RuBisCo) is a critical enzyme that catalyzes carbon dioxide assimilation during photosynthesis. However, it is an inefficient enzyme, having an extremely slow catalytic rate. A typical enzyme can process about a thousand molecules per second; however, RuBisCo fixes only around three-carbon dioxides per second. Photosynthetic cells compensate for this slow rate by synthesizing very high amounts of RuBisCo, making it the most abundant single...
4.7K
 01:28
Carbon-dioxide Fixation
83
Carbon dioxide fixation in prokaryotes enables the assimilation of inorganic carbon into organic molecules, supporting biosynthetic pathways, sustaining ecosystems, and contributing to the global carbon cycle. It also has industrial applications in carbon capture and bioproduct synthesis. Autotrophic organisms rely on this process to utilize CO₂ as a carbon source in diverse environments.The Calvin CycleThe Calvin cycle is the most widespread carbon fixation mechanism, primarily used by...
83
 01:28
Overview of Fatty Acid Metabolism
31.7K
Lipids also are sources of energy that power cellular processes. Like carbohydrates, lipids are composed of carbon, hydrogen, and oxygen, but these atoms are arranged differently. Most lipids are nonpolar and hydrophobic. Major types include fats and oils, waxes, phospholipids, and steroids.
Fatty acids are catabolized in a process called beta-oxidation, which takes place in the matrix of the mitochondria and converts their fatty acid chains into two-carbon units of acetyl groups. The acetyl...
Fatty acids are catabolized in a process called beta-oxidation, which takes place in the matrix of the mitochondria and converts their fatty acid chains into two-carbon units of acetyl groups. The acetyl...
31.7K
 01:25
Lipid Catabolism
165
Triglycerides serve as crucial long-term energy storage molecules in microorganisms, providing a dense source of metabolic energy. Their breakdown is mediated by lipases, which hydrolyze triglycerides into glycerol and free fatty acids. Each of these components follows distinct metabolic pathways, ultimately contributing to ATP synthesis and cellular energy homeostasis.Glycerol MetabolismGlycerol, released from triglyceride hydrolysis, is phosphorylated by glycerol kinase to form...
165
 01:18
Protein Transport to the Inner Chloroplast Membrane
2.1K
Proteins targeted to the inner chloroplast membrane, or plastid proteins, are transported by two general pathways: the stop-transfer and the re-insertion or post-import pathways. Most plastid proteins carry N-terminal transit sequences and internal import sequences targeting it to the specific chloroplast subcompartment. Proteins targeted by the stop-transfer pathway have internal hydrophobic sequences that inhibit their translocation into the stroma. As a result, these precursors are arrested...
2.1K