
Fmr1ノックアウトは,背中側タラモコルチカルニューロンのHCNチャネル活性低下によって,複数の内在的特性を破壊する
Gregory J Ordemann1,2, Polina Lyuboslavsky1,2, Alena Kizimenko1,2
1Department of Neurology, Dell Medical School at The University of Texas at Austin, Austin, Texas, USA.

マウスの脆弱X症候群 (Fragile X syndrome,FXS) は,前頭前皮質に発射する中背のタラムスのニューロンのHCNチャネル機能を損なう. この障害は神経のリズムに 影響を及ぼし 認知や社会的行動に 影響を及ぼします
科学分野:
- 神経科学
- 遺伝学
- チャネル病
背景:
- 脆弱X症候群 (Fragile X syndrome,FXS) は,FMR1遺伝子の高甲基化によって引き起こされる神経発達障害であり,FMRPタンパク質の欠乏につながります.
- FMRPタンパク質は脳回路に不可欠なイオンチャネル活動を含む様々な細胞機能を調節する.
- タラモコルチカル経路,特に中背のタラムス (MD) と中部前頭皮質 (mPFC) との接続は,FXSの病理生理学に関与しています.
研究 の 目的:
- Fmr1遺伝子ノックアウトが,mPFCに発射するMDタラミックニューロンの固有細胞特性への影響を調査する.
- Fmr1欠乏がMD→mPFCニューロンのハイパーポラライゼーション活性化およびサイクルヌクレオチドゲート (HCN) チャンネル機能にどのように影響するかを決定する.
主な方法:
- 野生型とFmr1ノックアウトの雄性マウスの逆行式ラベルとex vivo全細胞電気生理学を使用した.
- 側 (MD-L) と中部 (MD-M) のMDニューロンにおけるHCN媒介の膜反応を含む細胞内特性を調べた.
主要な成果:
- Fmr1のノックアウトにより,HCNによる電圧の低下とMD-Lニューロンの膜の超極化が発生した.
- Fmr1のノックアウトマウスの複合爆発と低値のスパイクの両方で,リバウンドスパイクのタイミングの遅延が観察されました.
- MD-L→mPFCニューロンのHCNチャネル活性低下は膜ポテンシャル調節を阻害し,潜在的にタロモコルチカルリズム伝播を妨害する.
結論:
- Fmr1欠乏はMDのタラミックニューロンのHCNチャネル機能を変化させ,タラモ皮質回路の活動に影響を与えます.
- これらの細胞の変化は,FXSで観察された認知および社会的欠陥の根底にある可能性があります.
- これらのメカニズムの理解は,FXSおよび関連するタラミックリズム障害の治療戦略にインパクトを与える可能性があります.
さらに関連する動画
 09:17
Combining Optogenetics with Artificial microRNAs to Characterize the Effects of Gene Knockdown on Presynaptic Function within Intact Neuronal Circuits
Published on: March 14, 2018
 11:10
Dissecting Cell-Autonomous Function of Fragile X Mental Retardation Protein in an Auditory Circuit by In Ovo Electroporation
Published on: July 6, 2022
関連する概念動画
 02:54
Nucleosome Remodeling
Nucleosome remodeling complex
Eukaryotic cells have specialized enzymes called ATP-dependent nucleosome remodeling enzymes. These enzymes...
 02:37
Restarting Stalled Replication Forks
 02:27
Nonsense-mediated mRNA Decay
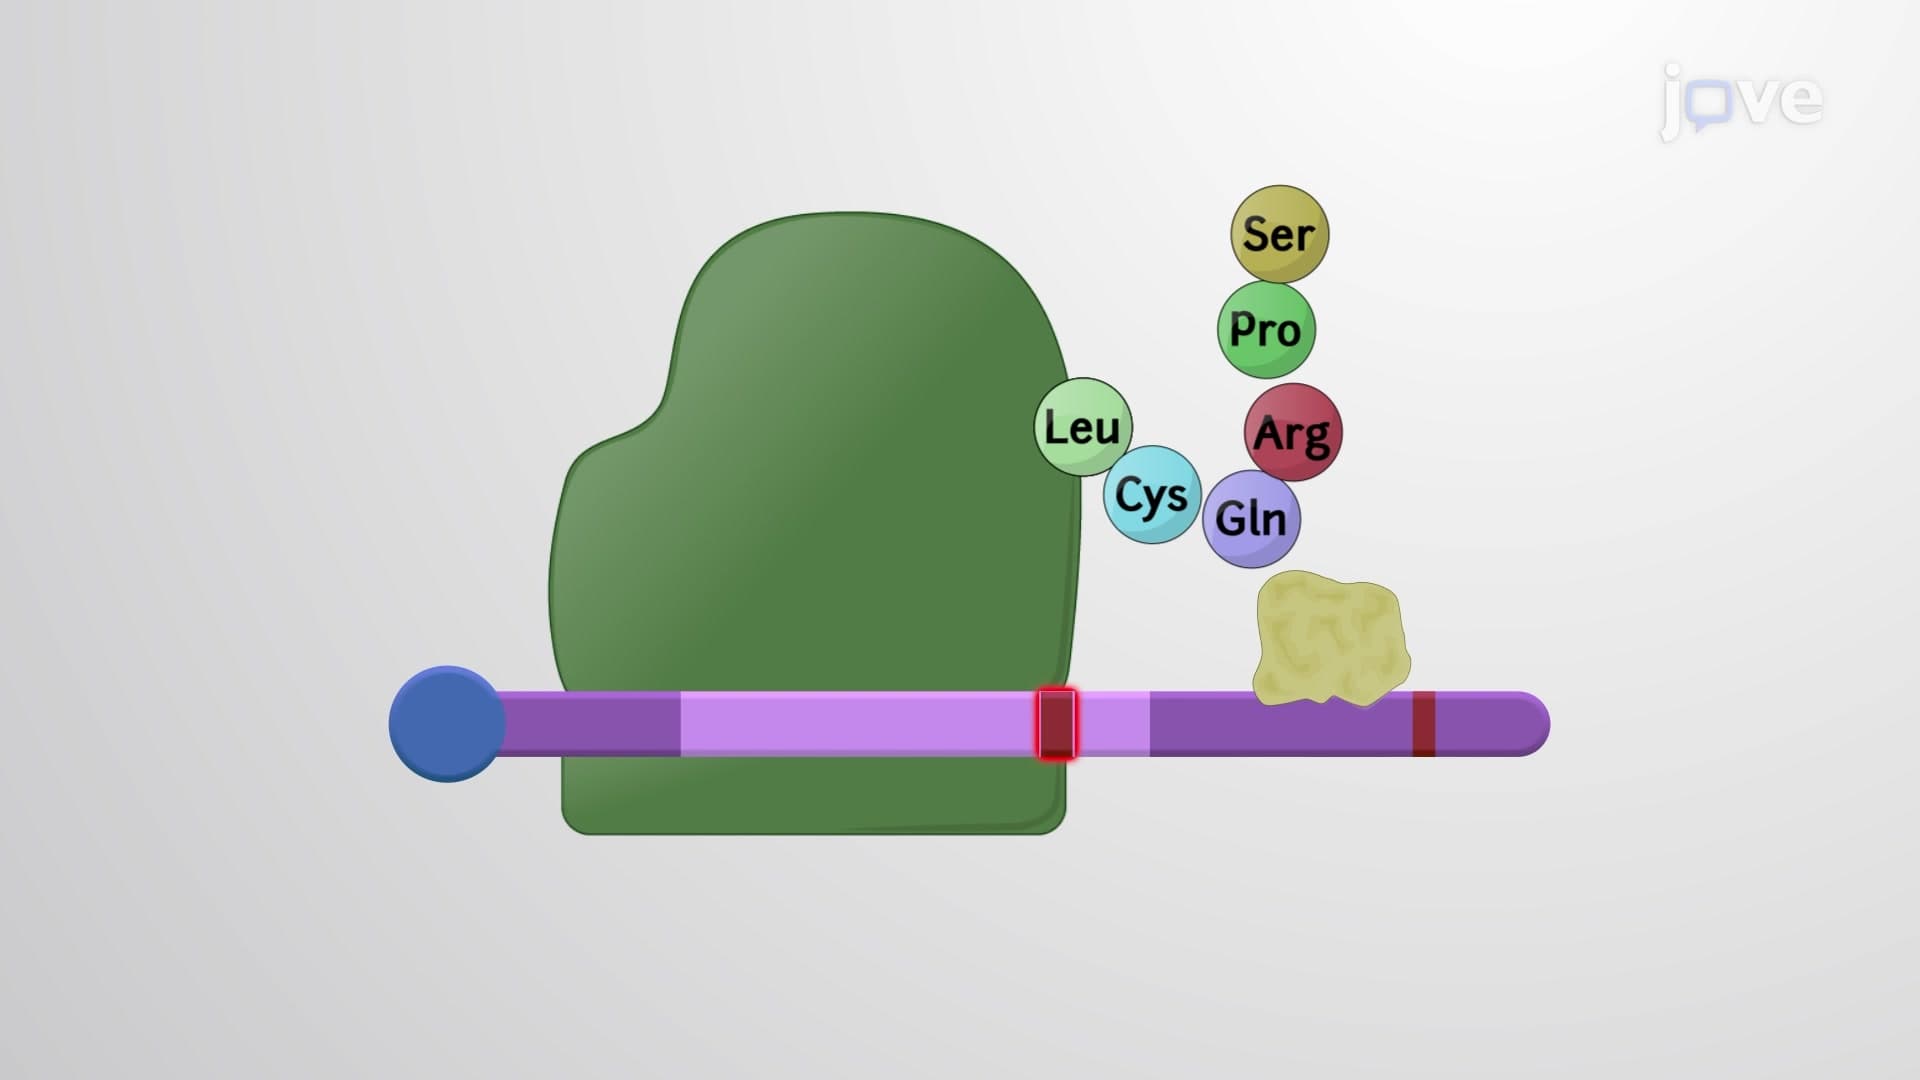
Usually, Upf3 binds to an Exon Junction Complex (EJC) at mRNA splice sites. If a ribosome fully translates the mRNA,...
 02:26
NF-κB-dependent Signaling Pathway
NF-κB-dependent Signaling Mechanism
The heterodimer of NF-κB...
 01:32
Export of Misfolded Proteins out of the ER
02:26NF-kB-dependent Signaling Pathway
NF-κB-dependent Signaling Mechanism
The heterodimer of NF-κB...