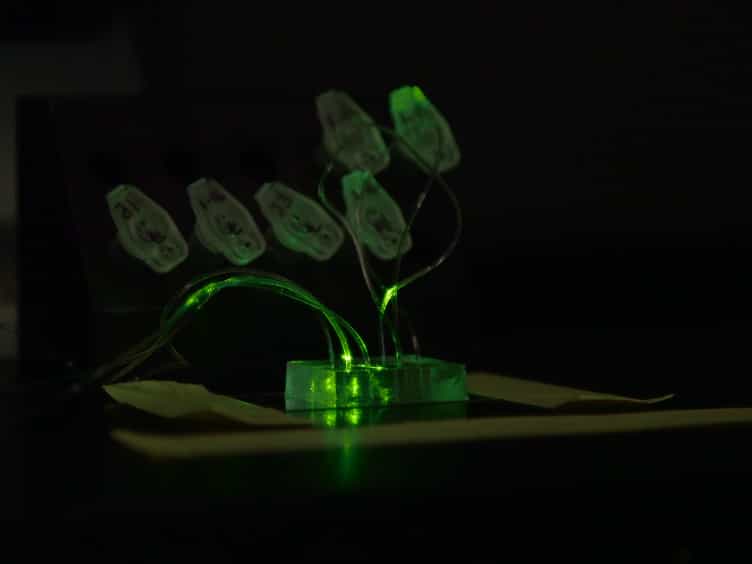

目标膜的synaptotagmin介导的曲是Ca(2+) 调节的融合过程中的关键步骤
Enfu Hui1, Colin P Johnson, Jun Yao
1Howard Hughes Medical Institute, USA.
Cell
|August 26, 2009

概括
通过Synaptotagmin-I (syt) 蛋白质介导的膜曲对于加速表细胞突变期间的膜融合至关重要. 这项研究表明,syt.
科学领域:
- 细胞生物学 细胞生物学
- 膜生物物理学 膜生物物理学
- 分子神经科学分子神经科学
背景情况:
- 囊泡与等离子体膜融合的过程 - - 细胞外生化,对于细胞通信至关重要.
- 在Ca2+触发的膜曲中,synaptotagmin-I (syt) 的作用及其对聚变动学的贡献仍在争论中.
- 之前的研究使用了具有预曲囊泡或非选择性细胞突变的复合系统,限制了关于膜曲的直接作用的结论.
研究的目的:
- 为了调查synaptotagmin-I的膜曲活性是否直接驱动目标膜发育,以加速融合.
- 为了确定膜曲率对syt的促进融合功能的影响.
主要方法:
- 利用具有不同程度膜曲率的脂质体来测试突触胺-I功能.
- 采用了管道缺陷的突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变.
- 评估了具有或没有添加N-BAR域的SNARE载体脂质体之间的融合效率.
主要成果:
- 一个管道缺陷的突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突变突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出突出
- 这种突变显示出相对平坦的脂质体与相对平坦的脂质体的融合活性显著减少.
- 外源的N-BAR域诱导的膜曲挽救了管道缺陷的突变突变的融合缺陷 synaptotagmin-I 在平面膜上.
结论:
- Synaptotagmin-I的膜曲能力对于在外细胞形成过程中有效的膜融合至关重要.
- 局部膜曲,而不仅仅是Ca2+) 结合,是一个关键的机制,通过它,synaptotagmin-I加速融合.
- 这一发现澄清了突触胺-I在膜贩运中的作用背后的生物物理机制.
更多相关视频
相关概念视频
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:43
SNAREs and Membrane Fusion
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:15
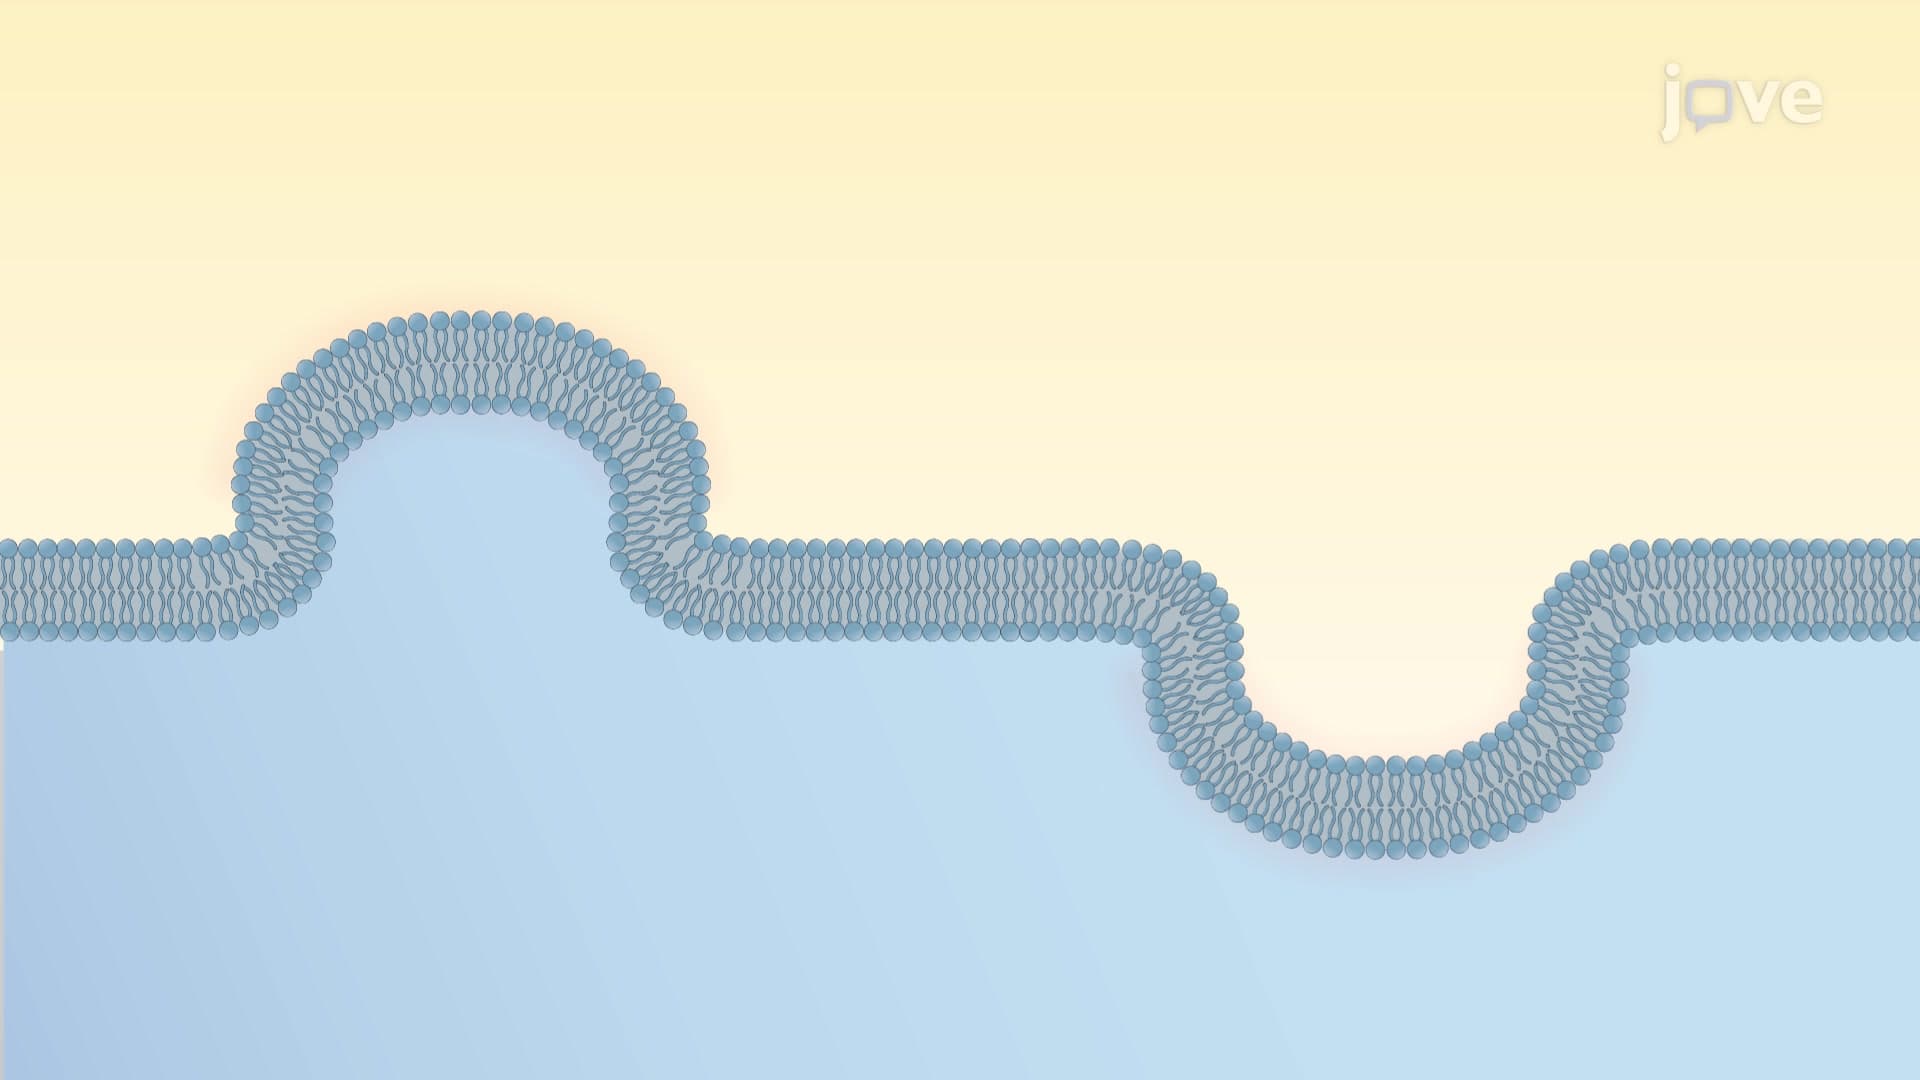
Mechanisms of Membrane-bending
The living membranes are flexible due to their fluid mosaic nature; however, their bending into different shapes is an active process regulated by specific lipids and proteins. The membrane bending can be transient as seen in vesicles or stable for a long time as in microvilli. Cells regulate the size, location, and duration of the membrane curvature.
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:16
Calmodulin-dependent Signaling
Calmodulin (CaM) is a calcium-binding protein in eukaryotes that controls various calcium-regulated cellular processes. It has four calcium-binding sites that bind calcium to form the calcium-calmodulin ( Ca2+-CaM) complex. GPCR stimulation increases the calcium levels in the cells that bind to CaM and induces a conformational change.
The Ca2+-CaM complex does not have enzymatic activity by itself. Instead, the complex binds downstream target proteins, including membrane proteins or enzymes,...
The Ca2+-CaM complex does not have enzymatic activity by itself. Instead, the complex binds downstream target proteins, including membrane proteins or enzymes,...
 01:25
Rab Cascades
Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
 01:45
Tail-anchoring of Proteins in the ER Membrane
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...