确定F-actin作为微生物诱导的GTPase极性电路中的动态枢纽
Robert C Orchard1, Mark Kittisopikul, Steven J Altschuler
1Department of Microbiology, University of Texas Southwestern Medical Center, Dallas, TX 75390, USA.
Cell
|February 21, 2012

概括
细菌病原体利用与F-actin相互作用的关氨酸核酸交换因子 (GEF) 劫持细胞极性. 这种相互作用驱动Cdc42 GTPase极化,揭示了哺乳动物和细菌细胞极性的保存机制.
科学领域:
- 细胞生物学 细胞生物学
- 生物化学 生物化学
- 微生物学 微生物学
背景情况:
- 细胞极性对哺乳动物细胞功能至关重要,并由复杂的信号网络调节.
- 细菌病原体可以操纵这些宿主细胞通路,以造福他们自己.
研究的目的:
- 揭示哺乳动物细胞极性和细菌病原学的基本原理.
- 调查肠病原性大肠杆菌瓜核酸交换因子 (GEF) 在Cdc42 GTPase信号传递中的作用.
主要方法:
- 开发一个可操作的实验和理论模型.
- 使用了GEF地图的合成衍生品.
- 运用数学建模来分析actin动态和反循环.
主要成果:
- 发现Cdc42 GTPase信号转导是由Map GEF和F-actin之间的相互作用控制的.
- 证明了actin动力学和Map依赖的正反循环在等离子体膜上自发地极化Cdc42.
- 表明,重新连接信号电路以刺激β-整合素,可以使Cdc42在响应细胞外线索时发生偏振.
结论:
- 提出了一个细胞极性分子途径,以GEFs和F-actin之间的相互作用为中心.
- 这种机制很可能在各种生物系统中存在并起作用,包括哺乳动物细胞和细菌感染.
相关概念视频
 02:14
GTPases and their Regulation
Guanine nucleotide-binding proteins (G-proteins), also known as GTPases, are a superfamily of proteins that regulate many cellular processes, such as cell signaling, vesicular transport, and the regulation of cell shape and motility. Mutation or dysfunction of these proteins can lead to disease. There are around 40,000 known G-proteins that can broadly be classified into two groups ‒ small G-proteins consisting of a single domain and large multi-domain G-proteins.
Large G-proteins, also known...
Large G-proteins, also known...
 01:14
Rab Proteins
Rab proteins constitute the largest family of monomeric GTPases, of which 70 members are present in humans. Rab proteins and their effectors regulate consecutive stages of vesicle transport such as vesicle transport, docking, and fusion to the correct recipient membrane.
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
02:14GTPases and their Regulation
Guanine nucleotide-binding proteins (G-proteins), also known as GTPases, are a superfamily of proteins that regulate many cellular processes, such as cell signaling, vesicular transport, and the regulation of cell shape and motility. Mutation or dysfunction of these proteins can lead to disease. There are around 40,000 known G-proteins that can broadly be classified into two groups ‒ small G-proteins consisting of a single domain and large multi-domain G-proteins.
Large G-proteins, also known...
Large G-proteins, also known...
 01:24
Small GTPases - Ras and Rho
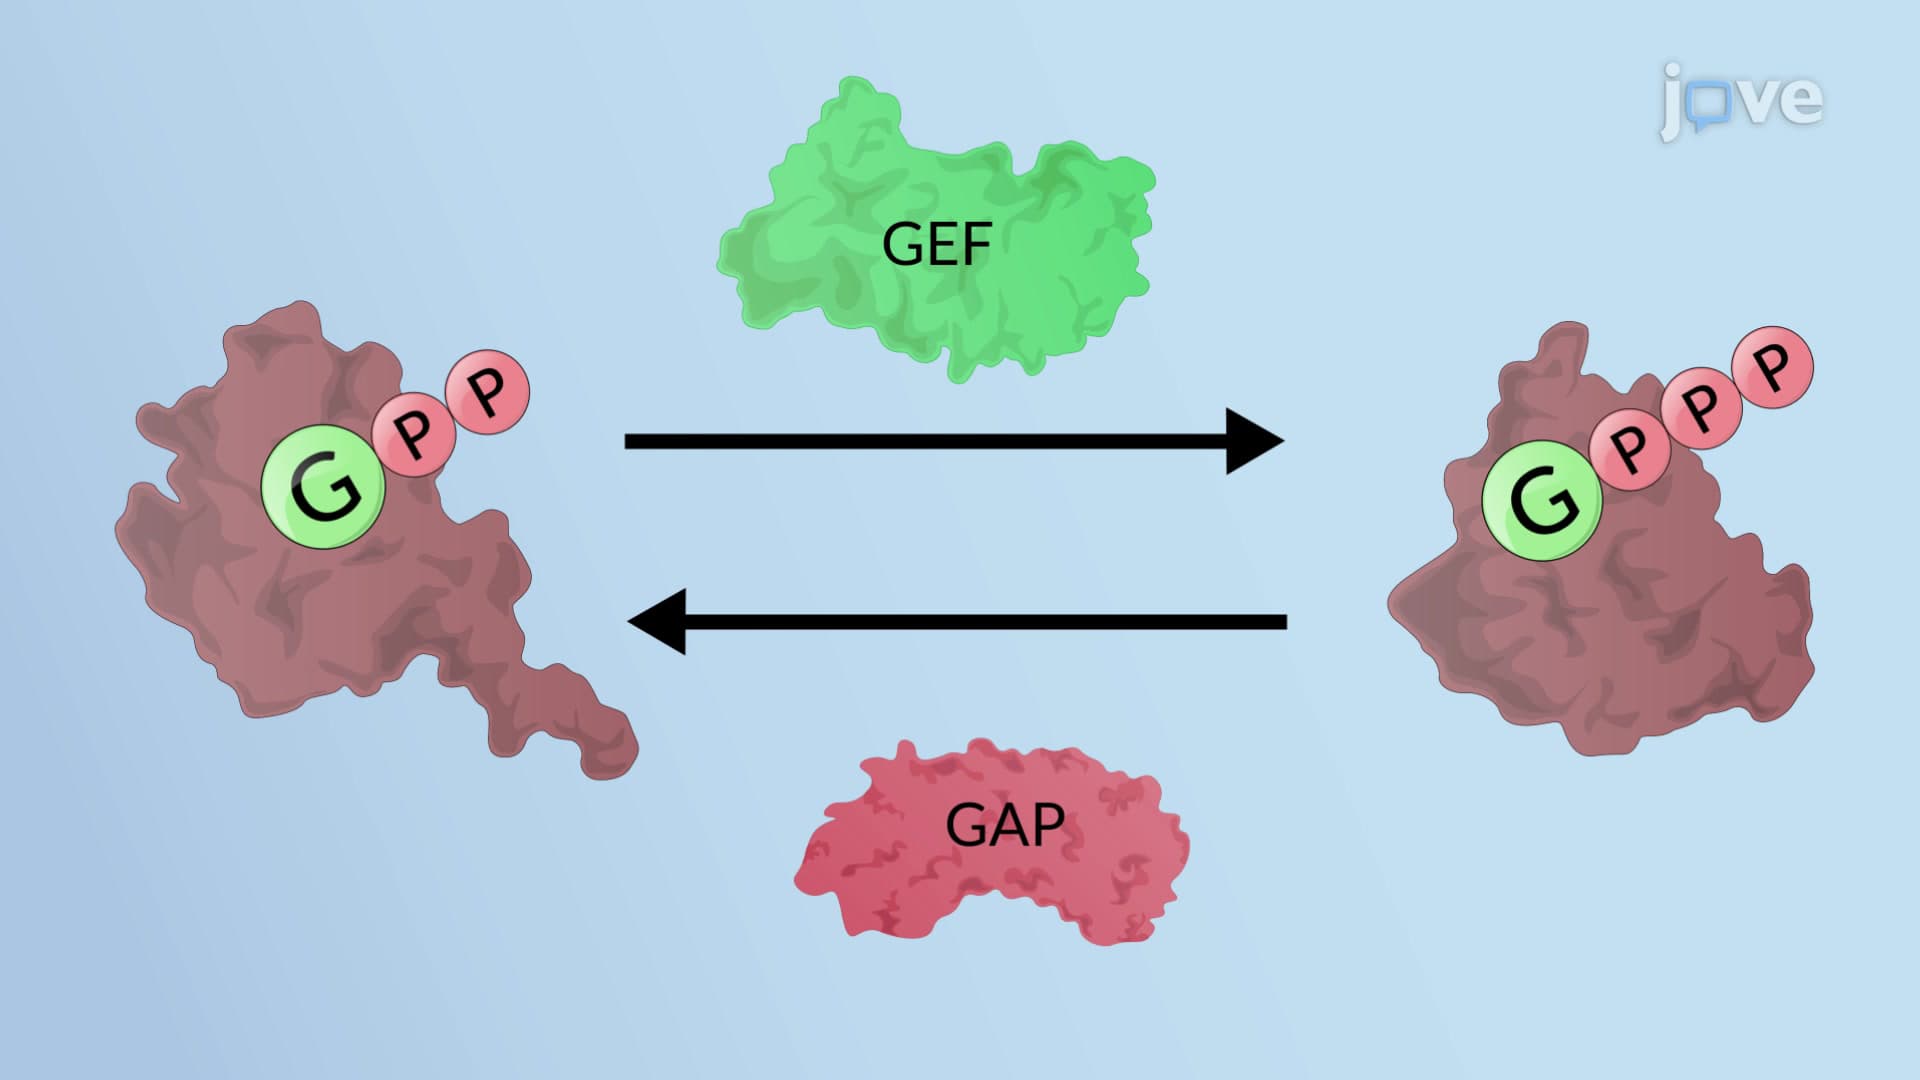
Ras and Rho are small monomeric GTPases that act downstream of receptor tyrosine kinase (RTK) and regulate various cellular processes. These GTPases switch between active and inactive states by binding to guanine nucleotides.
Three regulatory proteins control their activity:
Three regulatory proteins control their activity:
 01:22
Activation and Inactivation of G Proteins
Heterotrimeric G proteins are guanine nucleotide-binding proteins. As the name suggests, heterotrimeric G proteins are composed of three subunits: alpha, beta, and gamma. They remain GDP-bound or GTP-bound inside the cells and switch between inactive/active states. The Gα subunit possesses the nucleotide-binding pocket that binds guanine nucleotides and switches between GDP or GTP-bound states. In contrast, the Gꞵ and Gγ subunits are always bound together with high affinity and are together...
 01:09
GPCRs Regulate Adenylyl Cylase Activity
Some GPCRs transmit signals through adenylyl cyclase (AC), a transmembrane enzyme. AC helps synthesize second messenger cyclic adenosine monophosphate (cAMP). AC catalyzes cyclization reaction and converts ATP to cAMP by releasing a pyrophosphate. The pyrophosphate is further hydrolyzed to phosphate by the enzyme pyrophosphatase, which drives cAMP synthesis to completion. However, cAMP is rapidly degraded to 5′ AMP by the enzymes phosphodiesterase (PDE), preventing overstimulation of cells.
Two...
Two...