凝聚素通过转录,CTCF和Wapl定位在哺乳动物基因组中
Georg A Busslinger1, Roman R Stocsits1, Petra van der Lelij1
1Research Institute of Molecular Pathology (IMP), Vienna Biocenter (VBC), Campus-Vienna-Biocenter 1, A-1030 Vienna, Austria.
Nature
|April 21, 2017

概括
哺乳动物的基因组组织依赖于CCCTC结合因子 (CTCF) 和凝聚素. 这项研究揭示了转录可以转移凝聚素,影响其在CTCF位点的定位和基因调节.
科学领域:
- 基因组学
- 分子生物学
- 表观遗传学
背景情况:
- 哺乳动物的基因组由CTCF和凝聚素组织成染色体循环和拓相关的域.
- CTCF结合点对于凝聚素介导的长距离染色体相互作用至关重要,但凝聚素的招募机制尚不清楚.
研究的目的:
- 研究哺乳动物基因组中的凝聚蛋白分布因素.
- 阐明转录,CTCF和Wapl在凝聚力学和局部化中的作用.
主要方法:
- 使用CTCF枯竭的小鼠纤维细胞观察凝聚性行为.
- 在没有CTCF和Wapl的情况下分析了凝聚蛋白的分布.
- 研究了改变基因表达对凝聚素局部化的影响.
主要成果:
- 凝聚素未能在缺乏CTCF的细胞中进入CTCF位点,而是聚集在活跃的基因转录起点.
- 在没有CTCF和Wapl的情况下,凝聚蛋白在活跃基因的3'-端形成"岛屿",受基因表达水平的影响.
- 在长距离的DNA中观察到转录介导的凝聚素转位,类似于酵母.
结论:
- 转录在哺乳动物凝聚力转移中起着关键作用,有助于其在CTCF位点的定位.
- 活性基因可以通过转录介导转位或Wapl介导释放从凝聚素释放,影响基因调节.
相关概念视频
 02:20
Cohesins
5.8K
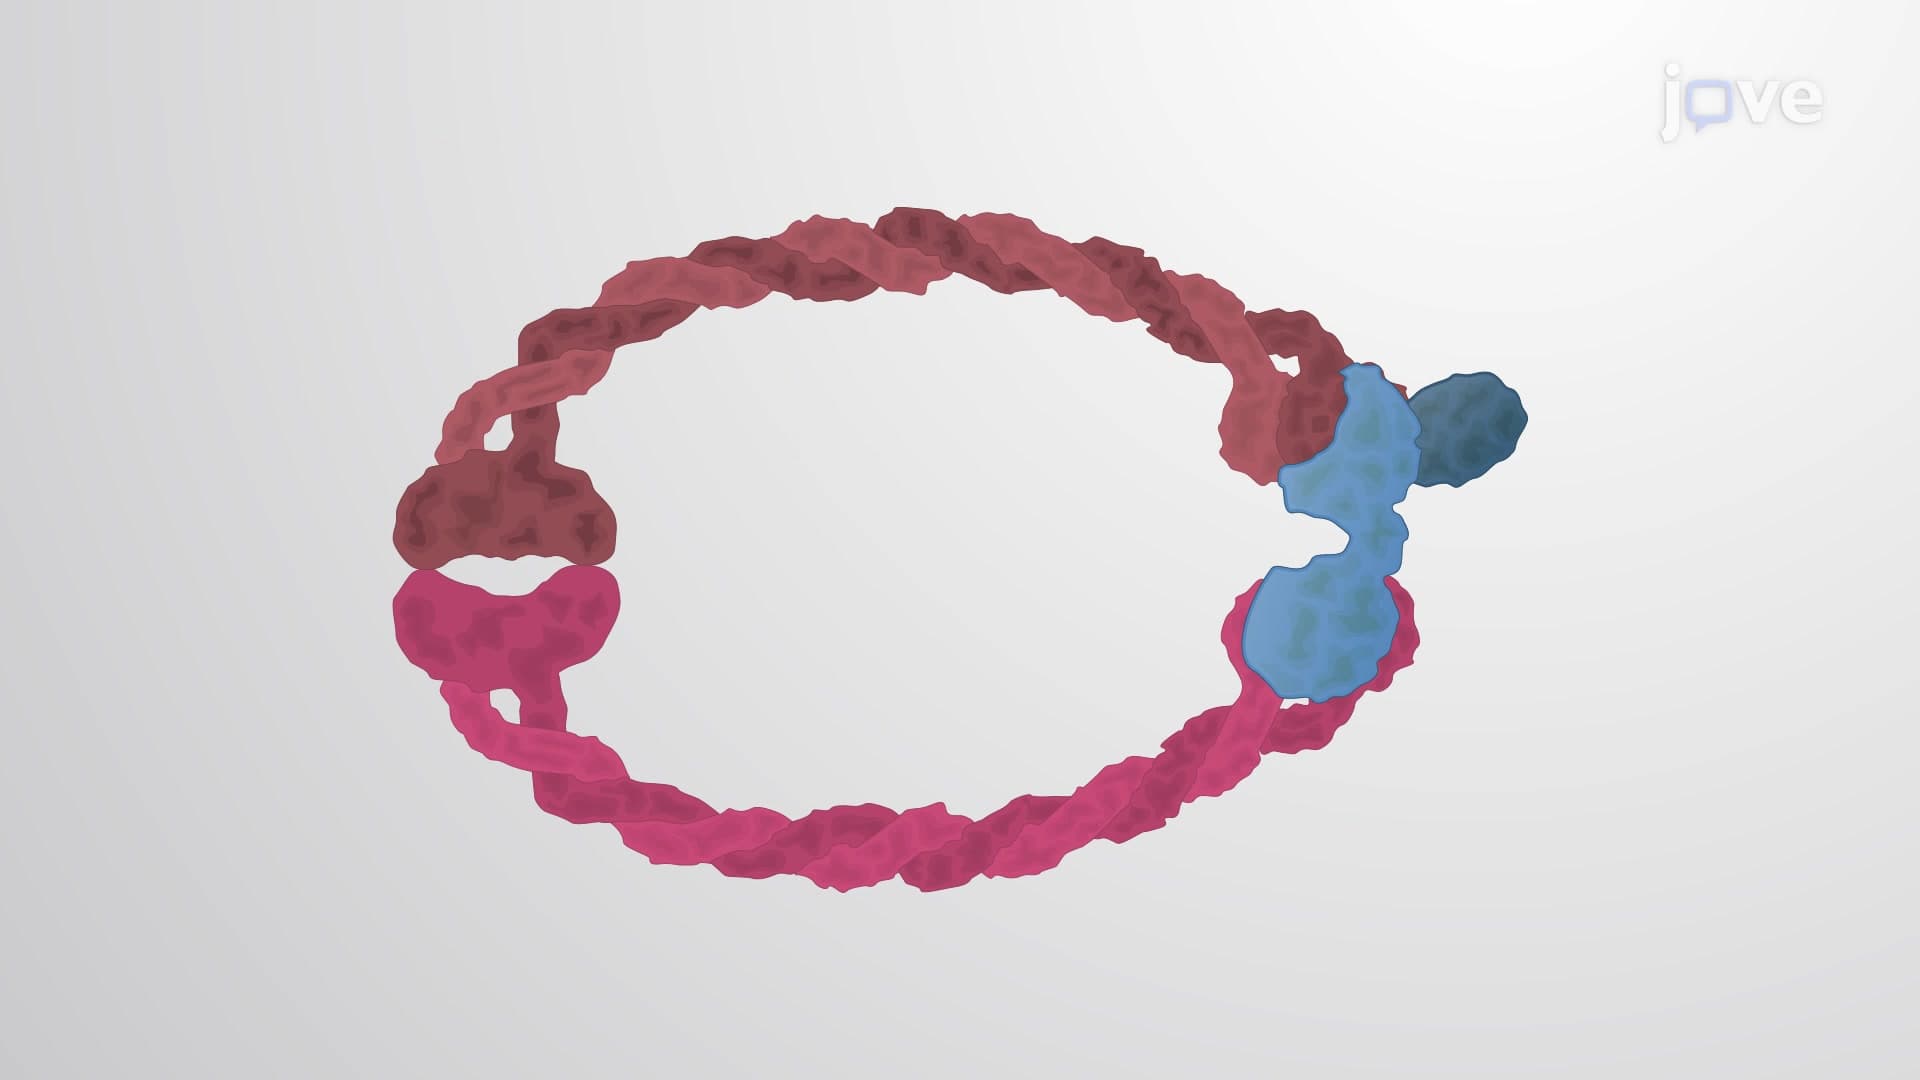
Cohesin protein complexes are a molecular glue that holds two sister chromatids together. They play an important role both in mitosis and meiosis. In mitosis, all cohesin complexes present on the chromosomes are removed before the start of the anaphase stage.
Cohesin complexes in Meiotic Division
Meiosis involves two distinct rounds of chromosomal segregation and cell divisions— Meiosis I followed by Meiosis II – producing four daughter cells. Meiosis I includes the separation of...
Cohesin complexes in Meiotic Division
Meiosis involves two distinct rounds of chromosomal segregation and cell divisions— Meiosis I followed by Meiosis II – producing four daughter cells. Meiosis I includes the separation of...
5.8K
 02:35
Chromatin Position Affects Gene Expression
25.1K
Chromatin is the massive complex of DNA and proteins packaged inside the nucleus. The complexity of chromatin folding and how it is packaged inside the nucleus greatly influences access to genetic information. Generally, the nucleus' periphery is considered transcriptionally repressive, while the cell's interior is considered a transcriptionally active area.
Topologically Associated Domains (TADs)
The 3-dimensional positioning of chromatin in the nucleus influences the...
Topologically Associated Domains (TADs)
The 3-dimensional positioning of chromatin in the nucleus influences the...
25.1K
 02:15
Condensins
4.8K
Condensins are large protein complexes that use ATP to fuel the assembly of chromosomes during mitosis. They transform the tangled, shapeless mass of post-interphase DNA into individualized chromosomes by compacting, organizing, and segregating chromosomal DNA.
The plant and animal cells contain two types of condensin complexes—condensin I and condensin II. Both complexes have five subunits: two SMC (Structural Maintenance of Chromosomes) subunits, a kleisin subunit, and two HEAT-repeat...
The plant and animal cells contain two types of condensin complexes—condensin I and condensin II. Both complexes have five subunits: two SMC (Structural Maintenance of Chromosomes) subunits, a kleisin subunit, and two HEAT-repeat...
4.8K
 02:17
Separation of Sister Chromatids
4.6K
At the transition from prophase to metaphase, there is a reduction in cohesion along the chromosomal arms, resulting in the resolution of sister chromatids. However, residual cohesin connections remain to hold the sister chromatids together until the transition from metaphase to anaphase. The residual connection prevents any premature separation of sister chromatids, blocking the risks of aneuploidy within the daughter cells.
At the onset of anaphase, separase, a proteolytic enzyme, is...
At the onset of anaphase, separase, a proteolytic enzyme, is...
4.6K
 02:30
Histone Variants at the Centromere
5.2K
Histone variants are the histone proteins with structural and sequence variations. These variants may be regarded as “mutant” forms that replace their canonical histone counterparts in the nucleosomes. Specific post-translational modifications on the histone variants enable further chromatin complexity and regulate tissue-specific gene expression. The most common histone variants are from histone H2A, H2B, and linker histone H1 families. However, several variants of histone H3...
5.2K
 02:32
Position-effect Variegation
7.2K
In 1928, a German botanist Emil Heitz observed the moss nuclei with a DNA binding dye. He observed that while some chromatin regions decondense and spread out in the interphase nucleus, others do not. He termed them euchromatin and heterochromatin, respectively. He proposed that the heterochromatin regions reflect a functionally inactive state of the genome. It was later confirmed that heterochromatin is transcriptionally repressed, and euchromatin is transcriptionally active chromatin.
7.2K