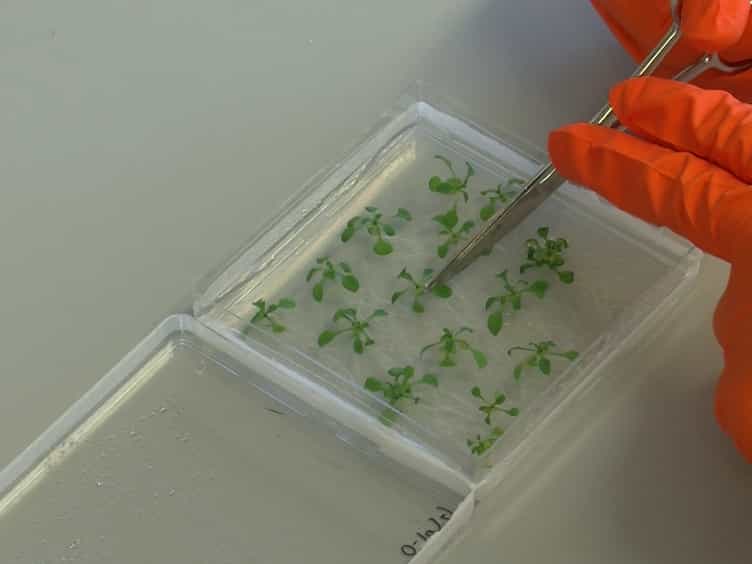

进口蛋白β1调解了EIN2C的核入口,从而赋予了对虫的浮膜防御能力
Kai Lu1, Liyuan Zhang1, Lina Qin1
1State Key Laboratory of Crop Biology, College of Plant Protection, Shandong Agricultural University, Taian 271018, China.
International journal of molecular sciences
|May 27, 2023

概括
乙烯不敏感2 (EIN2) 核贩运,由进口β1 (IMPβ1) 促进,触发了植物对虫的防御. 这种EIN2依赖的基于体的防御抑制了虫的食和Arabidopsis的感染.
科学领域:
- 植物分子生物学 植物分子生物学
- 植物与昆虫的相互作用
- 乙烯信号通路是乙烯信号通路.
背景情况:
- 乙烯不敏感2 (EIN2) 是乙烯信号的关键调节剂,影响植物发育和免疫力.
- EIN2通过释放其碳氧终端部分 (EIN2C) 进行核转位来发挥作用.
- 了解EIN2C的核进口机制对于破译乙烯介导植物反应至关重要.
研究的目的:
- 阐明进口蛋白β1 (IMPβ1) 在EIN2C核贩运中的作用.
- 调查EIN2C核进口,基于花的防御 (PBD) 和Arabidopsis虫的虫耐药性之间的联系.
- 评估EIN2C作为增强对昆虫害虫的植物保护目标的潜力.
主要方法:
- 研究了Arabidopsis中的IMPβ1和EIN2C之间的相互作用.
- 使用乙烯处理和绿色桃花虫感染作为刺激.
- 分析了EIN2C核定位和PBD激活.
- 评估了构成性表达EIN2C对*impβ1*突变物的影响.
主要成果:
- 进口因β1 (IMPβ1) 与EIN2C直接相互作用,通过其核进口进行中介.
- 核贩运EIN2C是由乙烯和绿色桃花虫感染引起的.
- 核进口EIN2C触发了EIN2依赖的基于体的防御反应 (PBD).
- PBD激活有效地阻碍了花的养活动,并减少了虫感染.
- 构成性表达的EIN2C补充了*impβ1*突变体,恢复了核定位和PBD.
结论:
- 进口蛋白β1对于EIN2C核转位至关重要,这是乙烯信号传递中的关键步骤.
- 核进口EIN2C激活了基于花的防御,提供了对虫的抵抗力.
- EIN2C在开发保护农作物免受昆虫伤害的策略方面具有重大潜力.
关键词:
EIN2 C-终端部分 (EIN2C)虫 虫 虫 虫 虫 是 一种阿拉比多普西斯 (Arabidopsis) 是一种植物.进口中的β1 (IMPβ1)核进口是核进口的一个方面.基于体的防御 (PBD)更多相关视频
相关概念视频
 01:25
Cell Signaling in Plants
5.7K
Plant cells communicate to coordinate their cycle of growth, flowering and fruiting, and activities in roots, shoots, and leaves in response to the changing environmental conditions. Plant signaling is distinct from animal signaling. Plants primarily utilize enzyme-linked receptors, whereas the largest class of cell-surface receptors in animals are G-protein coupled receptors (GPCRs). Unlike animals, receptor tyrosine kinases are rare in plants. Instead, plants have a diverse class of...
5.7K
 01:46
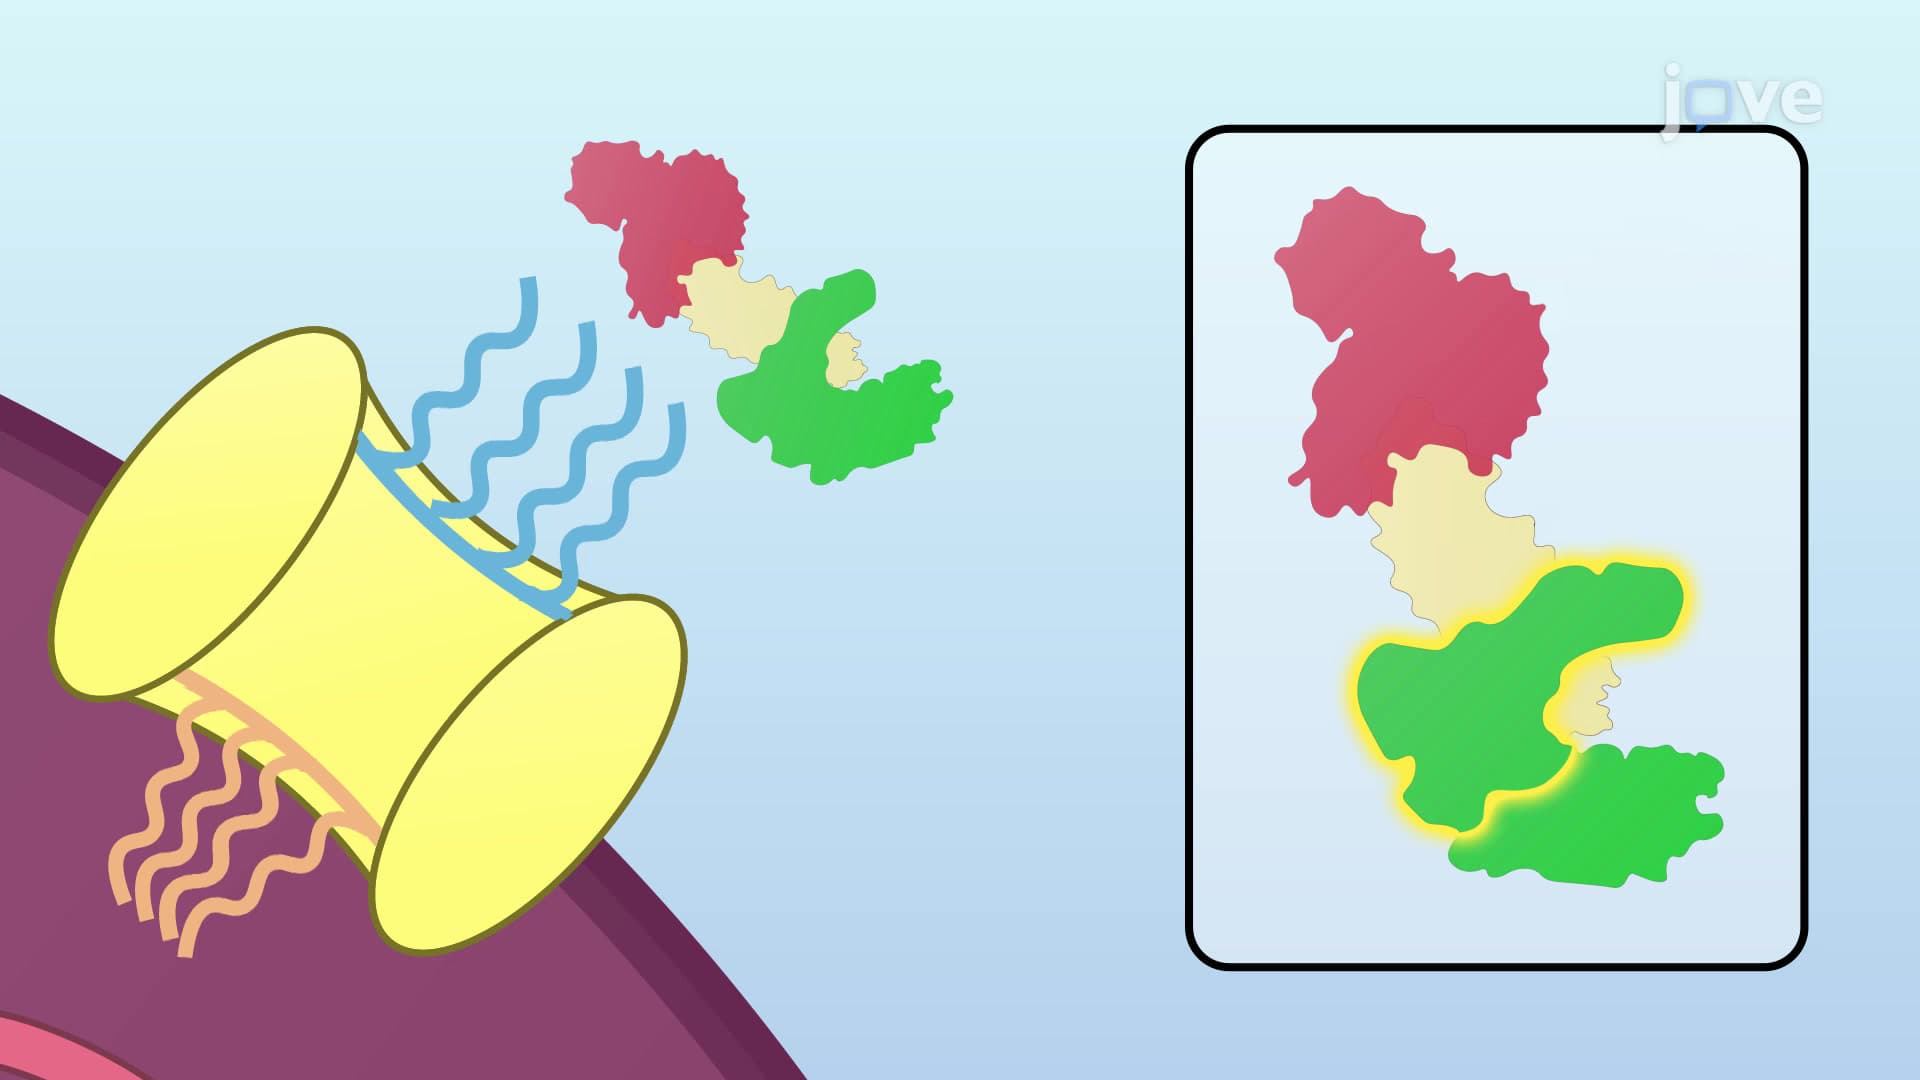
Nuclear Localization Signals and Import
5.8K
Proteins targeted to the nucleus carry short stretches of amino acid sequences called the nuclear localization signal or NLS. Classical nuclear localization signals are of two types: monopartite and bipartite NLS. Monopartite classical NLS (cNLS) consists of a single cluster of 4-8 amino acids. Bipartite cNLS consists of two clusters of 2-3 amino acids and a 9-12 residue long proline-rich linker bridging the two clusters. Signal clusters are rich in positively charged amino acids such as...
5.8K
 02:26
Defenses Against Pathogens and Herbivores
23.9K
Plants present a rich source of nutrients for many organisms, making it a target for herbivores and infectious agents. Plants, though lacking a proper immune system, have developed an array of constitutive and inducible defenses to fend off these attacks.
23.9K
 01:18
Protein Transport to the Inner Chloroplast Membrane
2.1K
Proteins targeted to the inner chloroplast membrane, or plastid proteins, are transported by two general pathways: the stop-transfer and the re-insertion or post-import pathways. Most plastid proteins carry N-terminal transit sequences and internal import sequences targeting it to the specific chloroplast subcompartment. Proteins targeted by the stop-transfer pathway have internal hydrophobic sequences that inhibit their translocation into the stroma. As a result, these precursors are arrested...
2.1K
 01:22
Role of Ephrin-Eph Signalling in Intestinal Stem Cell Renewal
2.3K
Erythropoietin-producing hepatocellular carcinoma receptor (Eph) and its ligand, Eph receptor-interacting protein (Ephrin) were first discovered in the human carcinoma cell line, hence the name. Ephrin-Eph interaction guides cells to reach their appropriate location in adult tissues. They also play an essential role in the immune system by helping in immune cell migration, adhesion, and activation. Based on their structure and function, Eph is divided into two classes — EphA and EphB.
2.3K
 01:11
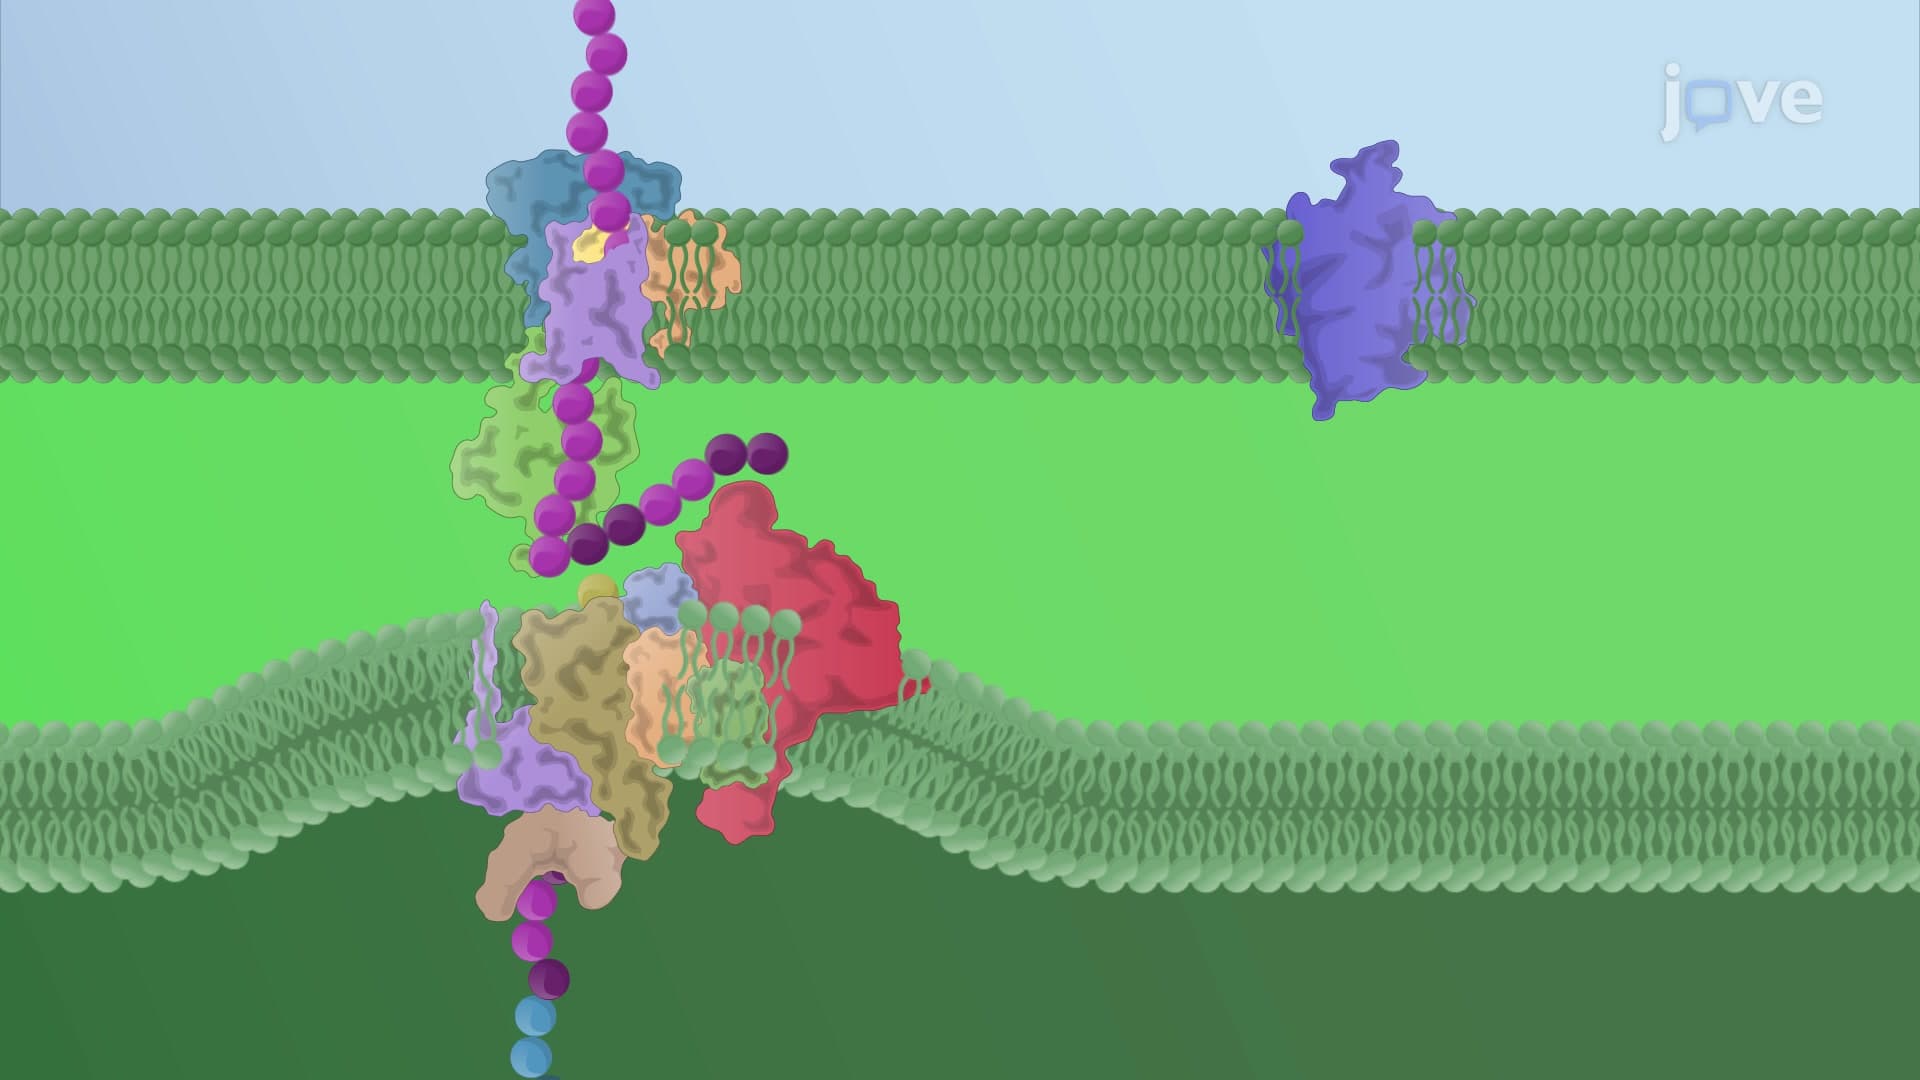
Protein Transport to the Outer Chloroplast Membrane
2.0K
Chloroplast outer membrane proteins encoded by the nucleus are synthesized in the cytosol. Soon after synthesis, they bind cytosolic factors such as 14-3-3 protein and the Hsp70 chaperones that keep these precursors in an unfolded state until their translocation.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
2.0K