相关实验视频
Updated: Jul 27, 2025
09:52
A Fluorescence-based Assay of Phospholipid Scramblase Activity
Published on: September 20, 2016
14.0K
一种脂质杂乱酶TMEM41B参与了GPI定蛋白质的处理和运输
Shu-Ya Cao1, Yi-Shi Liu1, Xiao-Dong Gao1
1Key Laboratory of Carbohydrate Chemistry and Biotechnology, Ministry of Education, School of Biotechnology, Jiangnan University, 1800 Lihu Avenue, Wuxi, Jiangsu 214122, China.
Journal of biochemistry
|June 6, 2023

概括
抑制TMEM41B稳定了PGAP1,增强了ER中的糖酸氨基醇固蛋白 (GPI-AP) 处理. 这与延迟的蛋白质运输一起发生,恢复GPI-APs中的PI-PLC灵敏度.
科学领域:
- 细胞生物学 细胞生物学
- 分子生物学分子生物学
- 蛋白质生物化学 蛋白质生物化学
背景情况:
- 葡萄糖酸氨基醇 (GPI) 定蛋白质 (GPI-APs) 在内质网膜 (ER) 中经历了基本的修改.
- GPI的处理,包括PGAP1的脱基化,决定了GPI-AP的功能和细胞表面的传输.
- 之前的研究将PGAP1活性受损与对酸氨基醇特异性脂酶C (PI-PLC) 的改变的GPI-AP敏感性联系起来.
研究的目的:
- 调查 ER 脂质混杂酶 TMEM41B 在 GPI-AP 处理和贩运中的作用.
- 阐明TMEM41B影响PGAP1活动和GPI-APPI-PLC灵敏性的机制.
主要方法:
- 使用的淘汰细胞模型 (SELT-KO,CLPTM1-KO) 有或没有TMEM41B删除.
- 评估了GPI-APs的PI-PLC敏感性.
- 使用显微镜和生物化学分析分析了从ER到Golgi的蛋白质运输.
- 通过与ER相关的降解途径研究了PGAP1的营业额.
主要成果:
- 丢失TMEM41B恢复了SELT-KO和CLPTM1-KO细胞中GPI-APs的PI-PLC敏感性.
- TMEM41B 缺陷导致了 GPI-AP 和跨膜蛋白从 ER 到 Golgi 的延迟运输.
- TMEM41B淘汰赛减缓了与ER相关的PGAP1降解,导致其稳定.
结论:
- 依赖TMEM41B的脂质杂乱抑制增强了ER中的GPI-AP处理.
- 稳定PGAP1和延迟蛋白贩运是TEMEM41B作用的关键机制.
- 针对TMEM41B提供了一个潜在的策略来调节GPI-AP成熟和细胞表面呈现.
相关概念视频
 01:19
Membrane Asymmetry Regulating Transporters
4.6K
Enzymes like flippase, floppase, and scramblase transfer phospholipids from one layer to another in the membrane, thereby affecting membrane asymmetry.
Flippase
Eukaryotic flippases are type-IV P-type ATPases or P4-ATPases belonging to P-type ATPase family proteins that are membrane-bound pumps involved in the ATP-mediated transport of ions and molecules across the membrane. Flippases flip specific phospholipids from the outer to the inner leaflet of a membrane. All P4-ATPases have one...
4.6K
 01:28
Assembly of the Lipid Bilayer in the ER
3.2K
Biological membranes are more than just a barrier separating cell cytoplasm from the outside environment. They are highly dynamic and help maintain the integrity and physiological stability of the cells as well as membrane-bound organelles. Membranes also play vital roles in cell-to-cell and intracellular communication.
A large chunk of any biological membrane is composed of phospholipids. These lipids have a heterogeneous distribution across different subcellular organelles and even between...
A large chunk of any biological membrane is composed of phospholipids. These lipids have a heterogeneous distribution across different subcellular organelles and even between...
3.2K
 01:29
GPI Anchoring of Proteins in the ER Membrane
4.1K
GPI-anchoring is a post-translational, reversible protein modification that is ubiquitous in eukaryotes. Such proteins are primarily present on the exoplasmic leaflet of the plasma membrane.
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
4.1K
 01:19
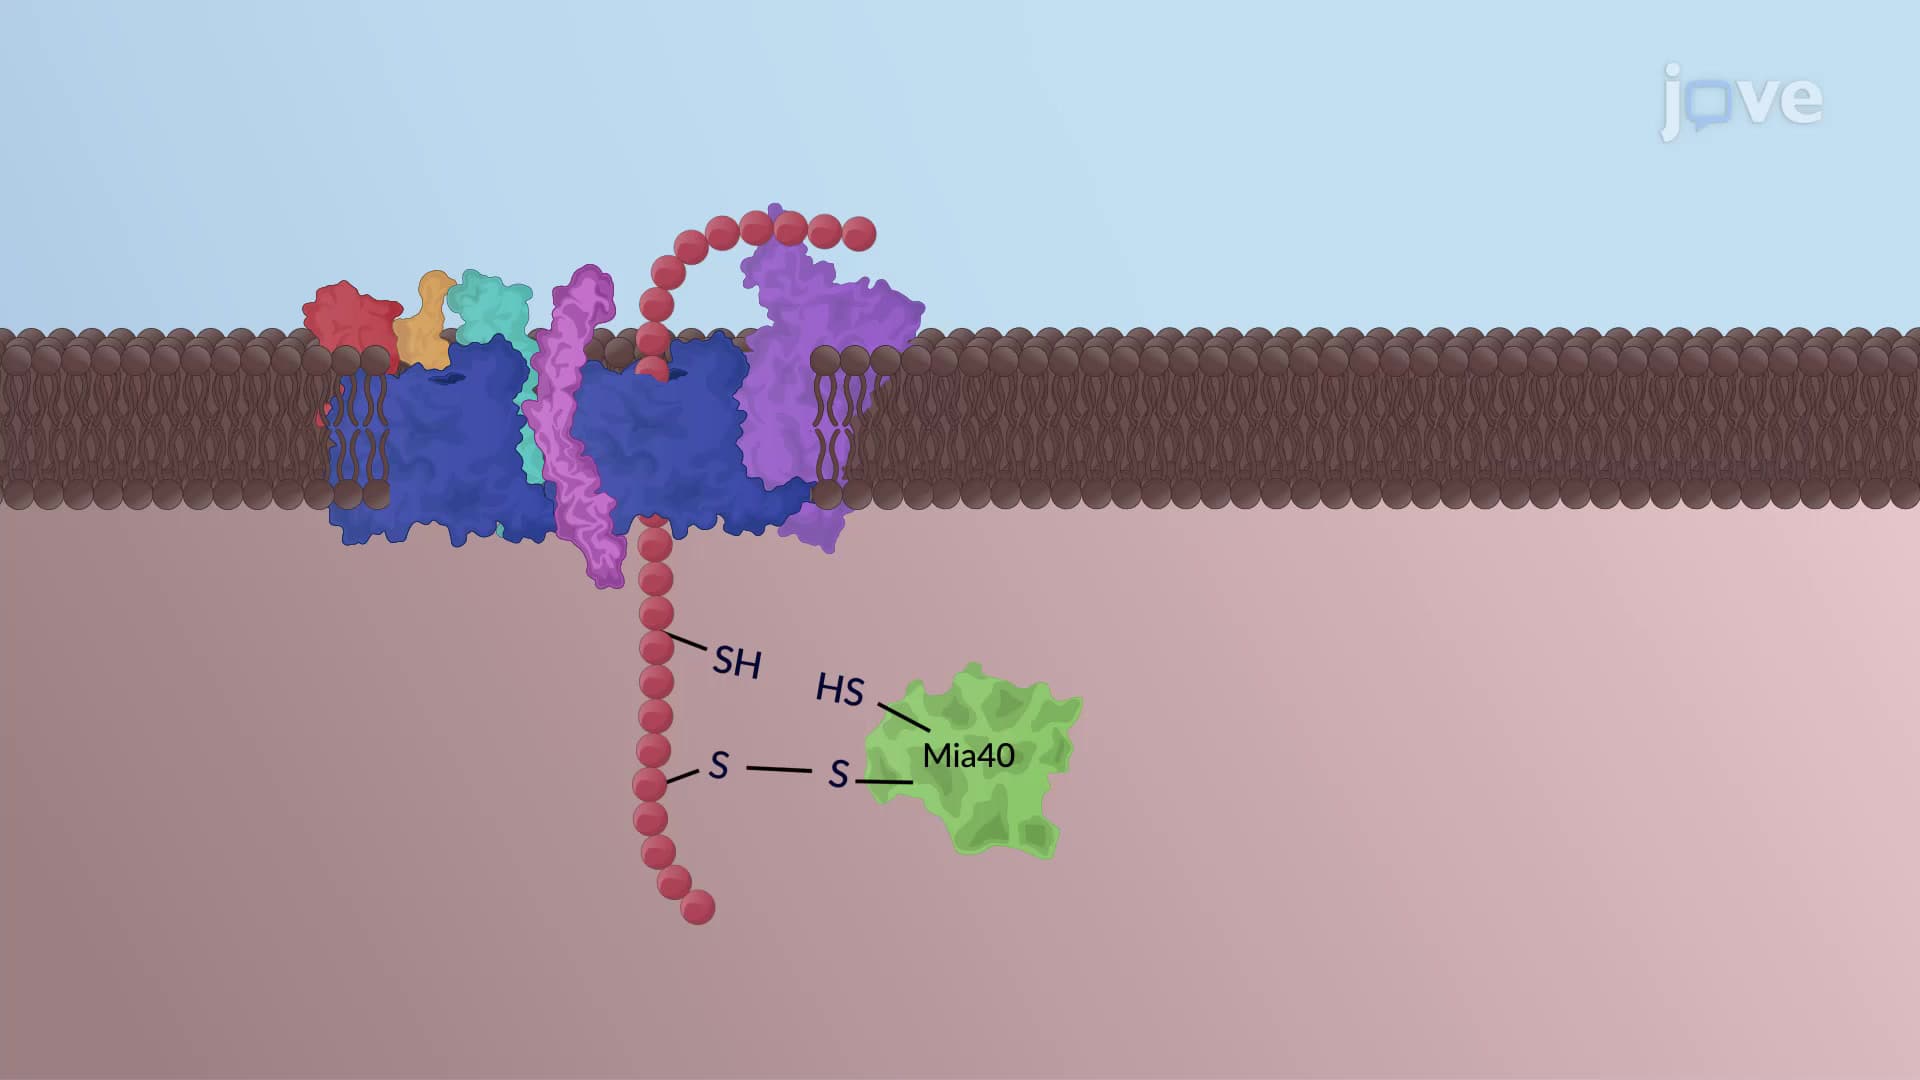
Translocation of Proteins into the Mitochondria
3.2K
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.2K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.1K
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.1K
 01:32
Export of Misfolded Proteins out of the ER
3.7K
After folding, the ER assesses the quality of secretory and membrane proteins. The correctly folded proteins are cleared by the calnexin cycle for transport to their final destination, while misfolded proteins are held back in the ER lumen. The ER chaperones attempt to unfold and refold the misfolded proteins but sometimes fail to achieve the correct native conformation. Such terminally misfolded proteins are then exported to the cytosol by ER-associated degradation or ERAD pathway for...
3.7K