在RTX毒素的乙基化部分中,一个保存的托控制着它们的β2整体素独立的细胞透
Adriana Osickova1, Sarka Knoblochova1, Ladislav Bumba1
1Institute of Microbiology of the Czech Academy of Sciences, Prague, Czech Republic.
The Journal of biological chemistry
|June 30, 2023

概括
像CyaA和HlyA这样的RTX毒素中保存的托芬是透缺乏β2整合素的细胞的关键. 它们的内醇决定了毒素构成,使它们能够独立于整合素结合而进入膜.
科学领域:
- 微生物学和分子生物学
- 蛋白质结构-功能关系 蛋白质结构-功能关系
- 细胞毒理学细胞毒理学
背景情况:
- 重复中毒素 (RTX) 毒素,包括腺酸环酶毒素 (CyaA) 和α-hemolysin (HlyA),与白细胞上的β2整合素结合.
- 这些毒素还可以透到缺乏β2整合素的细胞中,这表明细胞进入的替代机制.
- 在乙化部分内保存的托残留物与毒素活性有关.
研究的目的:
- 为了研究保留的型英醇 (CyaA中的W876,HlyA中的W579) 在β2整合素独立膜透中的作用.
- 阐明这些托残留物对RTX毒素活性的结构和功能影响.
主要方法:
- 保存的托残留物 (CyaA中的W876,HlyA中的W579) 的局部定向突变生成到各种氨基酸.
- 对具有和没有β2整蛋白表达的细胞的毒素活性和细胞毒性的评估.
- 热稳定性测试 (Tm) 和-交换质谱 (HDX-MS) 来探测结构变化.
主要成果:
- W876 (CyaA) 和W579 (HlyA) 的突变损害了β2整合素独立的膜透,同时节省了整合素依赖的活性.
- 这些替代物增加了CyaA的热稳定性,并改变了局部疏水性段的可访问性.
- 在W876中罗利丁-英多尔相互作用的破坏也选择性地损害了红细胞上的CyaA活性.
结论:
- 庞大的W876 (CyaA) 和W579 (HlyA) 的内醇对RTX毒素透至关重要,独立于β2整合素结合.
- 这些残留物调节了乙化环的定位,促进了穿透膜的形状.
- 这些发现揭示了RTX毒素进入细胞的新机制,突出了保存的型的结构性作用.
相关概念视频
 01:17
Intracellular Signaling Affects Focal Adhesions
2.7K
Integrins act both as extracellular input receivers and as intracellular processing activators. As their name suggests, integrins are entirely integrated into the membrane structure. Their hydrophobic membrane-spanning regions interact with the phospholipid bilayer's hydrophobic region. These membrane receptors provide extracellular attachment sites for effectors like hormones and growth factors. They activate intracellular response cascades when their effectors are bound and active.
Some...
Some...
2.7K
 01:15
Activation of Integrins
3.5K
Integrins bind ligands and transmit information from outside the cell to inside or vice-versa through an "outside-in signaling" or "inside-out signaling."
In "outside-in signaling," external factors in the extracellular space bind to exposed ligand binding sites on integrins. This causes the inactive protein to undergo a conformational change to become active. Integrins are often clustered on the cell membrane. Repetitive and regularly spaced ligand binding...
In "outside-in signaling," external factors in the extracellular space bind to exposed ligand binding sites on integrins. This causes the inactive protein to undergo a conformational change to become active. Integrins are often clustered on the cell membrane. Repetitive and regularly spaced ligand binding...
3.5K
 01:19
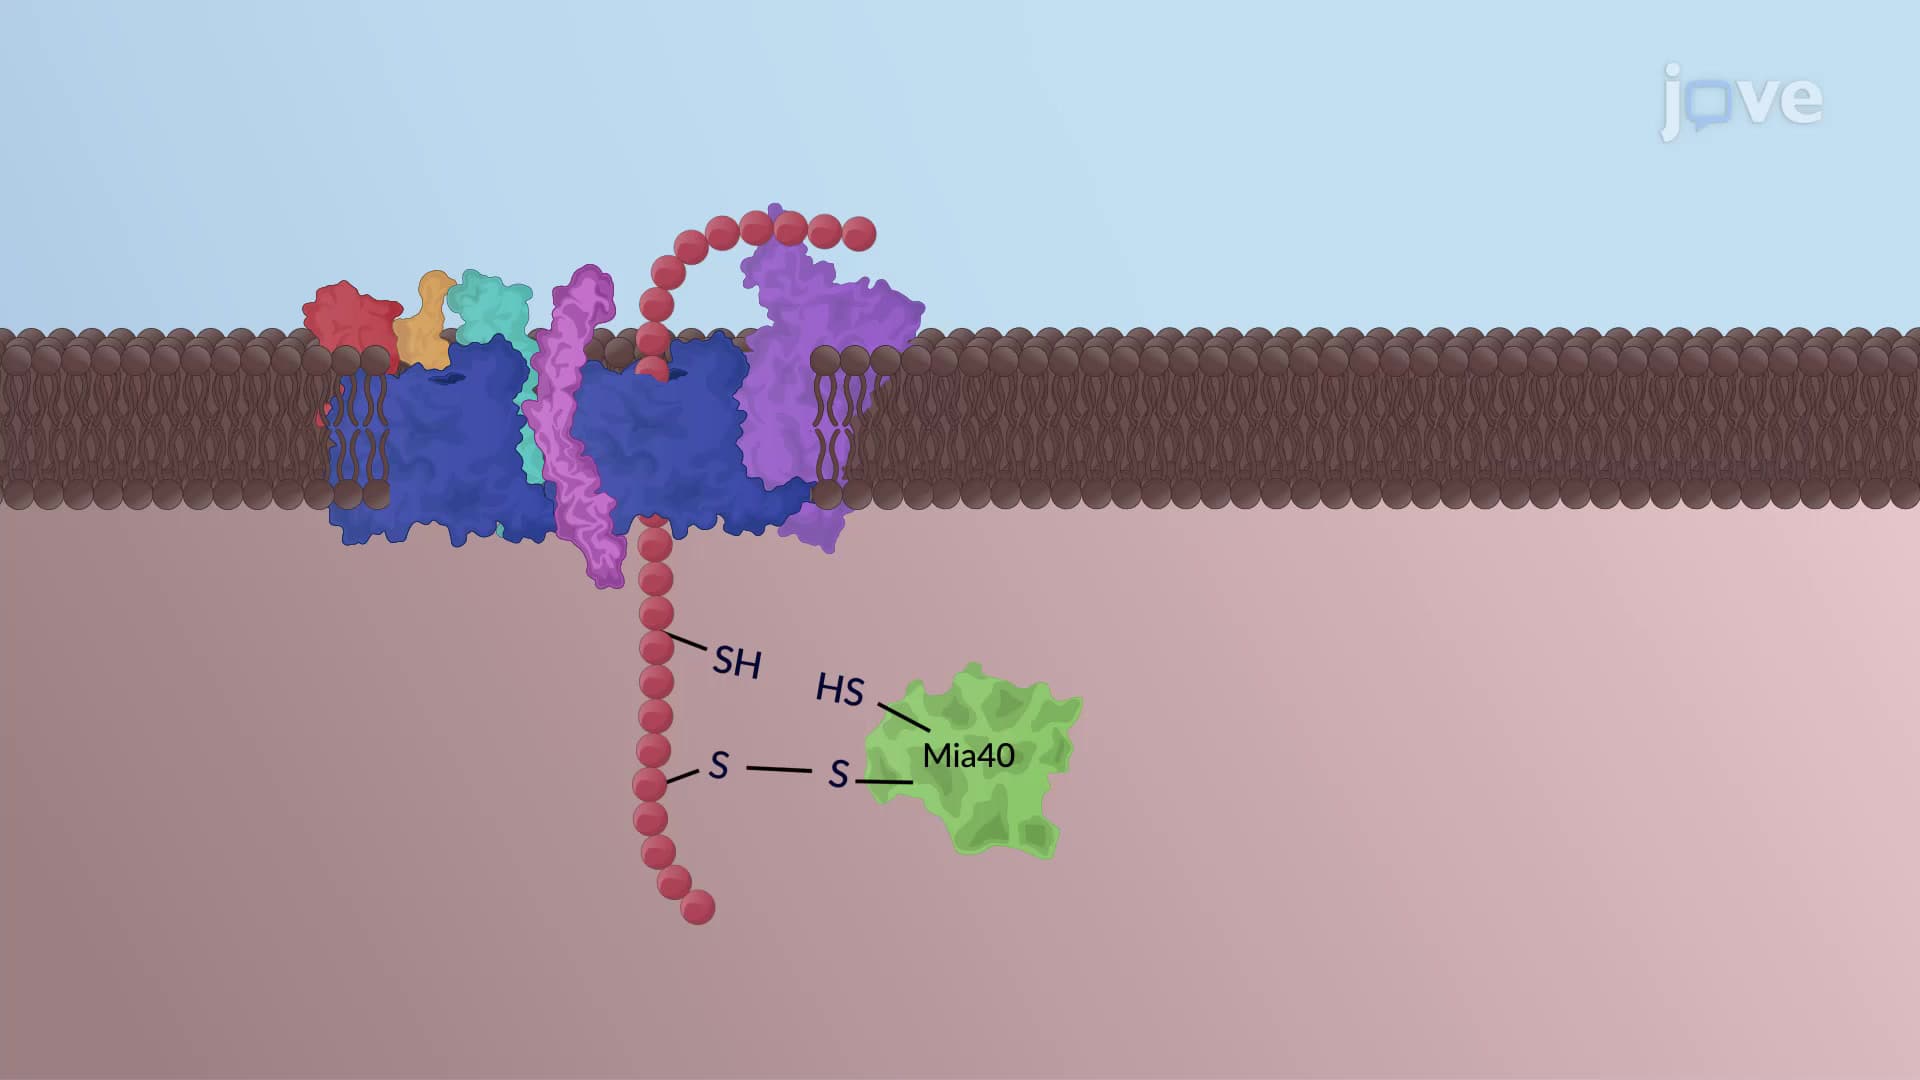
Translocation of Proteins into the Mitochondria
3.2K
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.2K
 01:10
Integrins
4.0K
Animal and protozoan cells do not have cell walls to help maintain shape and provide structural stability. Instead, these eukaryotic cells secrete a sticky mass of carbohydrates and proteins into the spaces between adjacent cells. This network of proteins and molecules is called an extracellular matrix or ECM.
Some ECM proteins assemble into a basement membrane to which the remaining components adhere. Proteoglycans typically form the bulk of the ECM while fibrous proteins, like collagen,...
Some ECM proteins assemble into a basement membrane to which the remaining components adhere. Proteoglycans typically form the bulk of the ECM while fibrous proteins, like collagen,...
4.0K
 01:34
Protein Transport into the Inner Mitochondrial Membrane
3.8K
Nuclear encoded mitochondrial precursors are imported to the inner membrane in a multistep process involving two separate translocons, TIM22 and TIM23. TIM23 is a cation-selective pore that remains closed by the N terminal segment of the protein. Negative charges on the TIM23 act as a receptor for the incoming precursor, pulling the positively charged matrix-targeting sequence for peptide insertion and translocation.
Transport of mitochondrial precursors across the TIM23 channel is driven by...
Transport of mitochondrial precursors across the TIM23 channel is driven by...
3.8K
 01:20
Cotranslational Protein Translocation
7.4K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
7.4K