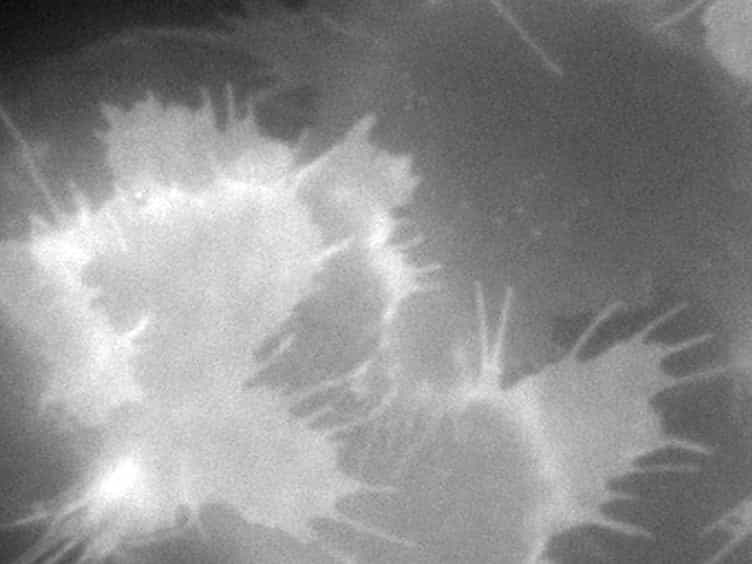
CIP4的自我组装驱动了在克拉特林介导的内细胞分裂中,以行为因子为媒介的不对称的坑关闭
Yiming Yu1, Shige H Yoshimura2
1Graduate School of Biostudies, Kyoto University, Kyoto, 606-8501, Japan.
Nature communications
|August 1, 2023

概括
克拉特林介导的内细胞分裂涉及不对称的坑关闭,由蛋白质CIP4驱动. 这种蛋白质的蛋白质.
科学领域:
- 细胞生物学 细胞生物学
- 生物物理学的生物物理.
- 细胞内核的分子机制 细胞内核的分子机制
背景情况:
- 克拉特林介导的内细胞分裂 (CME) 对于细胞通信至关重要.
- 在克拉特林涂层坑附近的不对称的行为分布表明CME期间的非辐射收缩.
- 这种不对称的CME的分子基础仍然不清楚.
研究的目的:
- 阐明CME中不对称的坑关闭背后的分子机制.
- 为了研究蛋白质CIP4在调节细胞内核分裂期间的actin动态中的作用.
主要方法:
- 使用了高速原子力显微镜 (HS-AFM).
- 对多域蛋白CIP4的分析,包括其F-BAR域和内在无序区域.
- 研究了CIP4,膜曲率和活性蛋白调节蛋白之间的相互作用.
主要成果:
- 在CME中,CIP4对于不对称的坑关闭机制至关重要.
- 通过内在无序区域的CIP4自我组装驱动了局部化的actin聚合.
- CIP4确定了与曲膜和活性调节剂的立体特异性相互作用.
结论:
- 结构化和无序域之间的CIP4的协作是时空actin聚合的关键.
- 这种机制解释了在克拉斯林介导的内细胞分裂过程中如何发生不对称的坑关闭.
- 提供了通过蛋白质-actin相互作用调节膜动态的机制性见解.
相关概念视频
 01:39
Mechanism of Filopodia Formation
2.4K
Filopodia are thin, actin-rich cellular protrusions that play an important role in many fundamental cellular functions. They vary in their occurrence, length, and positioning in different cell types, suggesting their diverse roles.
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
2.4K
 01:12
Clathrin Coated Vesicles
7.1K
Clathrin-coated vesicles use endocytosis to transport receptors and lysosomal hydrolases from the Golgi to the lysosome in the late secretory pathway. Clathrin-mediated endocytosis was the first described endocytic process, and Clathrin-coated vesicles remain one of the most well-studied transport vesicles. The molecular machinery that generates clathrin-coated vesicles comprises over 50 proteins that precisely coordinate vesicle formation. Cell surface receptors concentrated in indented sites...
7.1K
 01:32
Pinching-off of Coated Vesicles
3.2K
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
3.2K
 01:31
Mechanism of Lamellipodia Formation
2.6K
Cells migrating in response to external stimuli form lamellipodia, which are thin membrane protrusions supported by a mesh of linked, branched, or unbranched actin filaments. These actin filaments interact with myosin motor proteins, creating the dynamic actomyosin complex within the cytoskeleton. Contractility, or the ability to generate contractile stress, is inherent to the actomyosin complex. It helps cells detect the stiffness of the surrounding ECM and exert contractile force for...
2.6K
 01:33
Coat Assembly and GTPases
3.6K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.6K
 01:14
Generation of Straight or Branched Actin Filaments
2.9K
The straight or branched structure formation of actin filaments is controlled by nucleating proteins such as the formins and Arp2/3 complex. Formin-mediated assembly results in straight filaments, whereas Arp2/3 protein complex-mediated assembly results in branched actin filaments.
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
2.9K