
铁素调节了人体tRNA结合酶复合物的氧化还原状态和活性
Dhaarsini Jaksch1,2, Johanna Irnstorfer1, Petra-Franziska Kalman1
1Max Perutz Laboratories, Medical University of Vienna, Vienna Biocenter (VBC), 1030 Vienna, Austria.
RNA (New York, N.Y.)
|August 30, 2023

概括
铁素 (TRX) 通过减少氧化RTCB. 修复tRNA结合酶复合体 (tRNA-LC) 的活性位点. 这确保了在氧化应激下的tRNA前拼接和未折叠蛋白质响应 (UPR) 功能.
科学领域:
- 分子生物学分子生物学
- 细胞生物学 细胞生物学
- 生物化学 生物化学
背景情况:
- tRNA结合酶复合体 (tRNA-LC) 在未折叠蛋白质反应 (UPR) 期间对tRNA前拼接和XBP1mRNA拼接至关重要.
- 作为tRNA-LC的催化子单元的RTCB,需要对氧化损伤进行保护,正如之前PYROXD1.1所示的那样.
研究的目的:
- 调查雷素 (TRX) 在维持RTCB的酶活性中的作用.
- 了解UPR和氧化条件期间TRX和RTCB之间的相互作用.
主要方法:
- 在体外测试以评估RTCB活性和与TRX的相互作用.
- 在UPR的晚期阶段对TRX-RTCB相互作用的分析.
- 研究RTCB的氧化还原状态和TRX的影响.
主要成果:
- 铁素 (TRX) 保持了RTCB对氧化剂的酶活性.
- TRX与氧化RTCB物理相互作用,并通过其氧化还原活性氨酸对重新激活它.
- 在晚期的UPR期间,TRX与RTCB相互作用,这表明长期的UPR会产生活性氧物种.
结论:
- TRX在确保和修复tRNA-LC的活性位点方面发挥着至关重要的作用.
- 这种TRX的功能使得tRNA前拼接和UPR在温和,抑制性氧化应激水平下进行.
相关概念视频
 01:41
The Supercomplexes in the Crista Membrane
2.5K
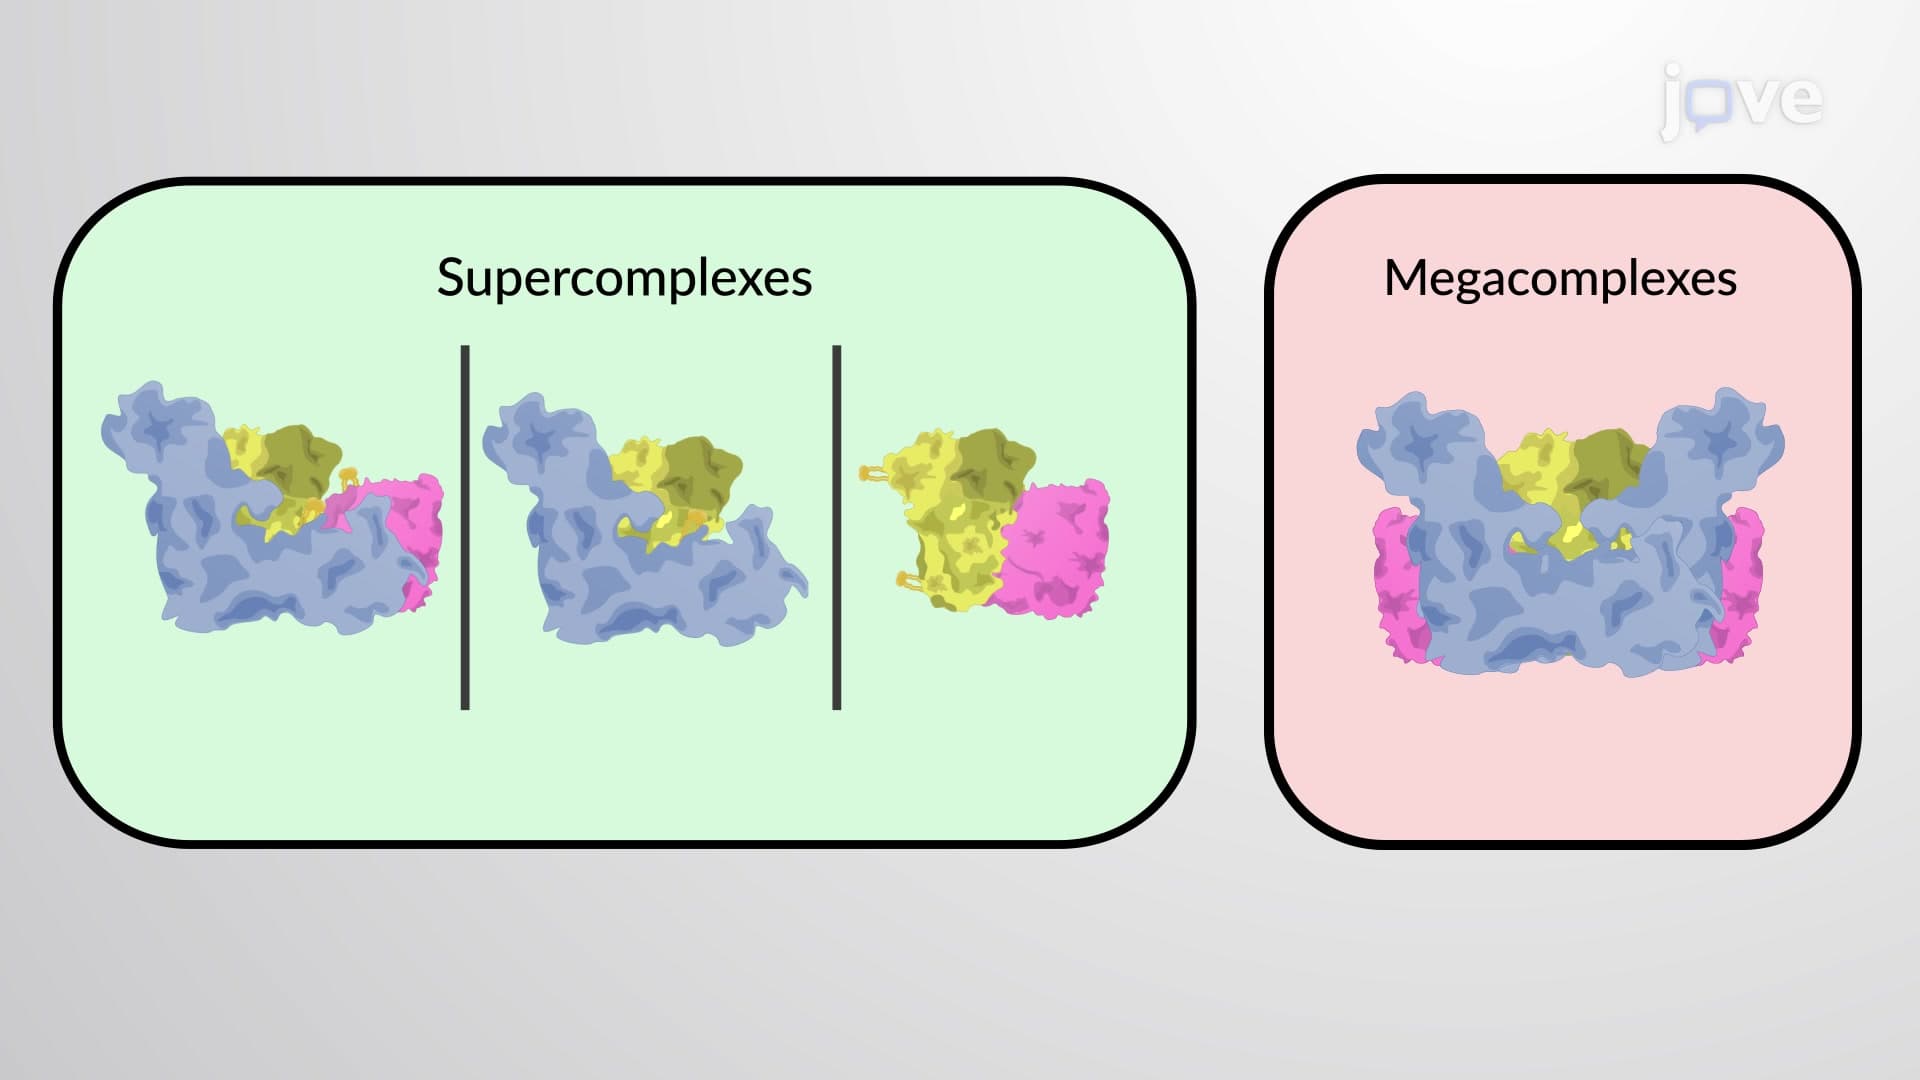
The mitochondrial cristae membrane is the primary site for the oxidative phosphorylation (OXPHOS) process of energy conversion mediated through respiratory complexes I to V. These complexes have been widely studied for decades, and it has been proven that they form supramolecular structures called respiratory supercomplexes (SC). These higher-order complexes may be crucial in maintaining the biochemical structure and improving the physiological activity of the individual complexes while...
2.5K
 01:30
The Electron Transport Chain
16.9K
The electron transport chain or oxidative phosphorylation is an exothermic process in which free energy released during electron transfer reactions is coupled to ATP synthesis. This process is a significant source of energy in aerobic cells, and therefore inhibitors of the electron transport chain can be detrimental to the cell's metabolic processes.
Inhibitors of the electron transport chain
Rotenone, a widely used pesticide, prevents electron transfer from Fe-S cluster to ubiquinone or Q...
Inhibitors of the electron transport chain
Rotenone, a widely used pesticide, prevents electron transfer from Fe-S cluster to ubiquinone or Q...
16.9K
 01:43
Electron Transport Chain: Complex III and IV
7.6K
During the electron transport chain, electrons from NADH and FADH2 are first transferred to complexes I and II, respectively. These two complexes then transfer the electrons to ubiquinol, which carries them further to complex III. Complex III passes the electrons across the intermembrane space to Cyt c, which carries them further to complex IV. Complex IV donates electrons to oxygen and reduces it to water. As electrons pass through complexes I, III, and IV, the energy released aids the pumping...
7.6K
 02:26
tRNA Activation
19.3K
Aminoacyl-tRNA synthetases are present in both eukaryotes and bacteria. Though eukaryotes have 20 different aminoacyl-tRNA synthetases to couple to 20 amino acids, many bacteria do not have genes for all of these aminoacyl-tRNA synthetases. Despite this, they still use all 20 amino acids to synthesize their proteins. For instance, some bacteria do not have the gene encoding the enzyme that couples glutamine with its partner tRNA. In these organisms, one enzyme adds glutamic acid to all of the...
19.3K
 02:36
Transfer RNA Synthesis
12.0K
One of the unique features of tRNA is the presence of modified bases. In some tRNAs, modified bases account for nearly 20% of the total bases in the molecule. Altogether, these unusual bases protect the tRNA from enzymatic degradation by RNases.
Each of these chemical modifications is carried by a specific enzyme, post-transcription. All of these enzymes have unique base and site-specificity. Methylation, the most common chemical modification, is carried by at least nine different enzymes, with...
Each of these chemical modifications is carried by a specific enzyme, post-transcription. All of these enzymes have unique base and site-specificity. Methylation, the most common chemical modification, is carried by at least nine different enzymes, with...
12.0K
 01:31
Regulation of the Unfolded Protein Response
2.5K
Inositol-requiring kinase one or IRE1 is the most conserved eukaryotic unfolded protein response (UPR) receptor. It is a type I transmembrane protein kinase receptor with a distinctive site-specific RNase activity. As the binding mechanics of the misfolded proteins with the N-terminal domain of IRE-1 are unclear, three binding models — direct, indirect, and allosteric -- are proposed for receptor activation. Nevertheless, it is known that once a misfolded protein associates with IRE1, it...
2.5K