
需要对Atg16进行卷轴-卷轴介导的二分化,以便与PROPPIN Atg21结合
Miranda Bueno-Arribas1, Celia Cruz-Cuevas1, María-Angeles Navas2
1Instituto de Investigaciones Biomédicas Sols-Morreale CSIC-UAM, Madrid, 28029, Spain.
Open biology
|November 21, 2023

概括
酵母Atg21和哺乳动物WIPI2蛋白与Atg16/ATG16L1结合,这对自细胞形成至关重要. 这项研究使用RD2H系统确定了Atg21和Atg16中的关键残留物,这些残留物对于这种相互作用至关重要.
科学领域:
- 细胞生物学 细胞生物学
- 分子生物学分子生物学
- 生物化学 生物化学
背景情况:
- PROPPINs/WIPIs是参与膜重塑的β-螺旋蛋白,包括自细胞形成和内贩运.
- 酵母Atg21和哺乳动物WIPI2与Atg16/ATG16L1相互作用,将脂化机制招募到自细胞膜中.
研究的目的:
- 用反向双双混合 (RD2H) 方法识别Atg21和Atg16中关键残留物,这些残留物对于它们的蛋白质-蛋白质结合至关重要.
- 为了研究Atg16卷轴-卷轴域二元化在Atg21结合中的作用.
- 评估WIPI2中确定的残留物的保存情况及其在ATG16L1结合中的作用.
主要方法:
- 反向双双混合 (RD2H) 系统用于识别蛋白质-蛋白质相互作用的关键残留物.
- 蛋白质复杂晶体结构的分析.
- 局部定向突变发生,以产生组合突变.
主要成果:
- 对于Atg21结合,Atg16卷-卷域的二元化是必要的.
- 确定了Atg21中调节ATG16L1结合的保存残留物,与其他自蛋白相互作用中的残留物占有类似的结构位置.
- 证明了RD2H系统在识别相互作用热点和产生完全失去结合的突变物的有效性.
结论:
- RD2H系统是剖析蛋白质与蛋白质相互作用的强大工具.
- 在Atg21和WIPI2中的特定残留物对于结合Atg16/ATG16L1至关重要,突出显示了自过程中保留的相互作用机制.
- 结构性见解表明,自机械内部的蛋白质-蛋白质相互作用接口的融合进化.
相关概念视频
 01:33
Coat Assembly and GTPases
3.5K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.5K
 01:39
Mechanism of Filopodia Formation
2.4K
Filopodia are thin, actin-rich cellular protrusions that play an important role in many fundamental cellular functions. They vary in their occurrence, length, and positioning in different cell types, suggesting their diverse roles.
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
2.4K
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.3K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.3K
 01:42
Actin Polymerization
6.6K
Actin polymerization occurs through the head-to-tail association of binding sites on monomeric actin or G-actin to form filamentous or F-actin. The polymerization can be divided into three phases ̶ nucleation, elongation, and steady-state phase.
The nucleation phase involves forming a stable nucleus consisting of three actin monomers to form a new actin filament. Actin-binding proteins such as formins and Arp2/3 complex help filament growth post-nucleation. The Formins form straight...
The nucleation phase involves forming a stable nucleus consisting of three actin monomers to form a new actin filament. Actin-binding proteins such as formins and Arp2/3 complex help filament growth post-nucleation. The Formins form straight...
6.6K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.1K
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.1K
 01:19
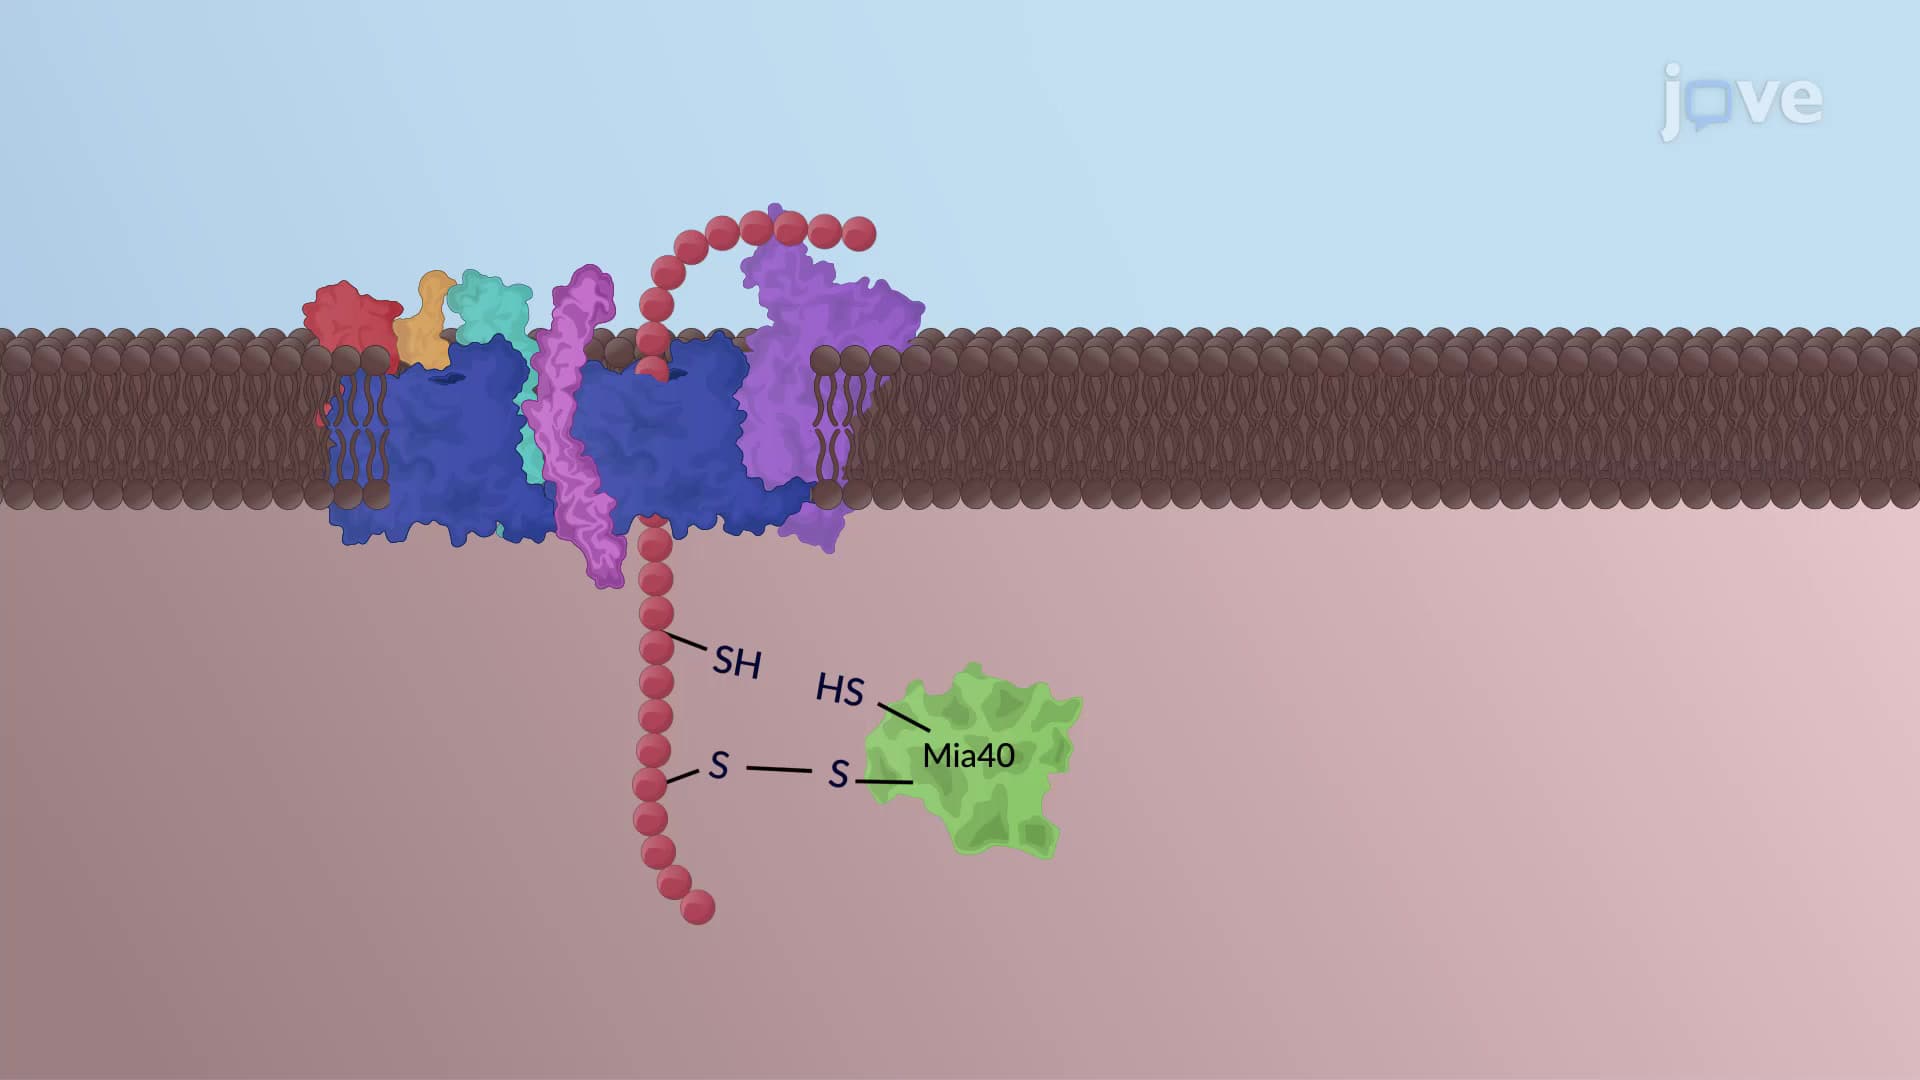
Translocation of Proteins into the Mitochondria
3.1K
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.1K