
ZYG-1的特定位点酸化调节ZYG-1的稳定性和中心细胞数量
Jeffrey C Medley1, Rachel N Yim1, Joseph DiPanni1
1Department of Biological Sciences, Oakland University, Rochester, MI, USA.
iScience
|November 30, 2023

概括
kazein kinase II (CK2) 通过调节 ZYG-1 蛋白质水平来控制中心体重复. CK2化向ZYG-1进行降解,防止过度的中枢细胞组合并保持基因组的稳定性.
科学领域:
- 细胞生物学 细胞生物学
- 分子遗传学 分子遗传学
- 基因组完整性 基因组完整性
背景情况:
- 螺旋双极性对于准确的细胞分裂和基因组完整性至关重要.
- 中心体数是轴心双极性的关键决定因素,需要严格监管中心体组合.
- 在这个过程中,ZYG-1 (中心细胞复制的主调节器) 是核心的.
研究的目的:
- 研究素激酶II (CK2) 在调节ZYG-1中的作用.
- 阐明CK2介导的ZYG-1调控对中枢细胞组合和重复的影响.
主要方法:
- 试验室内激酶试验以评估ZYG-1的CK2酸化.
- 在体内共免疫沉以确认ZYG-1和CK2相互作用.
- 通过RNA干扰 (RNAi) 来消耗CK2.
- 对野生型和突变的C. elegans菌株中中心细胞数的分析.
- 局部定向突变生成以产生非酸化的ZYG-1突变体.
- 蛋白质酶抑制研究.
主要成果:
- 在体外,CK2直接化ZYG-1,并在体内与ZYG-1相互作用.
- CK2的耗尽或ZYG-1酸化位点的破坏会导致中枢细胞体放大.
- 非酸化的ZYG-1突变体显示ZYG-1水平增加和中心体相关的ZYG-1水平升高.
- 抑制26S蛋白酶体阻断了相仿ZYG-1的降解.
结论:
- CK2-依赖ZYG-1的酸化是控制ZYG-1蛋白水平的关键机制.
- 这种酸化事件针对ZYG-1进行蛋白质体降解,从而限制中心体数量.
- 这种途径的调节失调可能导致中枢细胞体放大和潜在的基因组不稳定性.
相关概念视频
 00:50
Anaphase Promoting Complex
2.9K
The stepwise destruction of specific proteins is necessary for the progression and completion of the cell cycle. Such proteins are ubiquitinated by ubiquitin ligases and then subsequently destroyed by the proteasome. The SCF (Skp1/Cullin/F-box) and the anaphase-promoting complex (APC) are two important ubiquitin ligases involved in cell cycle progression. While SCF is active throughout the cell cycle, APC gets activated during metaphase to anaphase transition. Cdc20 or Cdh1 binds to APC and...
2.9K
 02:25
Centrosome Duplication
4.0K
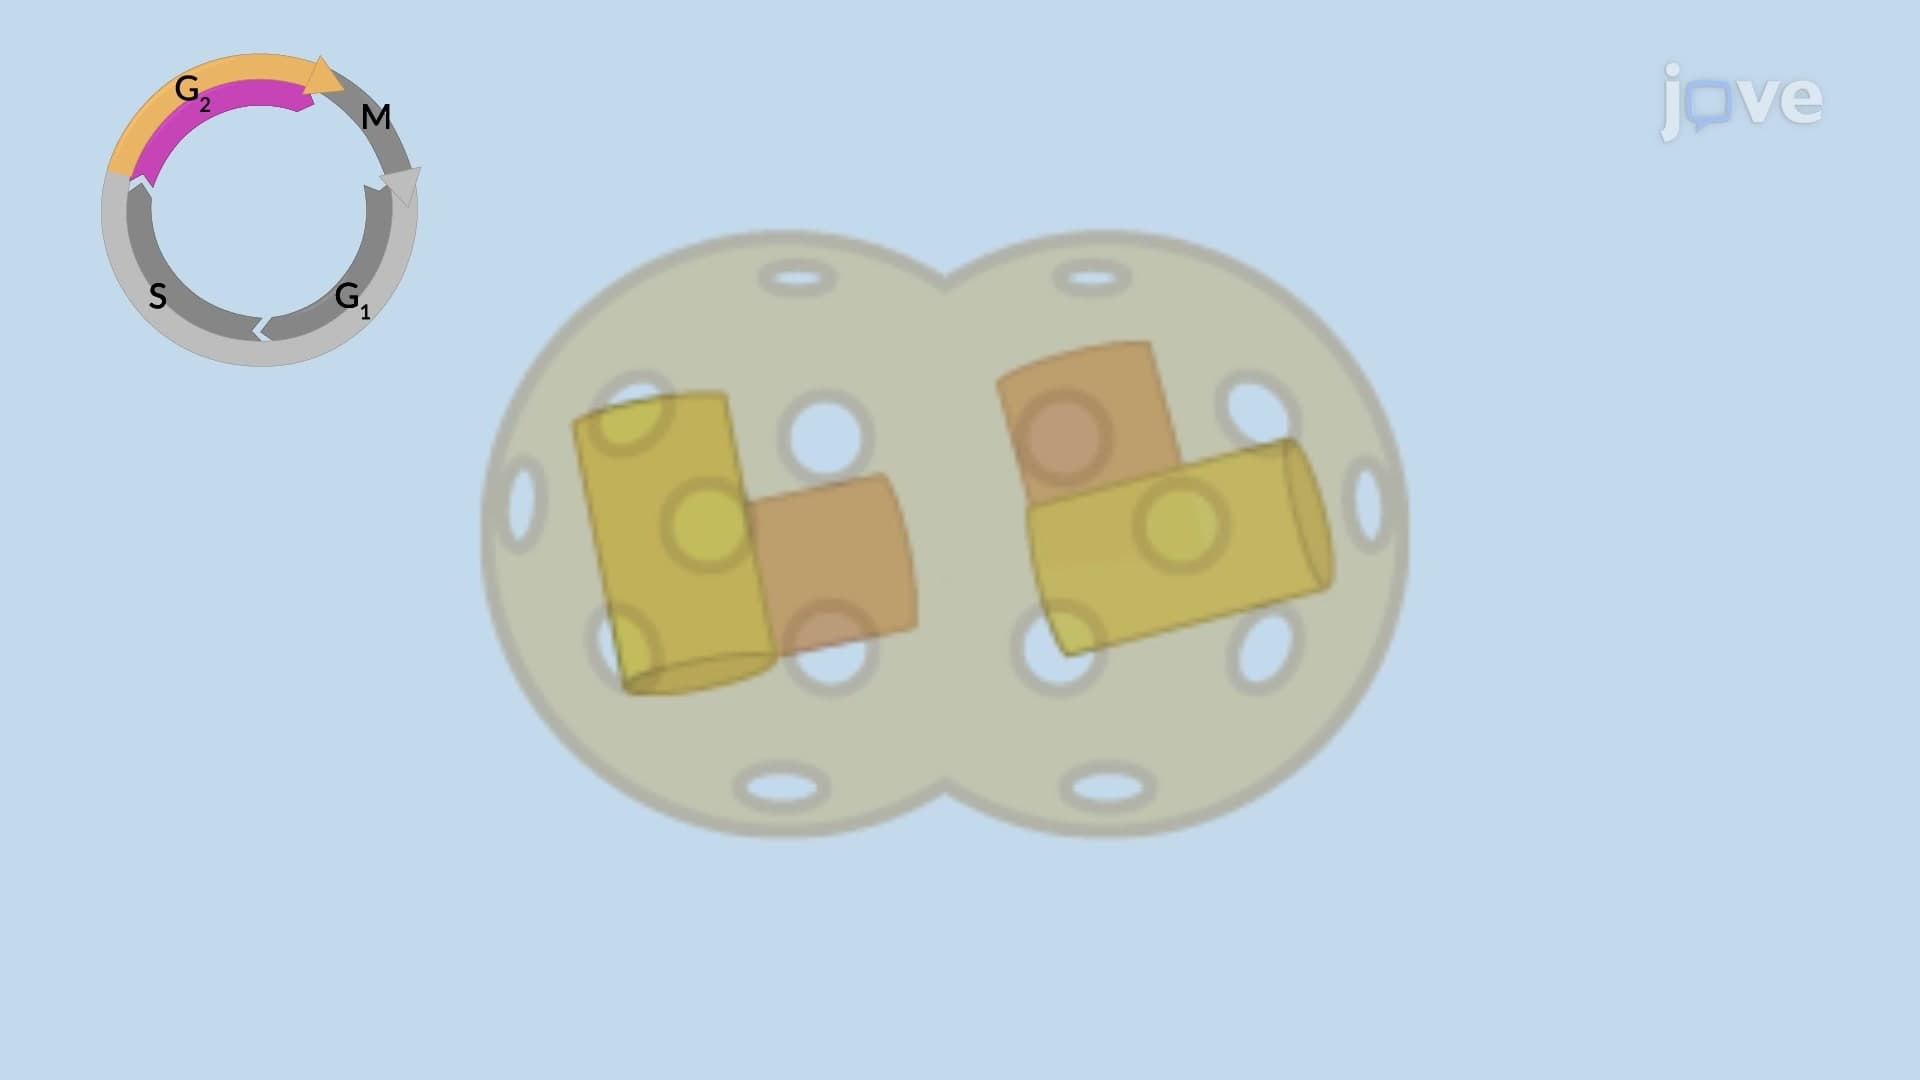
The primary microtubule organizing center (MTOC) in animal cells is the centrosome. A centrosome has two cylindrical centrioles at its core. Each centriole consists of nine sets of three microtubules held together by proteins. The centrioles are positioned at right angles to each other and surrounded by a shapeless protein cloud called the pericentriolar matrix, or pericentriolar material (PCM).
To ensure that each daughter cell receives a centrosome after cell division, centrosome duplication...
To ensure that each daughter cell receives a centrosome after cell division, centrosome duplication...
4.0K
 02:17
Microtubule Instability
5.1K
Microtubules are hollow cylindrical filaments having a diameter of approximately 25 nm and a length that varies from 200 nm to 25 μm. GTP-bound tubulin subunits form αβ-heterodimers for microtubule assembly. These core building blocks interact longitudinally, polymerizing into protofilaments. The protofilaments then interact with one another through lateral bonding forces to form stable cylindrical microtubules. These cylindrical filaments are dynamic as they undergo repeated...
5.1K
 02:17
Separation of Sister Chromatids
3.7K
At the transition from prophase to metaphase, there is a reduction in cohesion along the chromosomal arms, resulting in the resolution of sister chromatids. However, residual cohesin connections remain to hold the sister chromatids together until the transition from metaphase to anaphase. The residual connection prevents any premature separation of sister chromatids, blocking the risks of aneuploidy within the daughter cells.
At the onset of anaphase, separase, a proteolytic enzyme, is...
At the onset of anaphase, separase, a proteolytic enzyme, is...
3.7K
 02:02
Meiosis II
45.7K
Meiosis II entails cell division and segregation of the sister chromatids, resulting in the production of four unique haploid gametes. The steps for meiosis II are similar to mitosis, except that meiosis II occurs in haploid cells, whereas mitosis occurs in diploid cells.
The timing and cell division patterns of meiosis differ between males and females. In male meiosis, the centrosomes are part of the formation of the meiotic spindle. However, in oocytes, including that of humans, Drosophila,...
The timing and cell division patterns of meiosis differ between males and females. In male meiosis, the centrosomes are part of the formation of the meiotic spindle. However, in oocytes, including that of humans, Drosophila,...
45.7K
 02:30
Histone Variants at the Centromere
4.3K
Histone variants are the histone proteins with structural and sequence variations. These variants may be regarded as “mutant” forms that replace their canonical histone counterparts in the nucleosomes. Specific post-translational modifications on the histone variants enable further chromatin complexity and regulate tissue-specific gene expression. The most common histone variants are from histone H2A, H2B, and linker histone H1 families. However, several variants of histone H3...
4.3K