
在活体内,NAC和Zuotin/Hsp70陪伴系统在核糖体道出口处共存
Thomas Ziegelhoffer1, Amit K Verma1, Wojciech Delewski1
1Department of Biochemistry, University of Wisconsin-Madison, Madison, WI 53726, USA.
Nucleic acids research
|January 15, 2024

概括
新生的链关联复合体 (NAC) 和包括Zuotin在内的Hsp70伴侣系统可以同时结合核糖体. 这种定位允许高效的新生的多链折叠和成熟 in vivo.
科学领域:
- 分子生物学分子生物学
- 细胞生物学 细胞生物学
- 蛋白质折叠过程中的蛋白质折叠
背景情况:
- 60S核糖体子单元的退出道对于新生的多链折叠至关重要.
- 像新生链关联复合体 (NAC) 和Hsp70陪伴系统 (与Zuotin) 这样的蛋白质在核糖体上如何相互作用仍然不清楚.
研究的目的:
- 为了研究NAC和Hsp70-Zuotin系统在核糖体出口道的体内定位和相互作用.
主要方法:
- 在体内使用特定站点的交叉链接来研究蛋白质相互作用.
- 专注于NAC和Hsp70伴侣系统,特别是J域蛋白Zuotin.
主要成果:
- NAC和Zuotin在核糖体上交叉链接,即使没有活跃的翻译.
- 交叉链接数据表明,当Hsp70-Zuotin存在时,NAC的位置略有变化.
- Hsp70和Zuotin可以在道出口与NAC一起有效地参与新生的链条.
结论:
- 在体内,NAC和HSP70护航系统可以同时占据核糖体道的出口.
- 这种同时定位有助于高效的新生的多处理和折叠.
相关概念视频
 01:44
Termination of Translation
25.4K
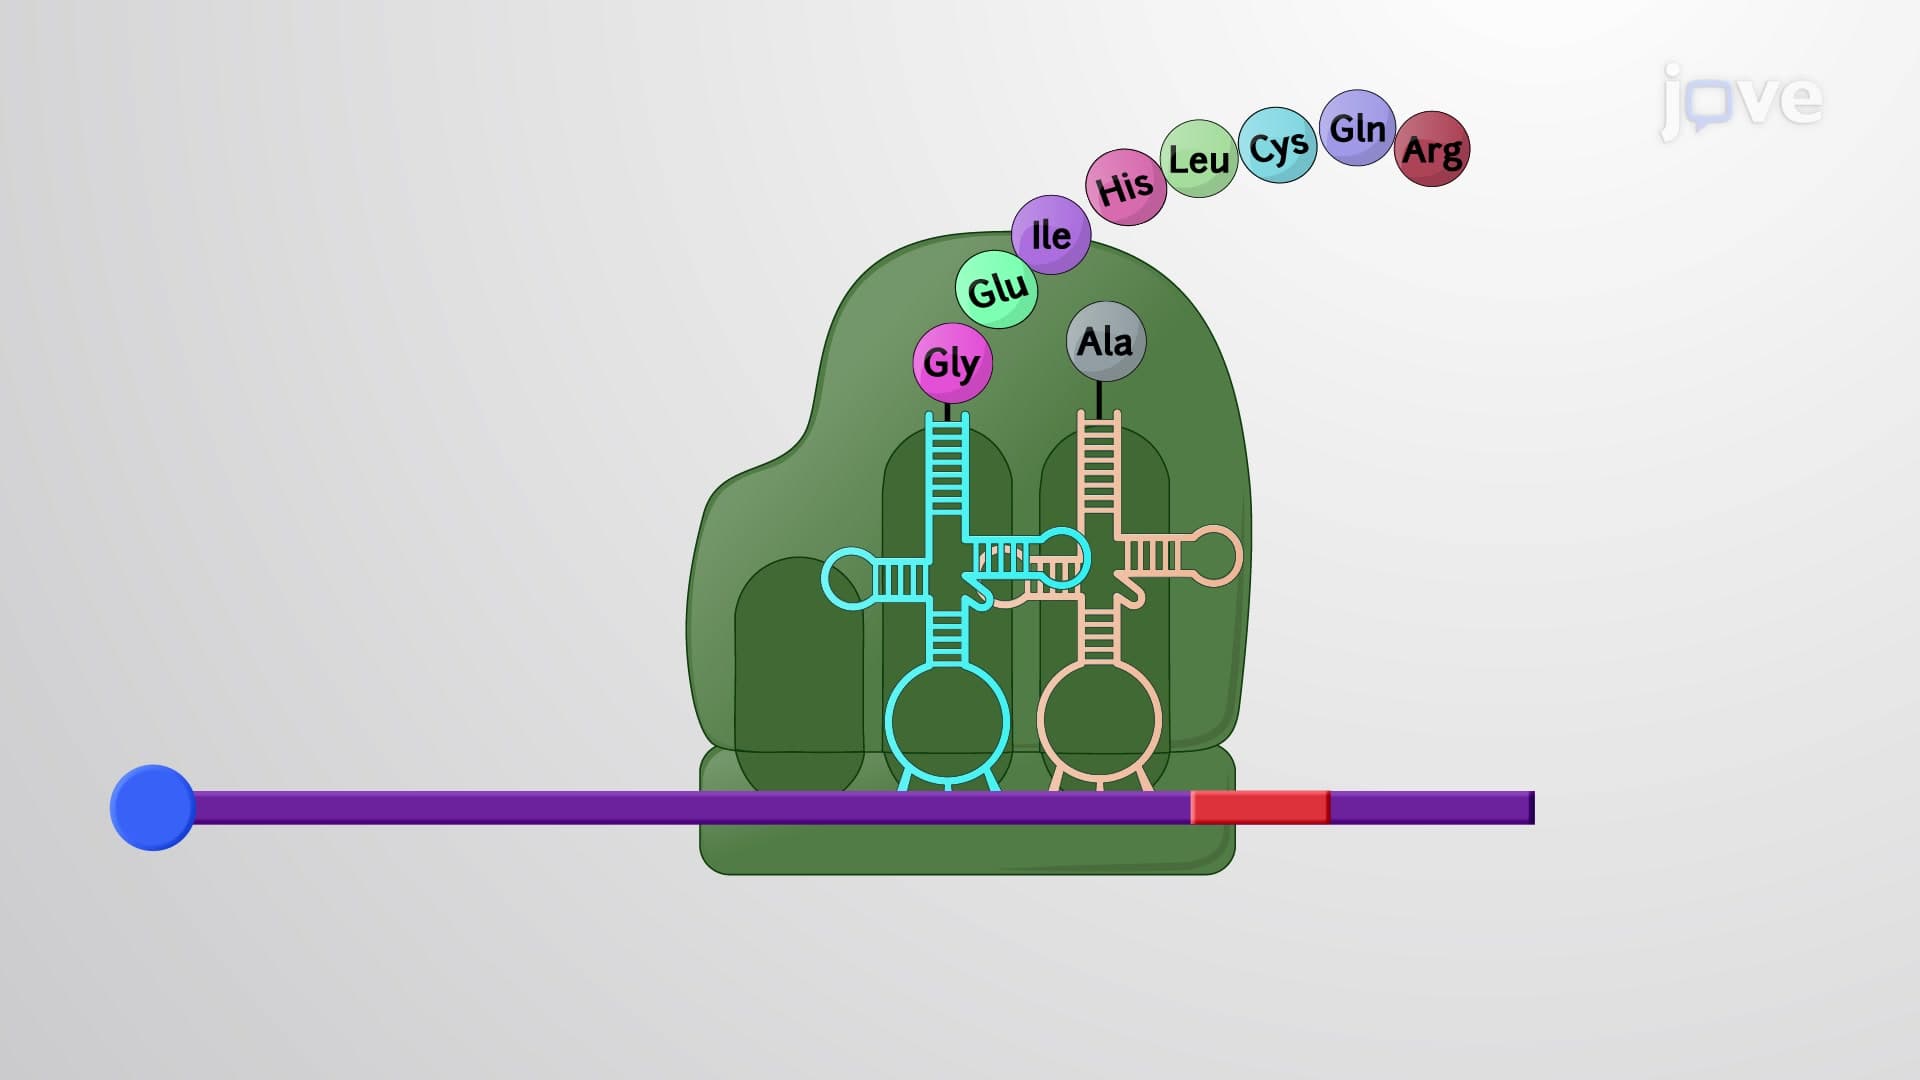
The large ribosomal subunit has several important structures essential to translation. These include the peptidyl transferase center (PTC) - which is the site where the peptide bond is formed - and a large, internal, water-filled tube through which the nascent polypeptide moves. This latter structure is called the Peptide Exit Tunnel, and it begins at the PTC and spans the body of the large ribosomal subunit. During translation, as the nascent polypeptide chain is synthesized, it passes through...
25.4K
 01:20
Cotranslational Protein Translocation
7.4K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
7.4K
 03:00
Molecular Chaperones and Protein Folding
18.0K
The native conformation of a protein is formed by interactions between the side chains of its constituent amino acids. When the amino acids cannot form these interactions, the protein cannot fold by itself and needs chaperones. Notably, chaperones do not relay any additional information required for the folding of polypeptides; the native conformation of a protein is determined solely by its amino acid sequence. Chaperones catalyze protein folding without being a part of the folded protein.
The...
The...
18.0K
 01:27
Post-translational Translocation of Proteins to the RER
5.7K
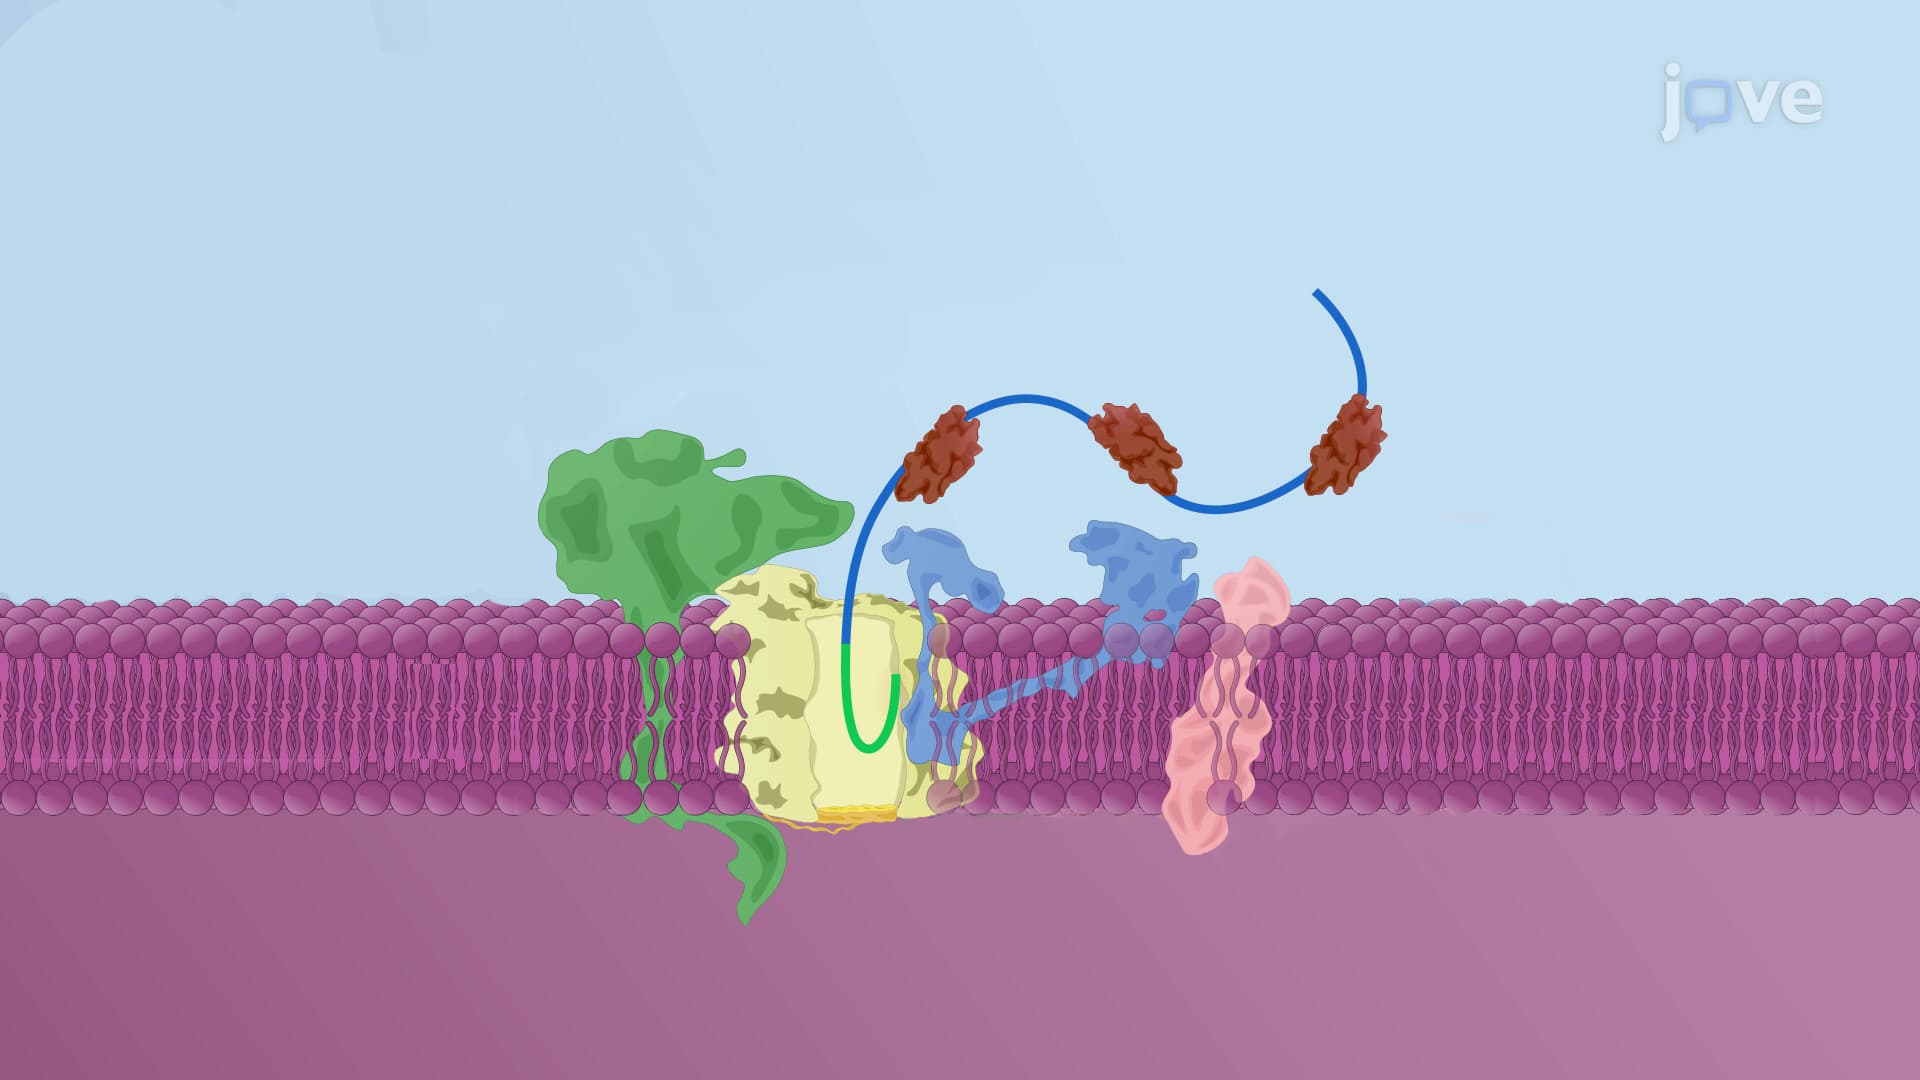
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
5.7K
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.3K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.3K
 01:45
Regulation of Nuclear Protein Sorting
2.4K
Nuclear protein sorting regulates nucleus composition and gene expression, crucial for determining the fate of a eukaryotic cell. Hence, the entry and exit of molecules across the nuclear envelope is a tightly controlled process. Nuclear protein sorting can be inhibited by one of the following ways: 1) masking cargo signal sequences, 2) modifying the nuclear receptor's affinity for cargo, 3) controlling the nuclear pore size, 4) retaining the cargo during its transit to the cytosol or the...
2.4K