
UFM1 E3酶识别并释放来自ER转位的60S核糖体
Linda Makhlouf1, Joshua J Peter2, Helge M Magnussen2
1Astbury Centre for Structural Molecular Biology, School of Molecular and Cellular Biology, Faculty of Biological Sciences, University of Leeds, Leeds, UK.
Nature
|February 21, 2024

概括
UFM1核糖体E3连接酶 (UREL) 复合物修改停滞的核糖体,促进它们从ER膜释放. 这种UFMylation过程对蛋白质平衡至关重要,并且通过将它们与SEC61转位素分离而循环利用核糖体.
科学领域:
- 分子生物学
- 细胞生物学
- 结构生物学
背景情况:
- 在内分泌网膜 (ER) 中停滞不前的核糖体会受到60S核糖体子单元 (RPL26) 上的泛胺类蛋白UFM1的修饰.
- 这一过程被称为UFMylation,由由UFL1,UFBP1和CDK5RAP3组成的UFM1核糖体E3联结酶 (UREL) 复合体介导.
- 精确的UREL催化机制和UFMylation的功能结果在很大程度上仍未确定.
研究的目的:
- 阐明UREL基质特异性的结构基础.
- 了解UFMylation在核糖体循环和蛋白质平衡中的功能后果.
- 研究UFMylation在SE61转位体中的核糖体解离中的作用.
主要方法:
- 使用冷电子显微镜 (cryo-EM) 来确定与60S核糖体结合的UREL复合物的结构.
- 生物化学测定用于评估UFMylation的必要性,以释放60S子单元中的SEC61.
- 分析了UREL的结构特征和功能状态 ("写字器"和"阅读器"模块).
主要成果:
- 低温EM结构显示,UREL在60S子单元周围形成C形,阻塞了tRNA结合部位和出口道.
- 在UREL中的UFL1循环重塑转移酶中心,表明它在核糖体释放和循环中发挥作用.
- 功能性研究表明,UFMylation对于将60S子单元与SEC61转位元分离至关重要,防止它们在ER膜上积累.
结论:
- UREL的状结构及其与基转移酶中心的相互作用是其在核糖体释放中的关键功能.
- UFMylation是从ER膜中释放停滞的核糖体的一个关键步骤,确保有效的蛋白质平衡.
- UREL既是UFMylation的"写入器"又是"读取器",突出显示了对核糖体循环的独特监管机制.
相关概念视频
 01:28
Protein Translocation Machinery on the ER Membrane
4.6K
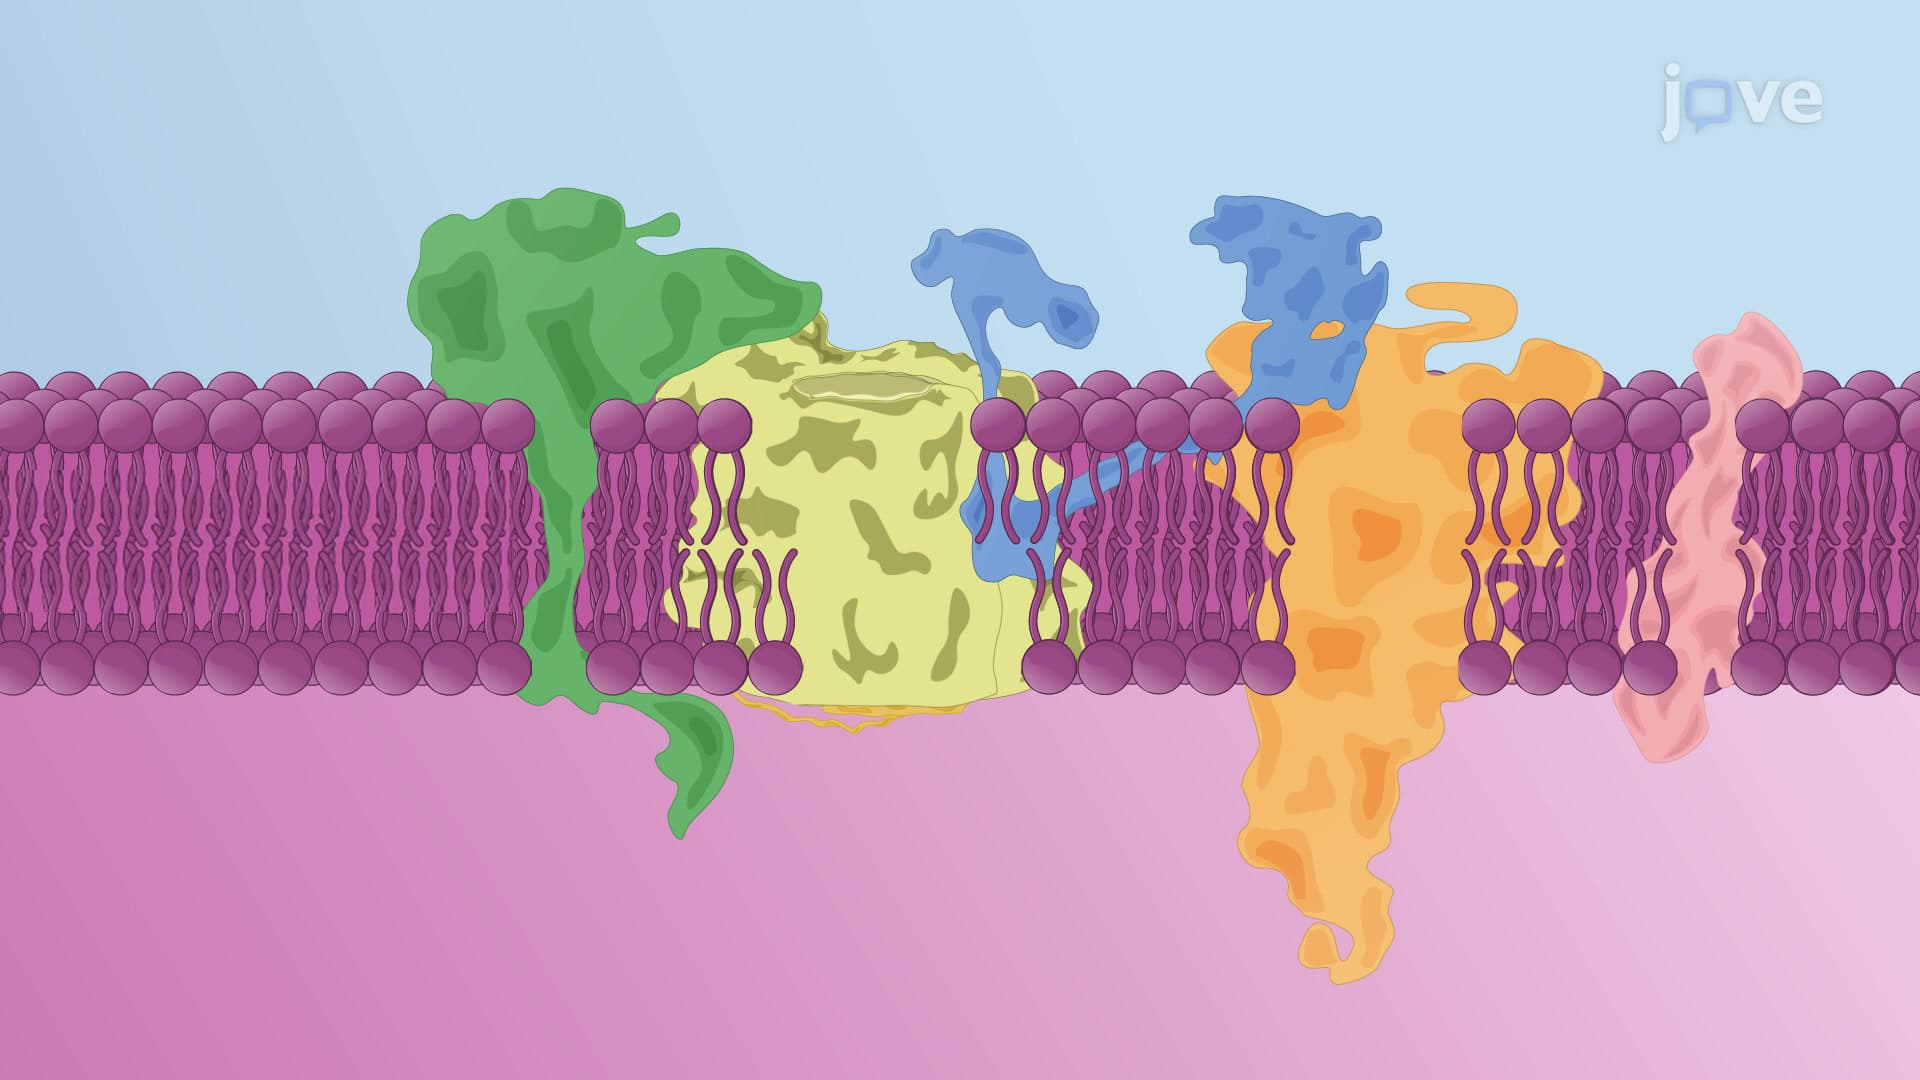
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
4.6K
 01:20
Cotranslational Protein Translocation
7.4K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
7.4K
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.3K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.3K
 01:27
Post-translational Translocation of Proteins to the RER
5.7K
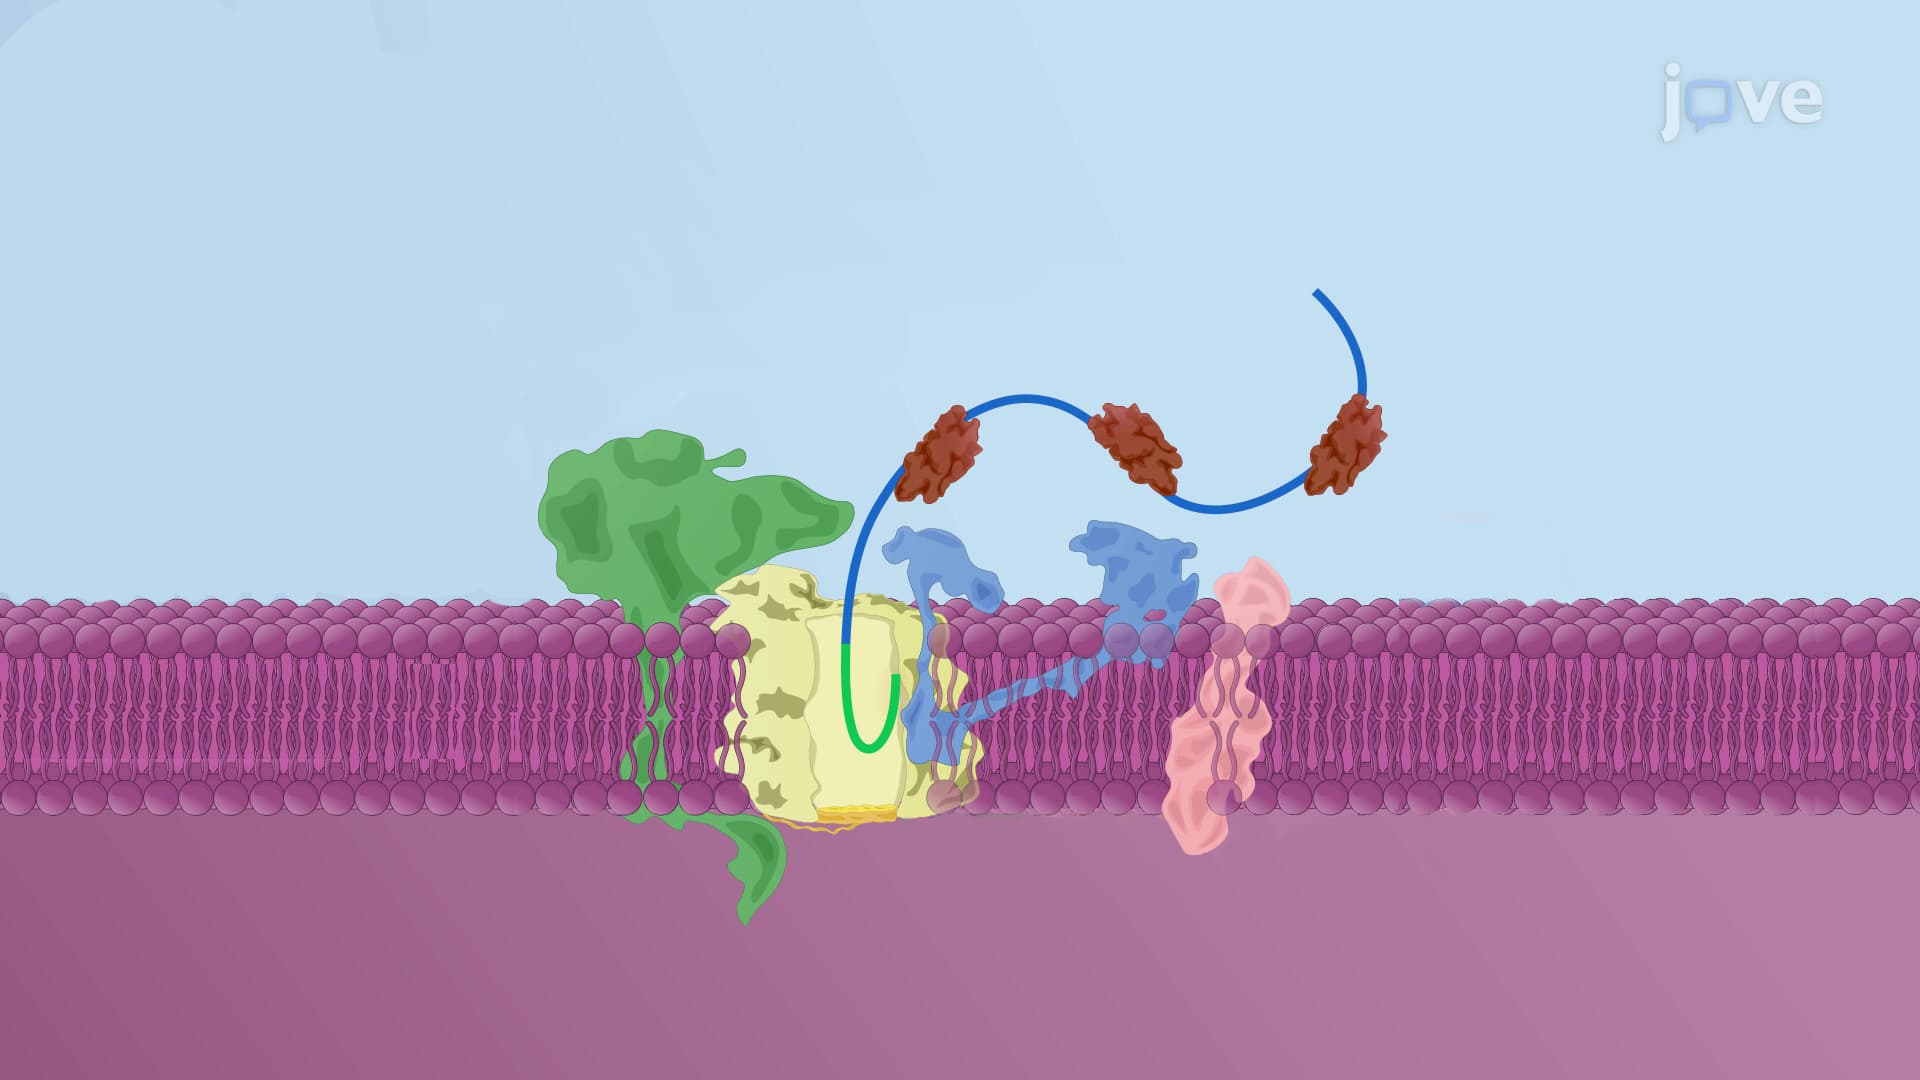
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
5.7K
 02:07
Improving Translational Accuracy
10.4K
Base complementarity between the three base pairs of mRNA codon and the tRNA anticodon is not a failsafe mechanism. Inaccuracies can range from a single mismatch to no correct base pairing at all. The free energy difference between the correct and nearly correct base pairs can be as small as 3 kcal/ mol. With complementarity being the only proofreading step, the estimated error frequency would be one wrong amino acid in every 100 amino acids incorporated. However, error frequencies observed in...
10.4K
 01:27
Ribosomes
7.6K
Ribosomes translate genetic information encoded by messenger RNA (mRNA) into proteins. Both prokaryotic and eukaryotic cells have ribosomes. Cells that synthesize large quantities of protein—such as secretory cells in the human pancreas—can contain millions of ribosomes.
Ribosome Structure and Assembly
Ribosomes are composed of ribosomal RNA (rRNA) and proteins. In eukaryotes, rRNA is transcribed from genes in the nucleolus—a part of the nucleus that specializes in ribosome...
Ribosome Structure and Assembly
Ribosomes are composed of ribosomal RNA (rRNA) and proteins. In eukaryotes, rRNA is transcribed from genes in the nucleolus—a part of the nucleus that specializes in ribosome...
7.6K