
与蛋白质局部化机制相关的细菌翻译逮捕的分散和广泛分布
Keigo Fujiwara1,2, Naoko Tsuji3,4, Mayu Yoshida3,4
1Faculty of Life Sciences, Kyoto Sangyo University, Motoyama, Kamigamo, Kita-Ku, Kyoto, 603-8555, Japan. kigfujiwara@cc.kyoto-su.ac.jp.
Nature communications
|April 2, 2024

概括
研究人员发现了新的与Sec/YidC相关的细菌逮捕,阻断了翻译. 这些,在各种细菌中发现,表明核糖体相互作用的共同进化起源.
科学领域:
- 分子生物学分子生物学
- 基因组学就是基因组学.
- 进化生物学 进化生物学
背景情况:
- 调控性停止对于通过停止翻译来控制细菌基因表达至关重要.
- 与Sec/YidC相关的蛋白质参与蛋白质分泌和膜插入,在转化调节中具有潜在的作用.
研究的目的:
- 在广泛的细菌物种中识别与Sec/YidC相关的新型逮捕.
- 调查这些已识别的逮捕的遗传分布和功能特征.
主要方法:
- 对超过3万个细菌基因组序列的生物信息分析.
- 在体内和体外实验验证确定逮捕的验证.
- 遗传学分析以确定分布模式.
主要成果:
- 识别了许多Sec/YidC相关的逮捕,在细菌中分布不齐但广泛.
- 证明了几种已识别的,尽管保留了C端序列,但有效地阻断了细菌核糖体.
- 在许多逮捕中发现一种常见的R-A-P-P类似序列动机.
结论:
- 与Sec/YidC相关的逮捕是细菌中一个重要的,但以前被低估的调节机制.
- 已识别的R-A-P-P样动图可能代表一种进化保存的元素,使其能够与多种细菌核糖体相互作用.
相关概念视频
 01:27
Post-translational Translocation of Proteins to the RER
5.7K
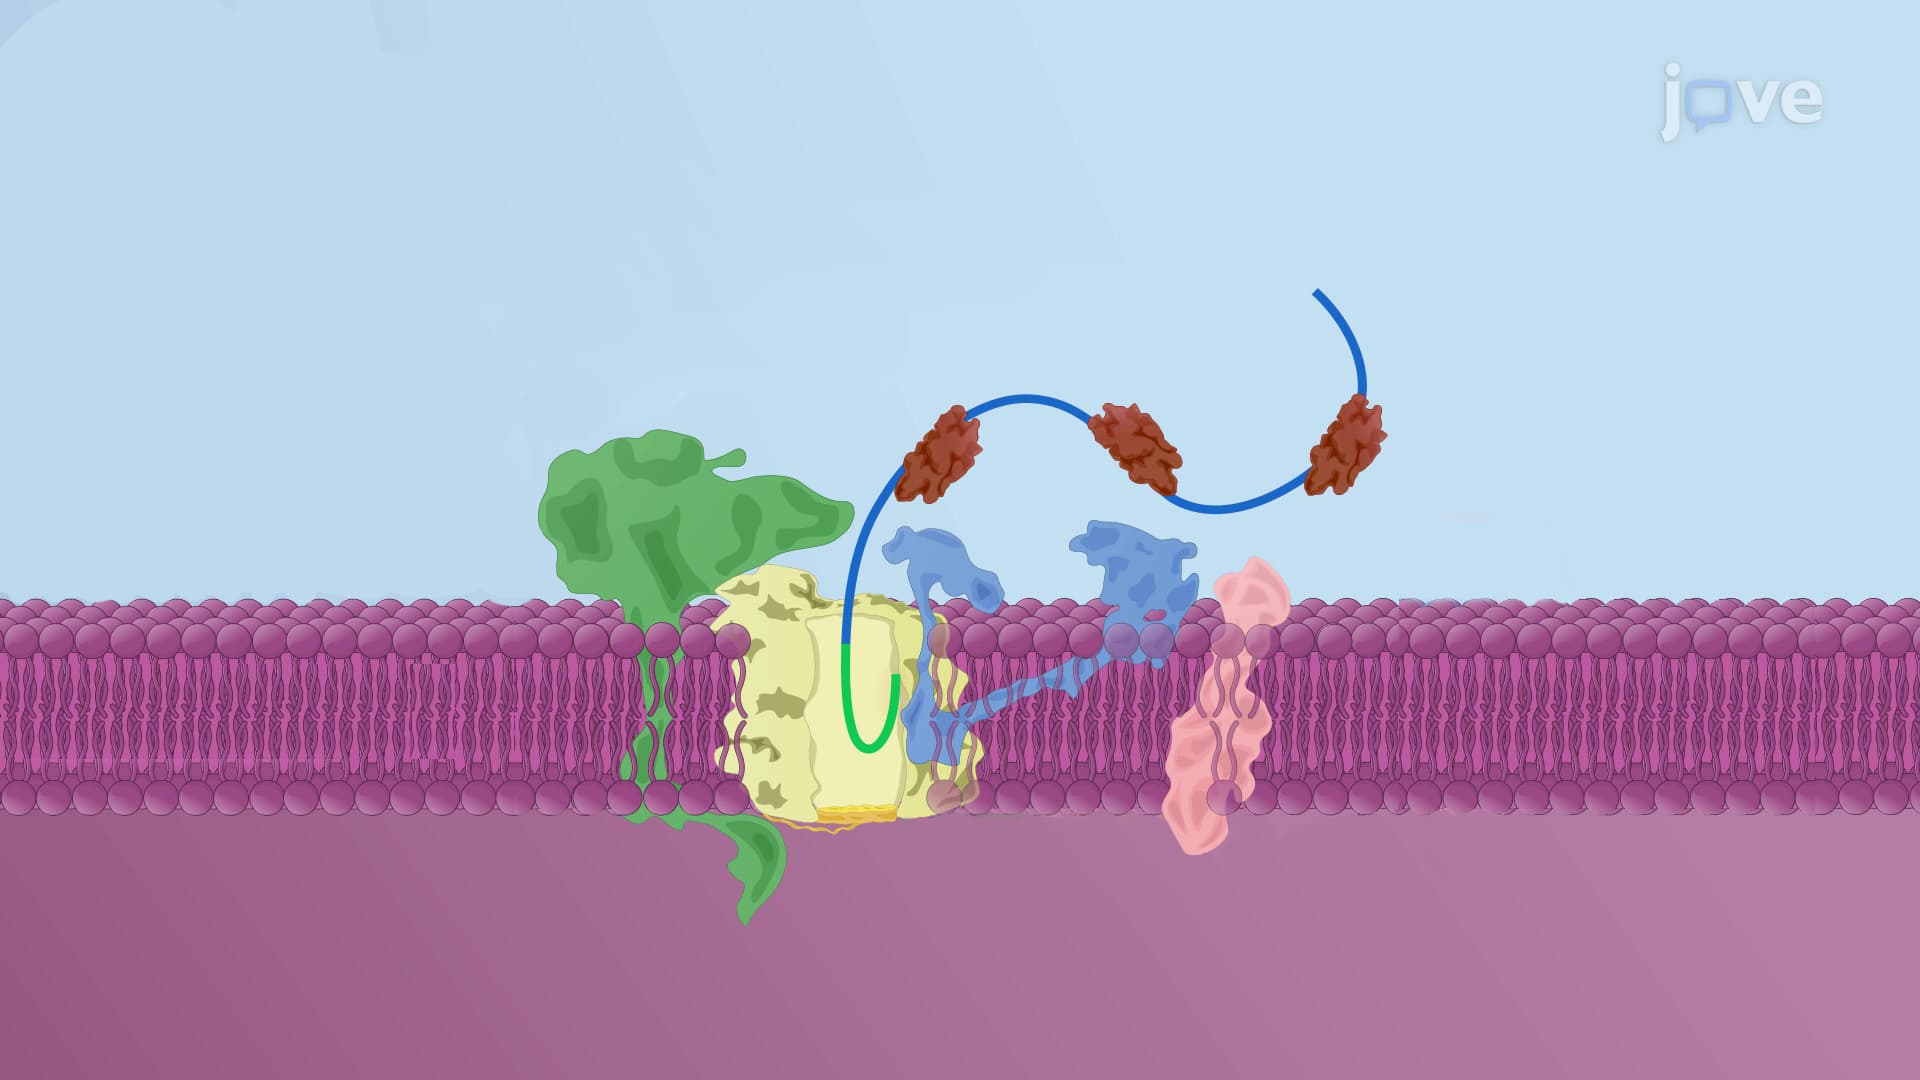
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
5.7K
 02:22
Regulated mRNA Transport
6.3K
In eukaryotes, transcription and translation are compartmentalized; an mRNA is first synthesized in the nucleus and then selectively transported to the cytoplasm for protein synthesis. Before transport, a pre-mRNA undergoes several steps of post-transcriptional modifications including splicing, 5' capping, and the addition of a poly-adenine tail. Various proteins bind to the pre-mRNA during these modifications. The mRNA transport takes place with the help of multiple proteins playing...
6.3K
 01:20
Cotranslational Protein Translocation
7.3K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
7.3K
 01:44
Termination of Translation
25.4K
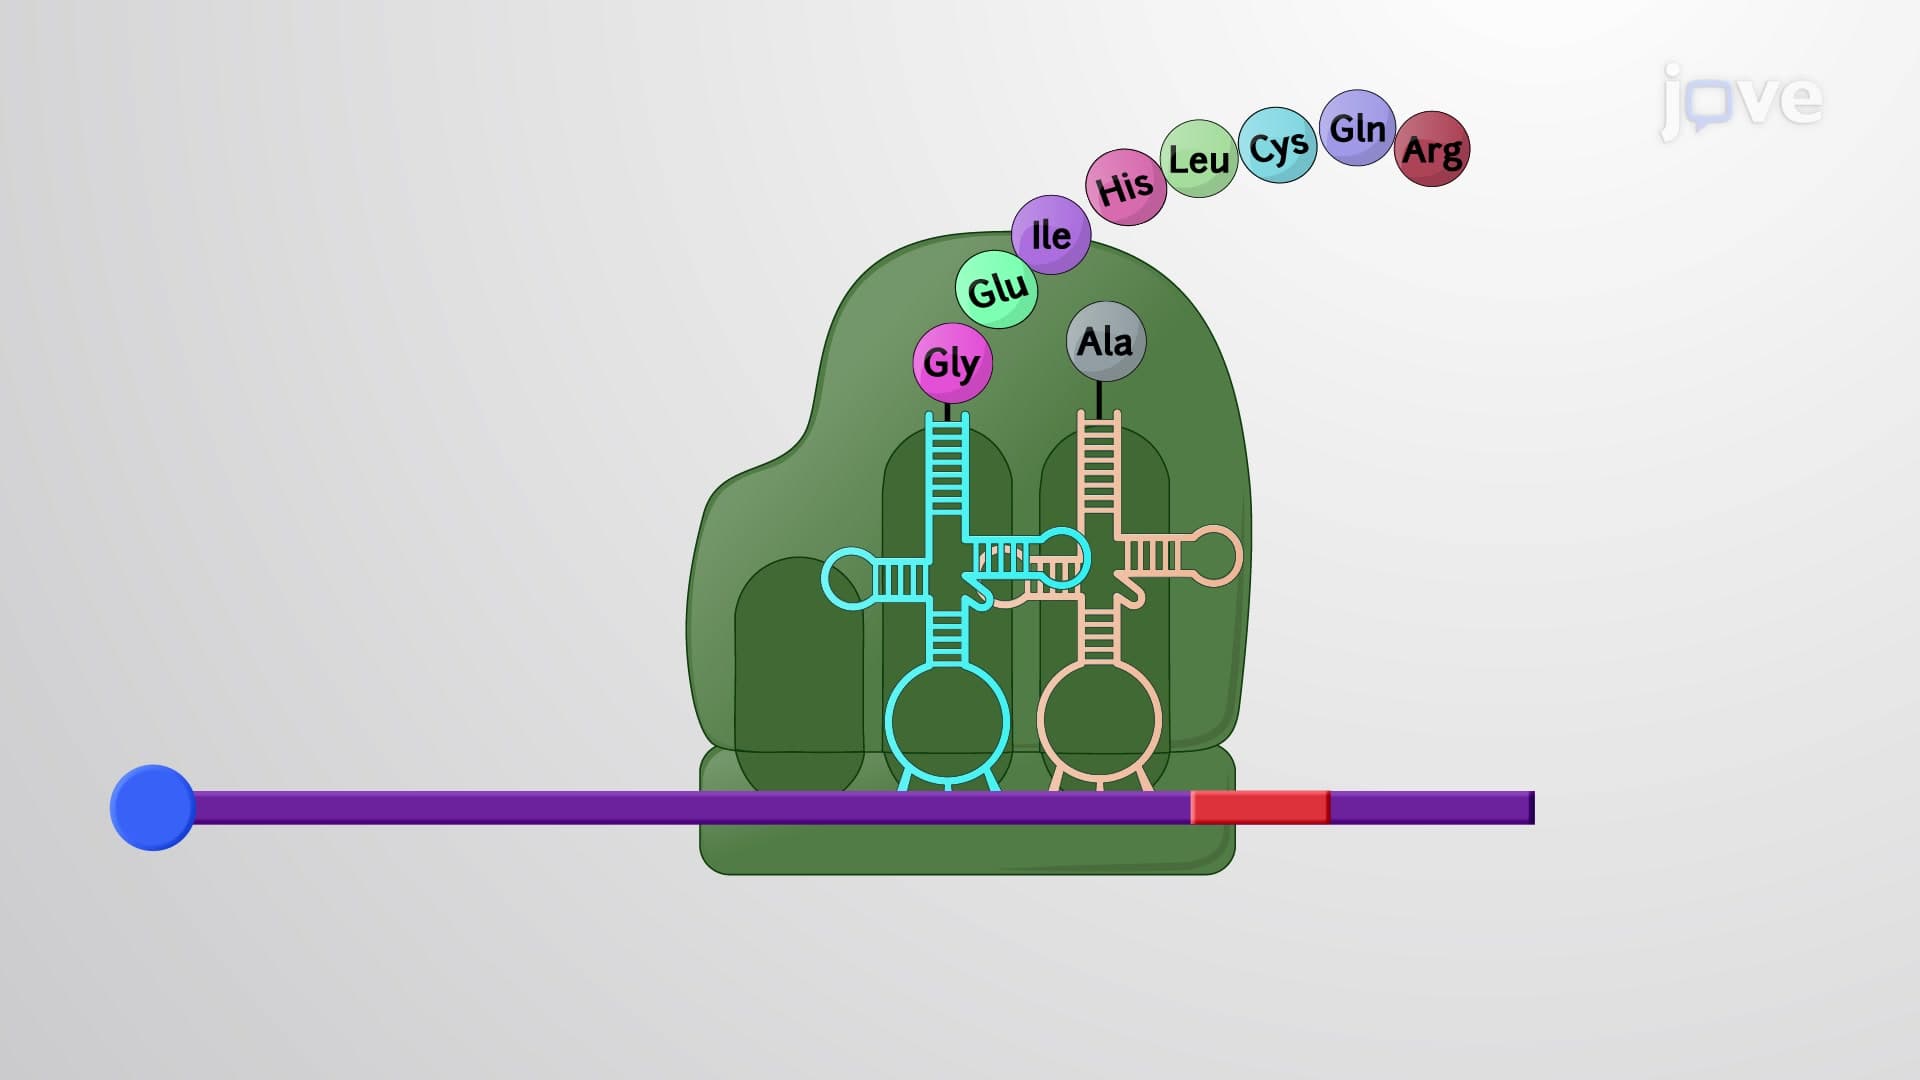
The large ribosomal subunit has several important structures essential to translation. These include the peptidyl transferase center (PTC) - which is the site where the peptide bond is formed - and a large, internal, water-filled tube through which the nascent polypeptide moves. This latter structure is called the Peptide Exit Tunnel, and it begins at the PTC and spans the body of the large ribosomal subunit. During translation, as the nascent polypeptide chain is synthesized, it passes through...
25.4K
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.2K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.2K
 02:07
Improving Translational Accuracy
10.3K
Base complementarity between the three base pairs of mRNA codon and the tRNA anticodon is not a failsafe mechanism. Inaccuracies can range from a single mismatch to no correct base pairing at all. The free energy difference between the correct and nearly correct base pairs can be as small as 3 kcal/ mol. With complementarity being the only proofreading step, the estimated error frequency would be one wrong amino acid in every 100 amino acids incorporated. However, error frequencies observed in...
10.3K