通过TOM20将poly (rC) 结合蛋白-2与 sideroflexin-3结合在一起,作为铁进入线粒体的途径
Danyang Mi1, Izumi Yanatori1,2, Hao Zheng1
1Department of Pathology and Biological Responses, Nagoya University Graduate School of Medicine, Nagoya, Japan.
Free radical research
|April 10, 2024

概括
研究人员发现了一条新的铁进入线粒体的途径. 这涉及细胞体Fe(II) 伴侣PCBP2与TOM20和SFXN3相互作用,影响细胞铁水平和呼吸.
科学领域:
- 细胞生物学 细胞生物学
- 线粒体生物学 线粒体生物学
- 铁的代谢 铁的代谢
背景情况:
- 铁对细胞功能至关重要,线粒体将其用于和Fe-S集群.
- PCBP2是铁 (Fe) 的一个关键的细胞分裂伴侣.
- 了解线粒体铁进口对于细胞健康和疾病至关重要.
研究的目的:
- 为了确定细胞质铁伴侣PCBP2.2.的线粒体受体.
- 为了阐明铁进入线粒体的途径.
- 调查已识别的蛋白质在线粒体铁稳态和细胞呼吸中的作用.
主要方法:
- 谷氨S转移酶拉下测试和LC-MS用于识别PCBP2相互作用的线粒体蛋白质.
- 刺激性排放枯竭显微镜和蛋白酶-K消化以确定蛋白质定位.
- 同免疫沉积和近距离结合试验,以评估蛋白质相互作用.
- 基因淘汰和淘汰实验 (PCBP2,SFXN3,MFRN1) 来评估对线粒体铁和呼吸的功能影响.
主要成果:
- 确定了TOM20,SFXN3,SFXN1和TOM70作为潜在的线粒体PCBP2受体.
- TOM20局限于外层线粒体膜,SFXN3局限于内层线粒体膜.
- PCBP2是TOM20的近邻,它直接与SFXN3结合.
- 击败PCBP2或SFXN3降低了线粒体Fe (II) 和呼吸.
- 与MFRN1淘汰赛相比,SFXN3淘汰赛明显影响了铁的稳态.
- 过度表达SFXN3导致细胞质铁缺乏,线粒体Fe (II) 过量,以及铁的敏感性.
结论:
- 通过PCBP2-TOM20-SFXN3轴发现了细胞质铁进入线粒体的新途径.
- 这一途径在调节线粒体铁水平,血红蛋白合成和细胞呼吸方面发挥着重要作用.
- 这些发现提供了对线粒体铁代谢及其对细胞过程 (如铁亡) 的影响的新见解.
相关概念视频
 01:28
The Early Endosome: Endocytosis of Transferrin
3.3K
Essential proteins such as insulin or low-density lipoprotein (LDL) and micronutrients such as iron enter a eukaryotic cell through receptor-mediated endocytosis. Subsequently, the early endosomes fuse with the vesicles containing such receptor-ligand complexes and play a vital role in sorting the incoming ligands and receptors. While the ligands are either degraded inside the vesicle or released into the cytosol, their receptors are returned to the plasma membrane for further rounds of...
3.3K
 01:19
Translocation of Proteins into the Mitochondria
3.1K
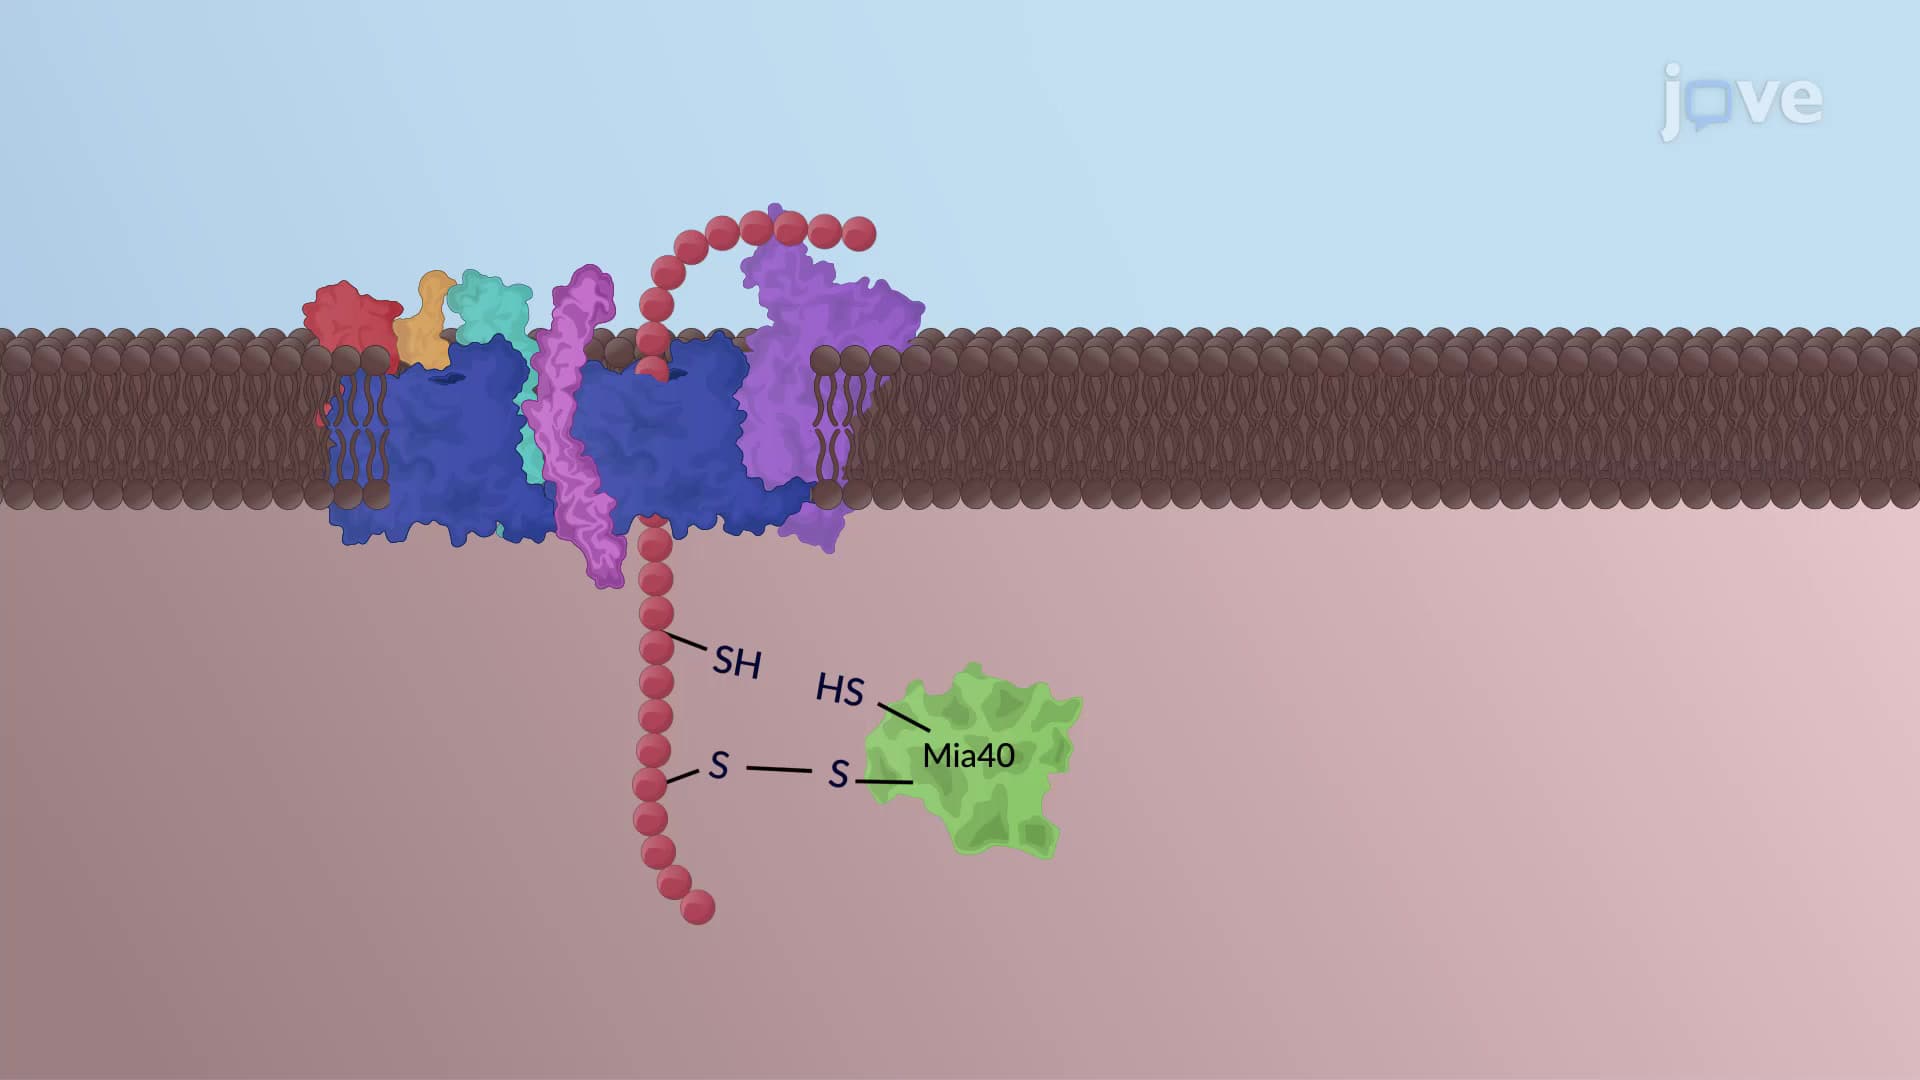
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.1K
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
7.2K
The organelle-specific signaling sequences direct proteins synthesized in the cytosol to their final destination like ER, mitochondria, peroxisomes, etc. Some of the proteins directed to ER are then trafficked via vesicles to other organelles within the cell or the extracellular environment through the Golgi complex. For example, the rough ER synthesizes soluble proteins for transportation to the lysosomes or secretion out of the cell. It can also synthesize transmembrane proteins that can...
7.2K
 01:39
Mitochondrial Protein Sorting
4.3K
Mitochondria are double-membrane organelles of the eukaryotes involved in cellular metabolism, signaling, ATP synthesis, and programmed cell death. Each of these processes requires specific proteins and enzymes that must be correctly sorted to the right mitochondrial subcompartment for the proper functioning of the organelle.
Most of these mitochondrial proteins are encoded by the nucleus and imported to the mitochondria as unfolded or loosely folded precursors. Mitochondrial precursors...
Most of these mitochondrial proteins are encoded by the nucleus and imported to the mitochondria as unfolded or loosely folded precursors. Mitochondrial precursors...
4.3K
 01:45
Regulation of Nuclear Protein Sorting
2.4K
Nuclear protein sorting regulates nucleus composition and gene expression, crucial for determining the fate of a eukaryotic cell. Hence, the entry and exit of molecules across the nuclear envelope is a tightly controlled process. Nuclear protein sorting can be inhibited by one of the following ways: 1) masking cargo signal sequences, 2) modifying the nuclear receptor's affinity for cargo, 3) controlling the nuclear pore size, 4) retaining the cargo during its transit to the cytosol or the...
2.4K
 01:26
Protein Modifications in the RER
5.1K
Modification of secretory and transmembrane proteins entering the rough ER begins in the ER lumen. These modifications aid in protein folding and stabilize the acquired tertiary structure. Protein modifications in the rough ER co-occur at different stages of protein folding.
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal...
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal...
5.1K