
瓜核酸交换因子DOCK11在HBV进入和在肝细胞中的持久性方面所起的作用
Ying-Yi Li1, Kazuhisa Murai2, Junyan Lyu2
1Department of Gastroenterology, Kanazawa University Graduate School of Medicine, 13-1, Takaramachi, Kanazawa 920-8640, Japan.
Viruses
|May 25, 2024

概括
细胞动力学11分辨器 (DOCK11) 蛋白质通过使病毒DNA转录和复制成为可能,有助于乙型肝炎病毒 (HBV) 的持久性. 用10M-D42AN抑制DOCK11抑制HBV,为慢性乙型肝炎提供了潜在的治疗策略.
科学领域:
- 肝病学 肝病学是一种肝病学.
- 病毒学 病毒学
- 分子生物学分子生物学
背景情况:
- 乙型肝炎病毒 (HBV) 感染持久性与病毒共价封闭圆形DNA (cccDNA) 有关.
- 细胞动力学11分辨器 (DOCK11),为CDC42的关氨核酸交换因子 (GEF),与HBV持久性有关.
研究的目的:
- 阐明DOCK11在HBV复制和持久性中的作用.
- 为了研究DOCK11与病毒成分和宿主细胞机械的相互作用.
- 评估DOCK11抑制作为慢性乙型肝炎 (CHB) 的治疗策略.
主要方法:
- 免疫光和共免疫沉以研究DOCK11局部化和相互作用.
- 在存在或缺少DOCK11.的情况下,对HBV复制和ccccDNA转录的分析.
- 在体外和体内使用DOCK11结合10M-D42AN和恩特卡维尔的研究.
主要成果:
- DOCK11为HBV从早期内分泌体到跨戈尔吉网络和内分泌网膜提供了替代的逆行贩运途径,避免了溶解体降解.
- DOCK11通过与H3K4me3和RNA聚合酶II结合来促进HBV的ccDNA转录.
- DOCK11对于ccDNA合成至关重要,10M-D42AN对其的抑制抑制了HBV复制.
- 与10M-D42AN和恩特卡维尔联合治疗在抑制HBV方面显示出有希望的结果.
结论:
- DOCK11是HBV持久性的关键宿主因素,参与病毒贩运,ccccDNA转录和复制.
- 用像10M-D42AN这样的抑制剂准DOCK11代表了CHB的潜在治疗途径.
- DOCK11是开发针对CHB的向治疗的有希望的候选分子.
相关概念视频
 01:33
Coat Assembly and GTPases
3.5K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.5K
 01:14
Rab Proteins
3.9K
Rab proteins constitute the largest family of monomeric GTPases, of which 70 members are present in humans. Rab proteins and their effectors regulate consecutive stages of vesicle transport such as vesicle transport, docking, and fusion to the correct recipient membrane.
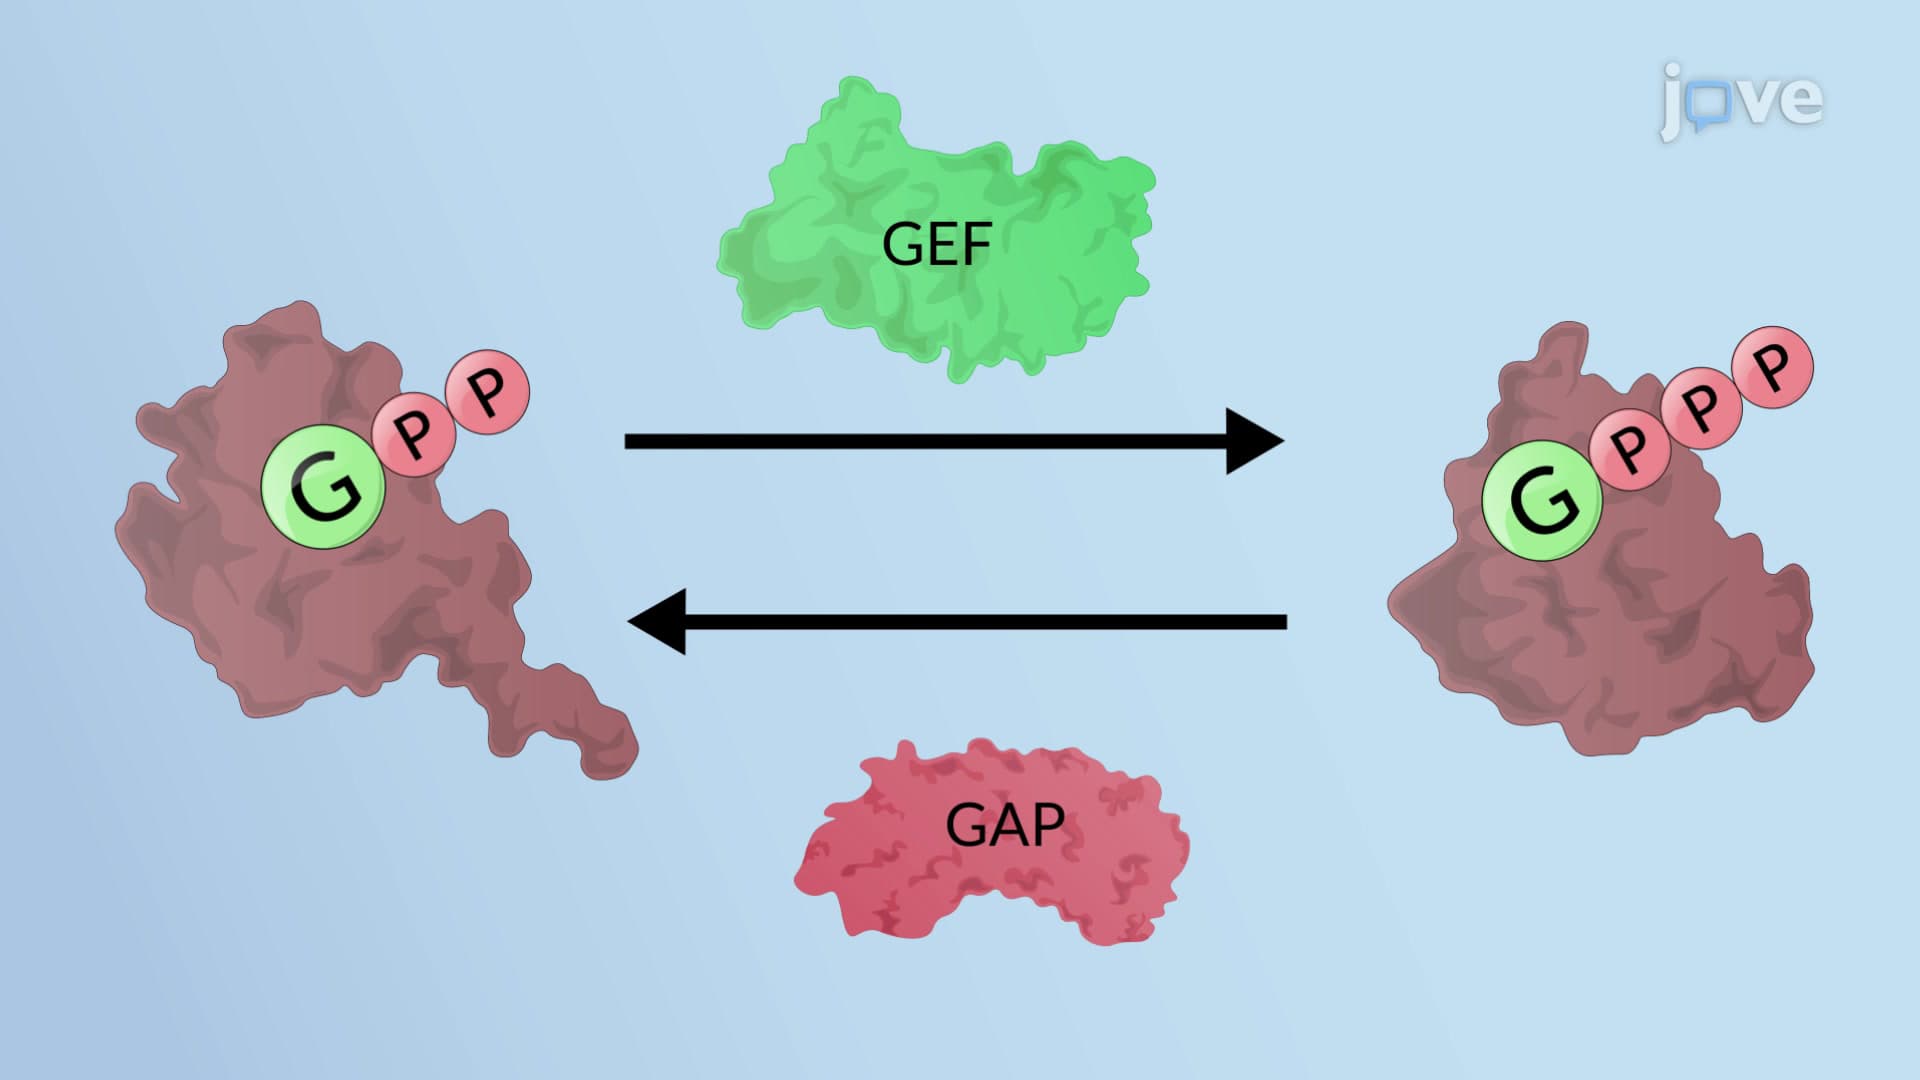
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
3.9K
 01:45
Regulation of Nuclear Protein Sorting
2.4K
Nuclear protein sorting regulates nucleus composition and gene expression, crucial for determining the fate of a eukaryotic cell. Hence, the entry and exit of molecules across the nuclear envelope is a tightly controlled process. Nuclear protein sorting can be inhibited by one of the following ways: 1) masking cargo signal sequences, 2) modifying the nuclear receptor's affinity for cargo, 3) controlling the nuclear pore size, 4) retaining the cargo during its transit to the cytosol or the...
2.4K
 01:29
GPI Anchoring of Proteins in the ER Membrane
4.0K
GPI-anchoring is a post-translational, reversible protein modification that is ubiquitous in eukaryotes. Such proteins are primarily present on the exoplasmic leaflet of the plasma membrane.
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
4.0K
 01:32
Pinching-off of Coated Vesicles
3.1K
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
3.1K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.1K
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.1K