
塔马插酶的POTRA域与外膜相互作用并调节膜性质
Abdelkader Mellouk1,2, Paul Jaouen2,3, Louis-Jacques Ruel2,4,5
1Institut National de la Rechyuerche Scientifique (INRS), Centre Armand-Frappier Santé Biotechnologie, Laval, QC H7V 1B7, Canada.

概括
转移和组装模块 (TAM) 的监护人
科学领域:
- 细菌外膜蛋白质生物生成 细菌外膜蛋白质生物生成
- 蛋白质运输的分子机制
- 格拉姆阴性细菌的细胞外结构结构.
背景情况:
- 阴性细菌具有独特的外膜 (OM),对细胞功能和毒性至关重要.
- 外膜蛋白 (OMP) 是 OM 的重要组成部分,需要专门的机器来组装它们.
- 转位和组装模块 (TAM) 是一个关键的伴侣系统,参与OMP生物发生.
研究的目的:
- 研究TAMA的POTRA域在OMP组装和膜相互作用中的作用.
- 阐明TAM调节细菌外膜特性的机制.
- 为了确定TAM和OM脂质环境之间的特定相互作用.
主要方法:
- 用X射线晶体学来确定TAM组件的结构.
- 分子动力学模拟用于分析蛋白质膜相互作用.
- 生物分子相互作用研究以量化结合亲缘关系.
主要成果:
- 塔马的POTRA域与OM的内部表面相互作用.
- 在POTRA域1和2上确定了一个特定的结合位点.
- 塔玛A对酸糖醇表现出偏好,这是促进OMP组装的脂质.
- 这些相互作用调节膜性质,并可能有助于OMP生物发生.
结论:
- TAM的POTRA域在招募TAMB和与OM互动方面发挥着双重作用.
- 由Tama调解的脂质相互作用有助于有效的OMP组装.
- 这项研究为细菌外膜蛋白生物发生的复杂过程提供了新的见解.
更多相关视频
相关概念视频
 01:12
Porin Insertion in the Outer Mitochondrial Membrane
2.9K
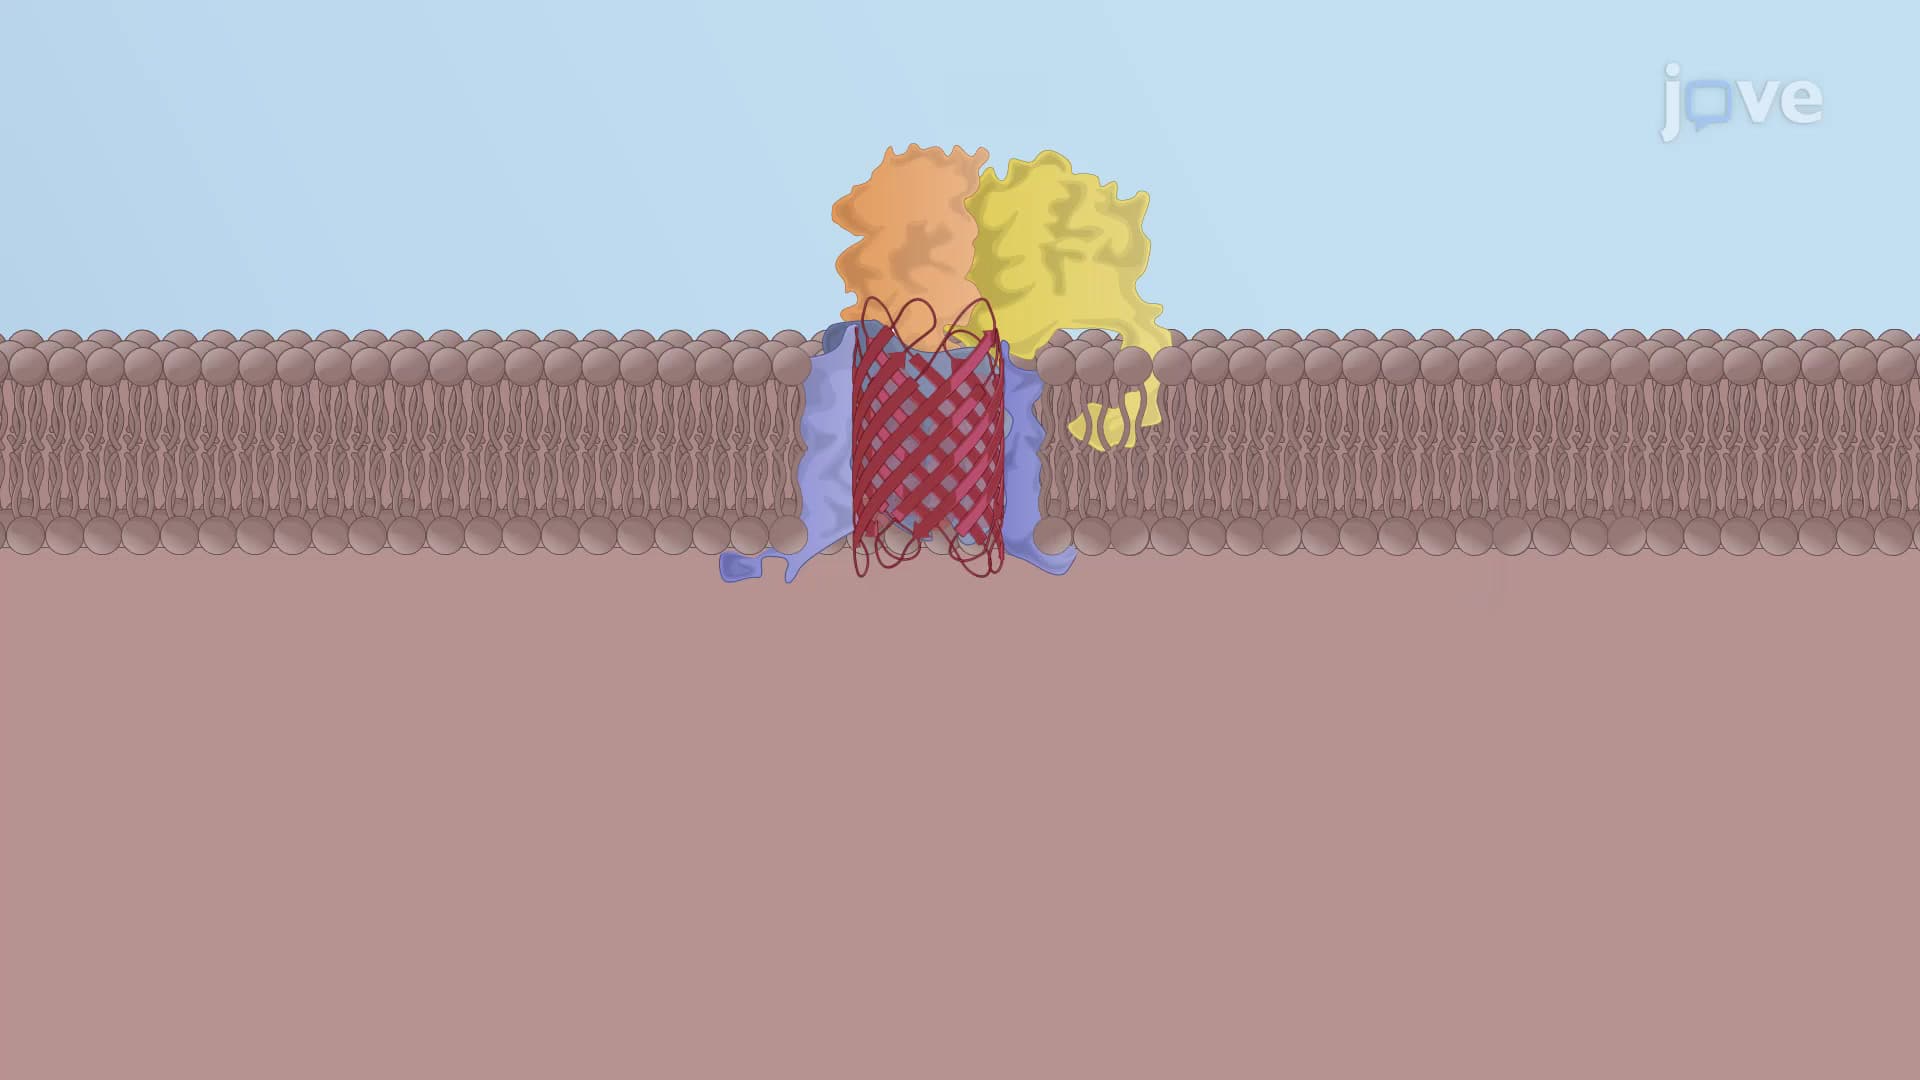
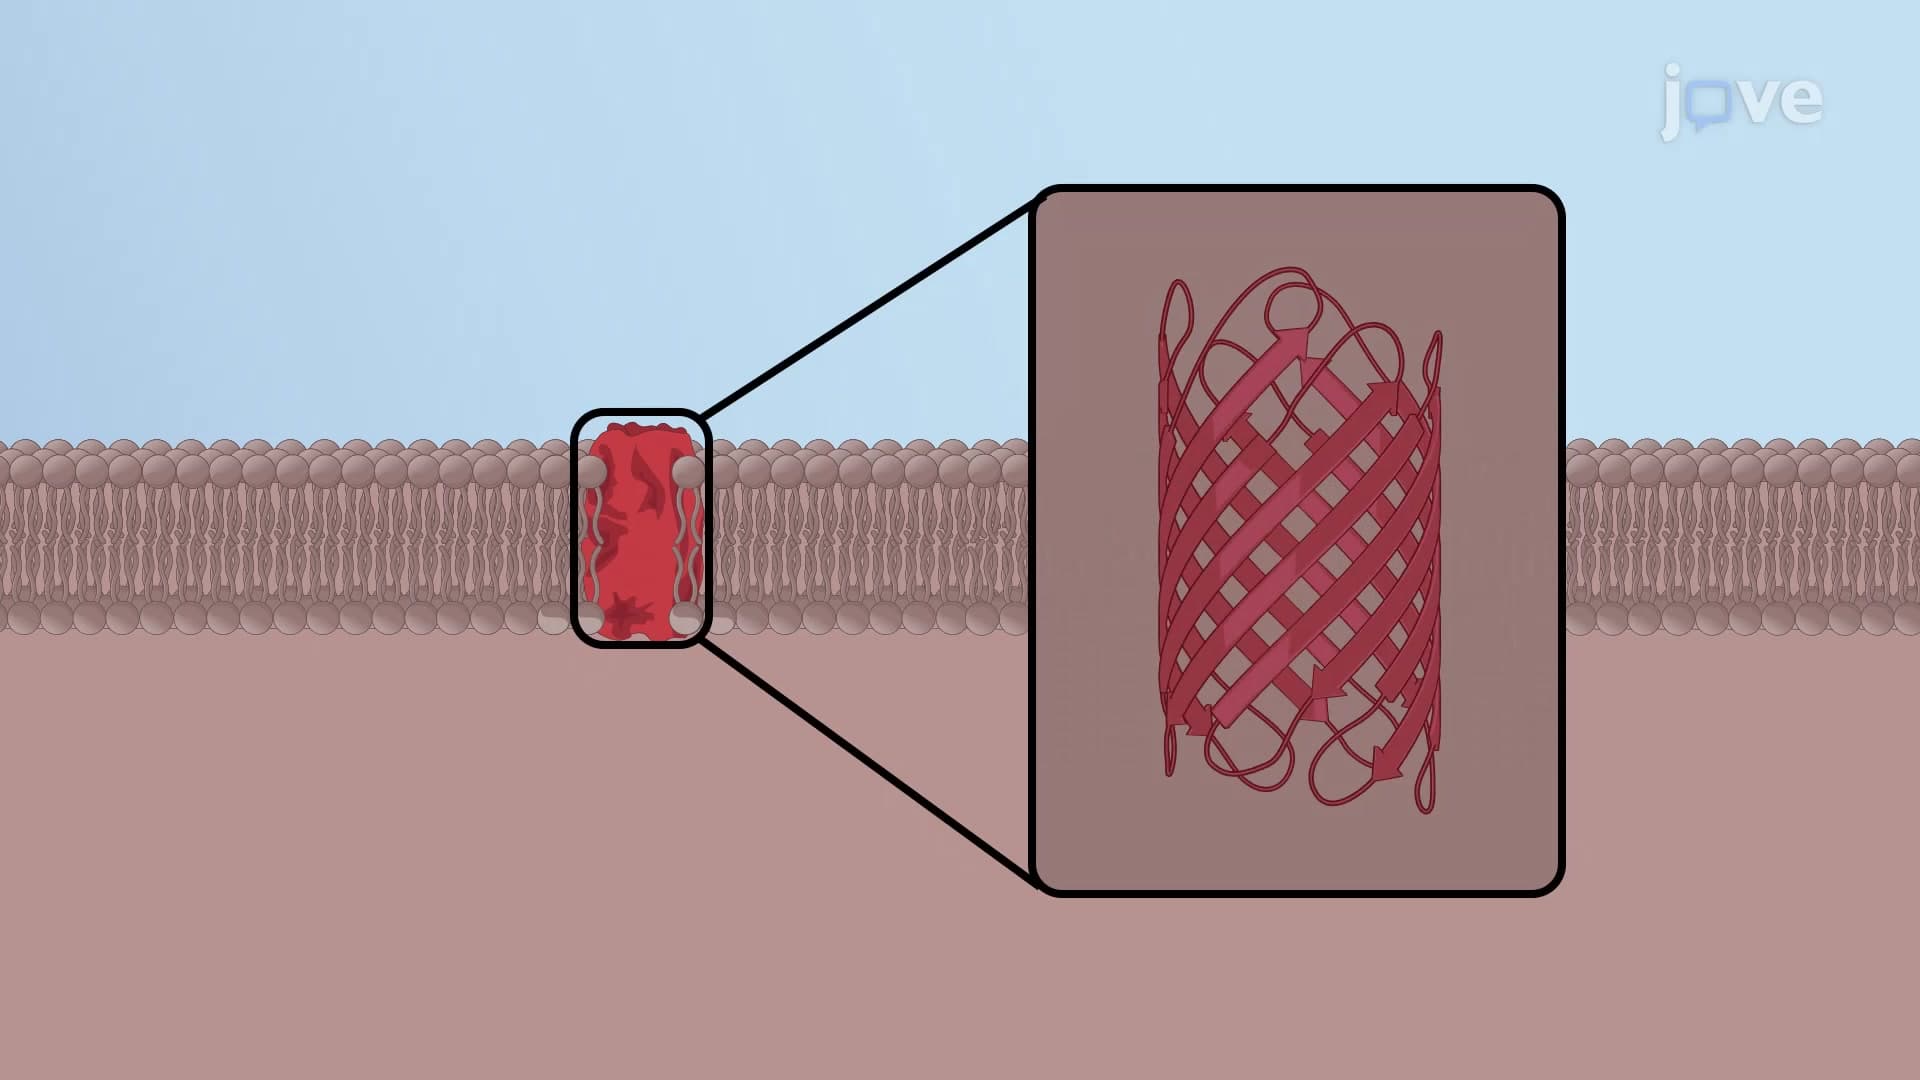
Porins are beta-barrel proteins translocated to the mitochondrial outer membrane through the TOM complex into the intermembrane space. Porin precursors bind TIM chaperones within the intermembrane space and are guided to the Sorting and Assembly Machinery complex or SAM complex on the outer mitochondrial membrane.
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
2.9K
 01:21
Structure of Porins
2.9K
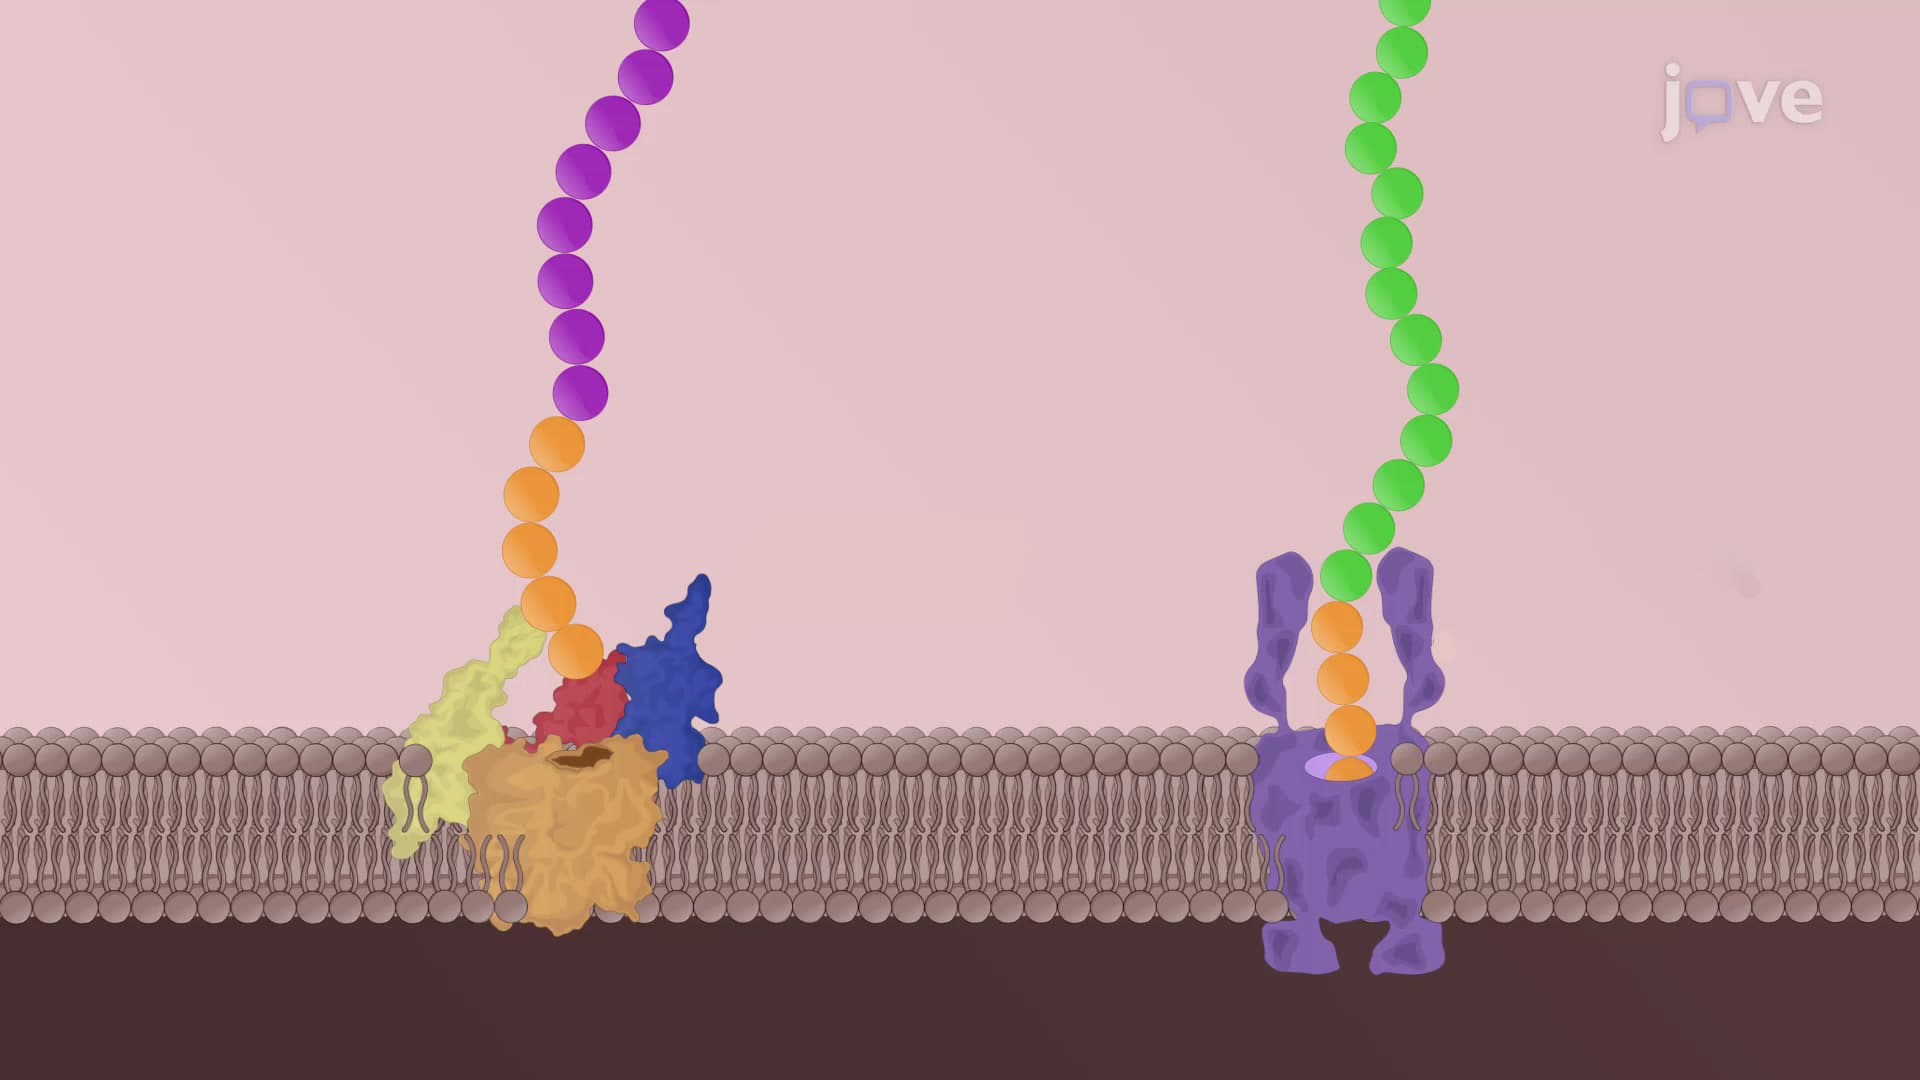
Mitochondria, chloroplasts, and gram-negative bacteria have transmembrane, beta-barrel proteins called porins to mediate the free diffusion of ions and metabolites across the membrane. Mitochondrial porin precursors contain conserved amino acid sequences called beta signals at their C-terminal. Beta signals have a motif of PoXGXXHyXHy (Po-Polar, X-Any amino acid, G-Glycine, Hy-LargeHydrophobic), which are crucial for precursor recognition to initiate precursor assembly. Beta-barrel...
2.9K
 01:34
Protein Transport into the Inner Mitochondrial Membrane
3.7K
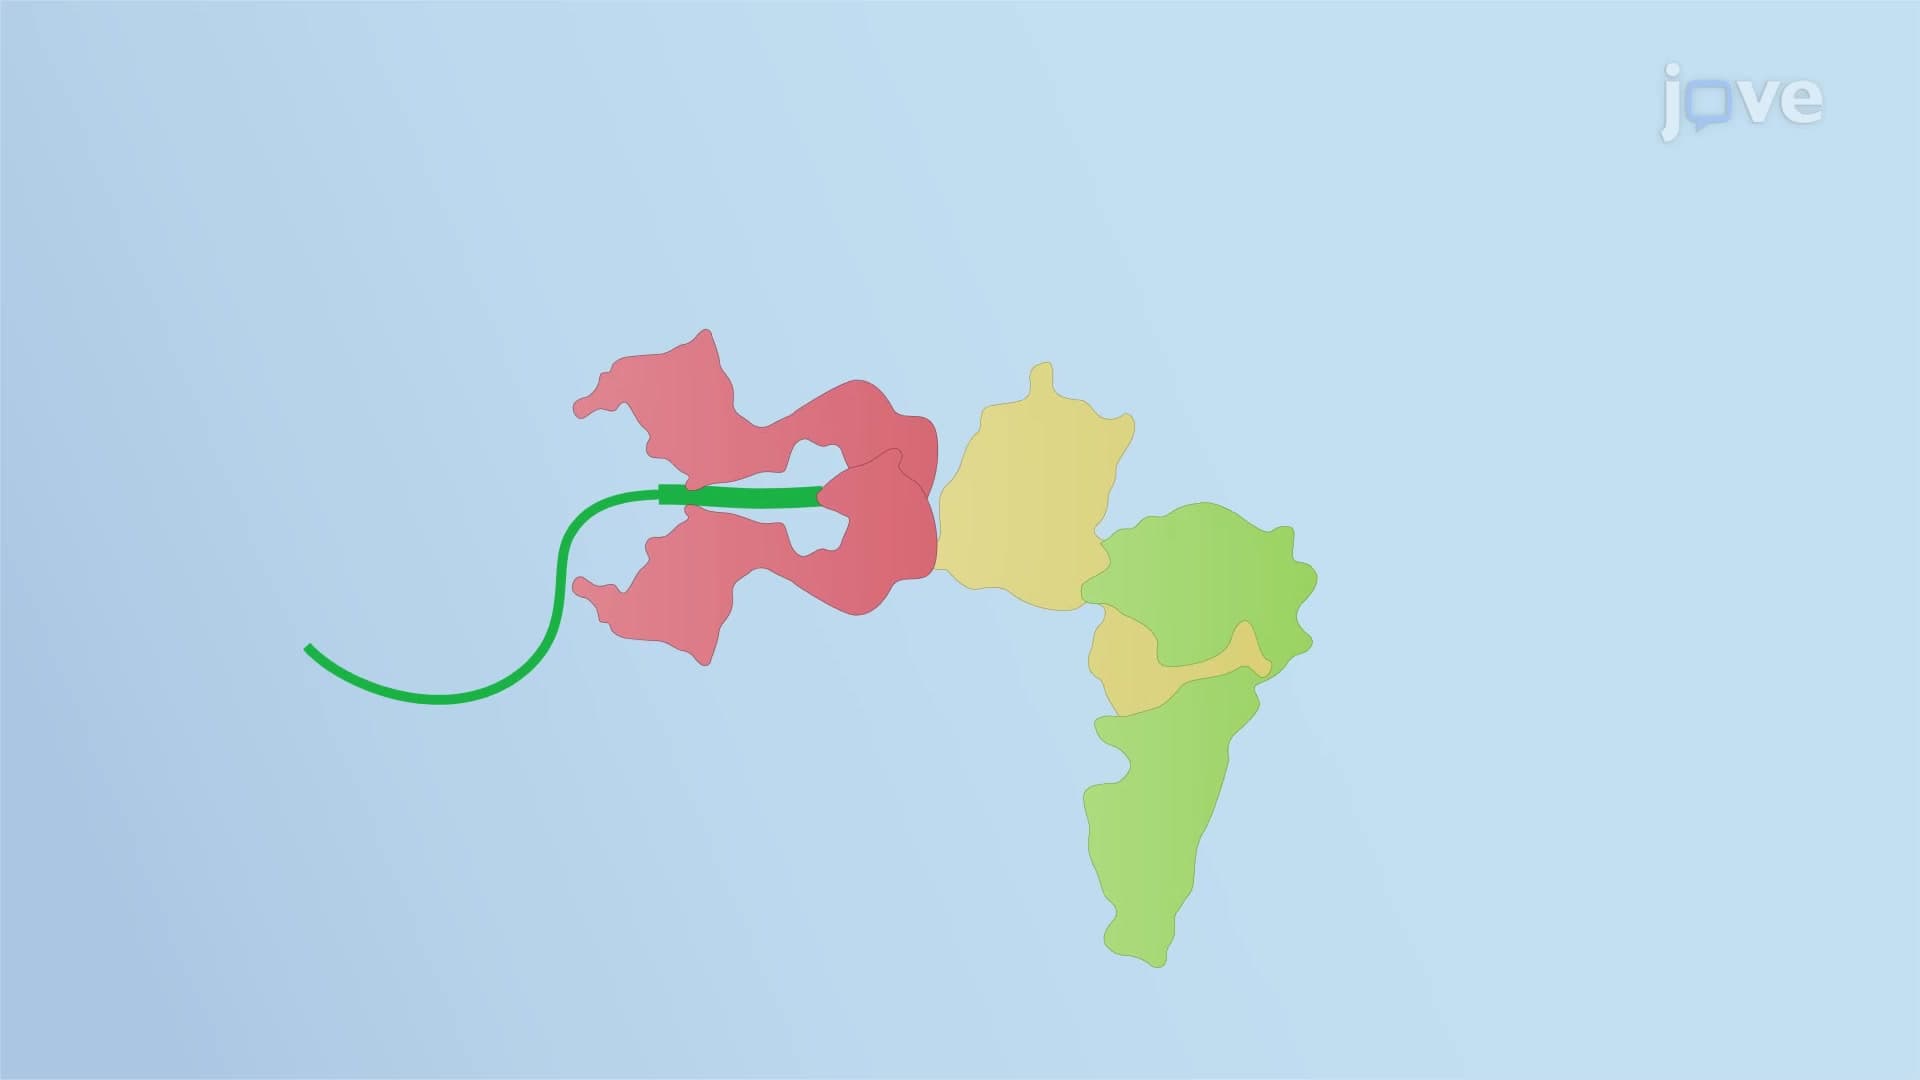
Nuclear encoded mitochondrial precursors are imported to the inner membrane in a multistep process involving two separate translocons, TIM22 and TIM23. TIM23 is a cation-selective pore that remains closed by the N terminal segment of the protein. Negative charges on the TIM23 act as a receptor for the incoming precursor, pulling the positively charged matrix-targeting sequence for peptide insertion and translocation.
Transport of mitochondrial precursors across the TIM23 channel is driven by...
Transport of mitochondrial precursors across the TIM23 channel is driven by...
3.7K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.1K
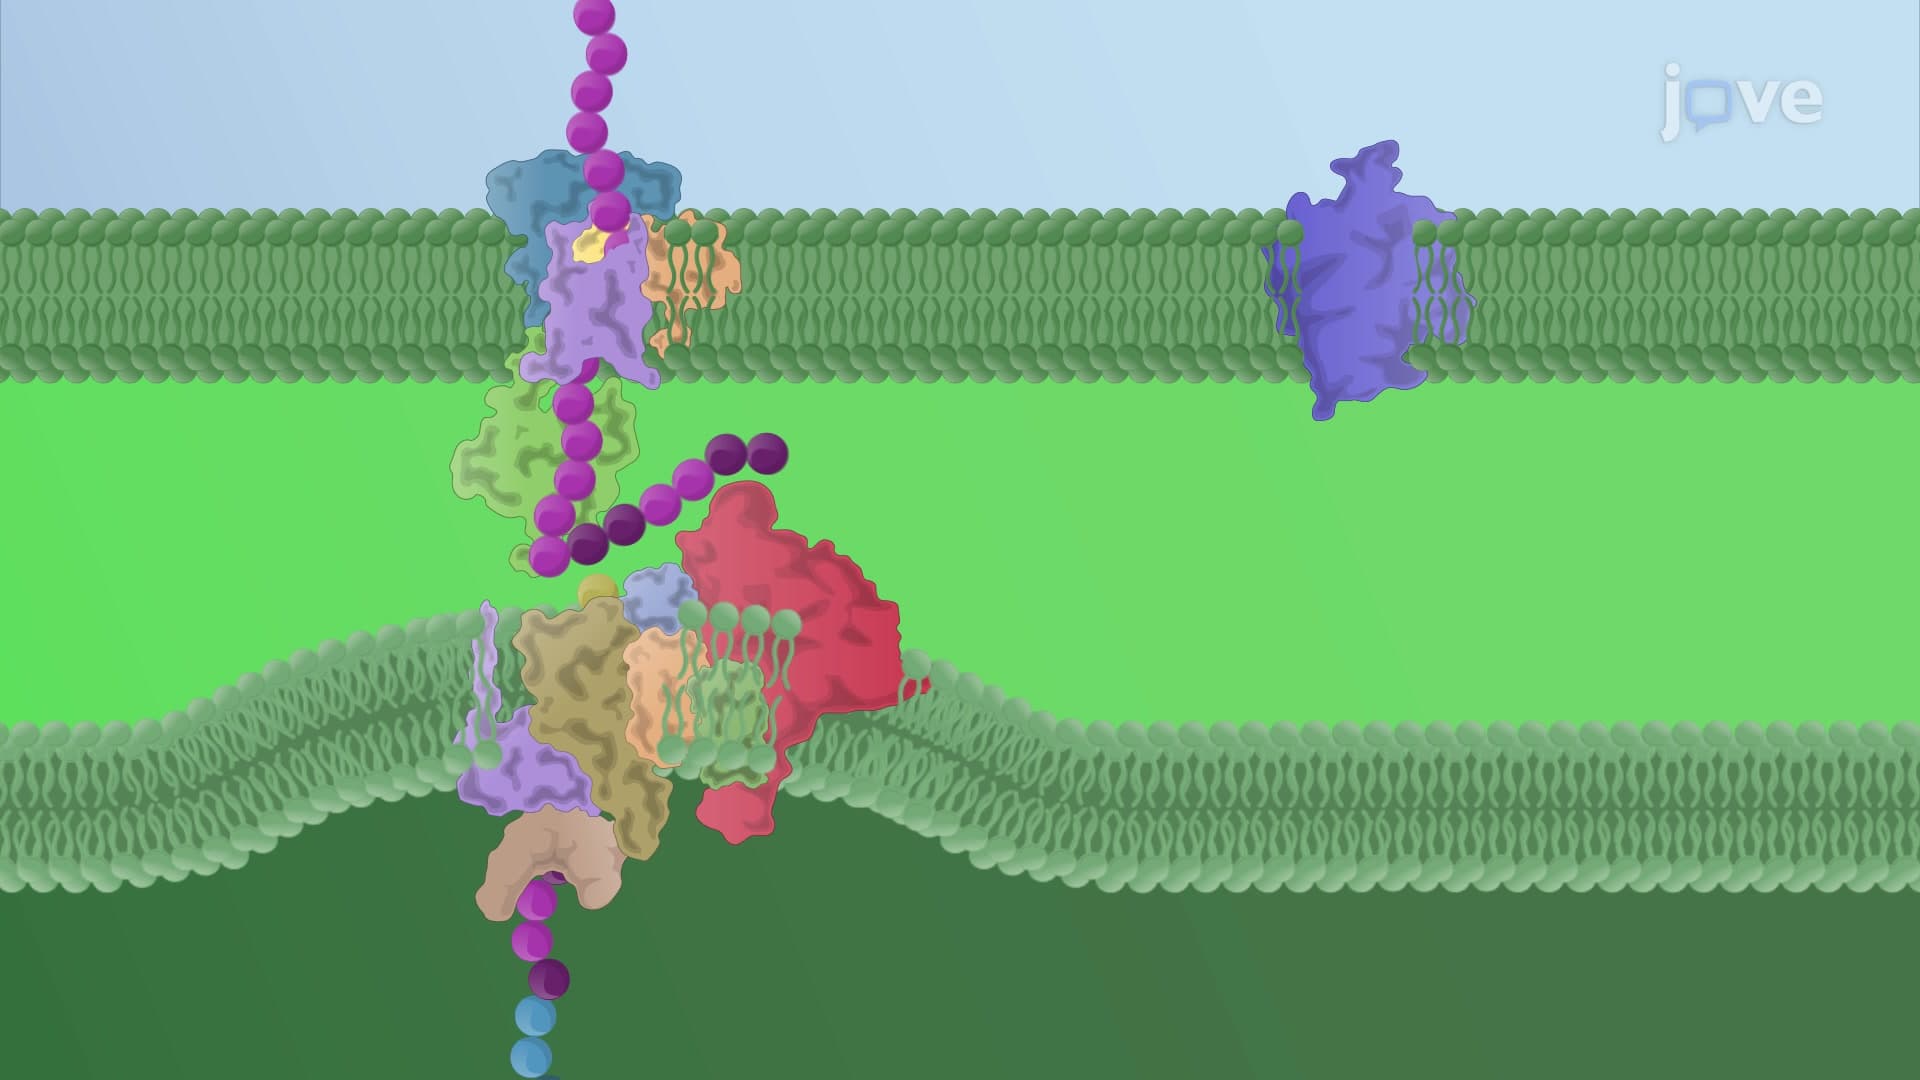
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.1K
 00:59
Mechanisms of Membrane Domain Formation
3.0K
Different physical properties of lipids and proteins allow them to localize and form distinct islands or domains in the membrane. Some membrane domains are formed due to protein-protein interactions, whereas others are formed due to the presence of specific lipids such as sphingolipids and sterols—for example, large proteins, such as bacteriorhodopsin, aggregate and create distinct domains.
Another mechanism for membrane domain formation involves membrane proteins interacting with...
Another mechanism for membrane domain formation involves membrane proteins interacting with...
3.0K
 01:11
Protein Transport to the Outer Chloroplast Membrane
2.0K
Chloroplast outer membrane proteins encoded by the nucleus are synthesized in the cytosol. Soon after synthesis, they bind cytosolic factors such as 14-3-3 protein and the Hsp70 chaperones that keep these precursors in an unfolded state until their translocation.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
2.0K