
加斯德明 D 半氨酸残留物协同控制其棕化介导的膜向和组装
Eleonora Margheritis1, Shirin Kappelhoff1, John Danial2,3,4
1Department of Biology/Chemistry and Center for Cellular Nanoanalytics (CellNanOs), University of Osnabrück, Osnabrück, Germany.
The EMBO journal
|August 14, 2024

概括
气体皮质D (GSDMD) 孔组合涉及囊介导的寡合化和膜插入. 特定的半氨酸 (Cys39,Cys57,Cys192) 对于GSDMD构建块和在热时的功能性孔隙形成至关重要.
科学领域:
- 细胞生物学 细胞生物学
- 分子生物学分子生物学
- 生物化学 生化学
背景情况:
- 加斯德明D (GSDMD) 是热的关键执行者,这是一个被编程的细胞死亡途径.
- GSDMD在血中形成毛孔,导致细胞溶解.
- GSDMD毛孔组合的精确机制以及囊残留物的作用仍然不清楚.
研究的目的:
- 为了阐明Gasdermin D (GSDMD) 孔组合的机制.
- 调查特定的氨酸残留在GSDMD寡合化和膜插入中的作用.
- 了解GSDMD膜准的调节方法.
主要方法:
- 采用了单分子成像技术.
- 进行了氨酸残留物的局部导向突变发生.
- 实验使用人工膜和等离子膜.
主要成果:
- 在膜上,GSDMD预组装成二度和三度构建块.
- 氨酸残留物Cys39,Cys57和Cys192对于GSDMD的寡合化至关重要.
- Cys192的S-palmitoylation和负电荷的脂质控制了GSDMD的膜向.
- 同时的Cys39/57/192突变取消了GSDMD膜插入,而单个或对突变没有.
- Cys192或Cys39/Cys57对可使二聚体/三聚体形成,但所有这些都是高阶寡聚体所需的.
结论:
- GSDMD的寡合化遵循涉及氨酸残留的两步机制.
- Cys192棕化介导的膜结合和Cys39/57/192介导的寡合化在GSDMD孔组合中进行合作.
- 这项研究提供了关键的洞察力,了解了由GSDMD.GSDMD.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.D.
相关概念视频
 01:32
Lipids as Anchors
5.6K
In the plasma membrane, the lipids forming the bilayer can also act as an anchor to tether proteins to the membrane. The three main types of lipid anchors found in eukaryotes are – prenyl groups, fatty acyl groups, and glycosylphosphatidylinositol or GPI groups. Prenyl and fatty acyl groups act as anchors on the cytosolic surface of the membrane, whereas GPI anchors proteins on the extracellular side.
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains...
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains...
5.6K
 01:33
Coat Assembly and GTPases
3.5K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.5K
 01:29
GPI Anchoring of Proteins in the ER Membrane
4.0K
GPI-anchoring is a post-translational, reversible protein modification that is ubiquitous in eukaryotes. Such proteins are primarily present on the exoplasmic leaflet of the plasma membrane.
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
4.0K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.1K
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.1K
 01:26
Protein Modifications in the RER
5.1K
Modification of secretory and transmembrane proteins entering the rough ER begins in the ER lumen. These modifications aid in protein folding and stabilize the acquired tertiary structure. Protein modifications in the rough ER co-occur at different stages of protein folding.
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal...
Broadly, these modifications can be categorized into four main categories — glycosylation, formation of disulfide bonds, assembly of protein subunits, and specific proteolytic cleavages like removal of signal...
5.1K
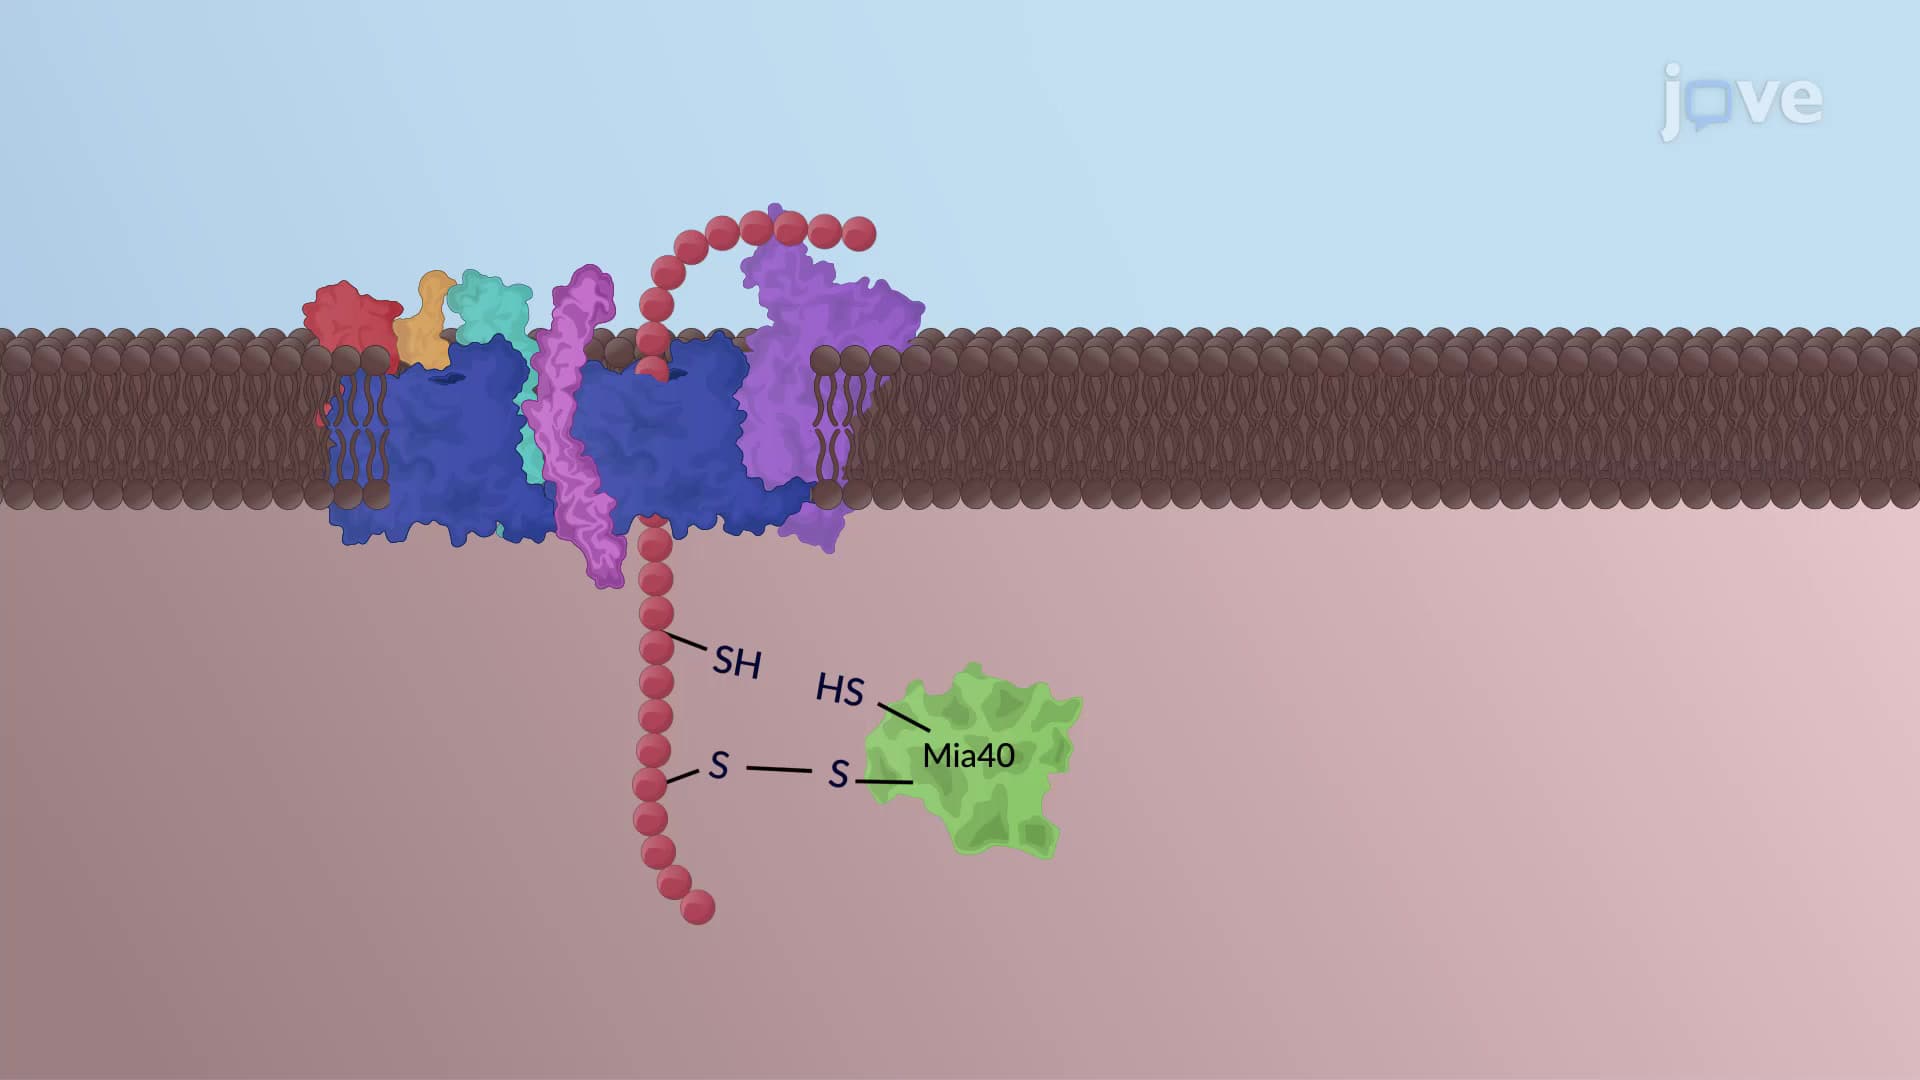 01:19
Translocation of Proteins into the Mitochondria
3.1K
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.1K