相关实验视频
Updated: Jun 9, 2025
09:33

Methods to Classify Cytoplasmic Foci as Mammalian Stress Granules
Published on: May 12, 2017
14.5K
线粒体展开蛋白质反应的激活调节了压力颗粒的动态形成
Marta Lopez-Nieto1,2, Zhaozhi Sun3, Emily Relton1,2
1Faculty of Health and Medical Sciences, School of Biosciences and Medicine, University of Surrey, Guildford GU2 7HX, UK.
Journal of cell science
|October 28, 2024

概括
线粒体展开蛋白反应 (UPRmt) 暂时形成压力颗粒 (SGs),这可能会损害线粒体的功能. 由UPRmt诱导的GADD34限制了SG的形成,有助于细胞存活和线粒体平衡.
科学领域:
- 细胞生物学 细胞生物学
- 线粒体生物学 线粒体生物学
- 压力反应应激反应
背景情况:
- 细胞激活了综合应激反应 (ISR) 和线粒体未折叠蛋白反应 (UPRmt),以适应环境压力.
- ISR触发了转录/翻译变化和压力颗粒 (SG) 的形成,而UPRmt维持了线粒体平衡.
- 通过ISR介导的SG形成与UPRmt之间的相互作用尚未得到充分理解.
研究的目的:
- 调查压力颗粒 (SG) 形成和线粒体展开蛋白质反应 (UPRmt) 之间的交叉.
- 阐明SG动态在细胞适应线粒体压力的作用.
主要方法:
- 在细胞模型中诱导UPRmt.
- 对eIF2α酸化和SG形成动态的分析.
- 在UPRmt期间评估GADD34 (PPP1R15A) 表达.
- 在不同的SG条件下评估线粒体功能和细胞存活率.
主要成果:
- UPRmt诱导导致暂时的eIF2α酸化和SG形成.
- 在晚期UPRmt期间GADD34诱导抑制了进一步的SG组装.
- 缺少SG可以在UPRmt期间增强线粒体功能和细胞存活率.
- 由UPRmt诱导的SG似乎对线粒体平衡有害.
结论:
- 在SG形成和UPRmt路径之间存在一种新的交叉通话.
- UPRmt暂时诱导SGs,这可能会对线粒体功能产生负面影响.
- 通过GADD34介导的SG抑制对于恢复线粒体平衡和在压力下细胞存活至关重要.
相关概念视频
 01:37
The Unfolded Protein Response
4.4K
The ER is the hub of protein synthesis in a cell. It has robust systems to quality control protein folding and also for degradation of terminally misfolded proteins. Under normal conditions, a small proportion of misfolded proteins that cannot be salvaged need to be transported to the cytoplasm by the ER-associated degradation or ERAD pathways. However, if the ERAD cannot handle the misfolded proteins, the cell activates the unfolded protein response or UPR to adjust the protein folding...
4.4K
 01:31
Regulation of the Unfolded Protein Response
2.4K
Inositol-requiring kinase one or IRE1 is the most conserved eukaryotic unfolded protein response (UPR) receptor. It is a type I transmembrane protein kinase receptor with a distinctive site-specific RNase activity. As the binding mechanics of the misfolded proteins with the N-terminal domain of IRE-1 are unclear, three binding models — direct, indirect, and allosteric -- are proposed for receptor activation. Nevertheless, it is known that once a misfolded protein associates with IRE1, it...
2.4K
 01:19
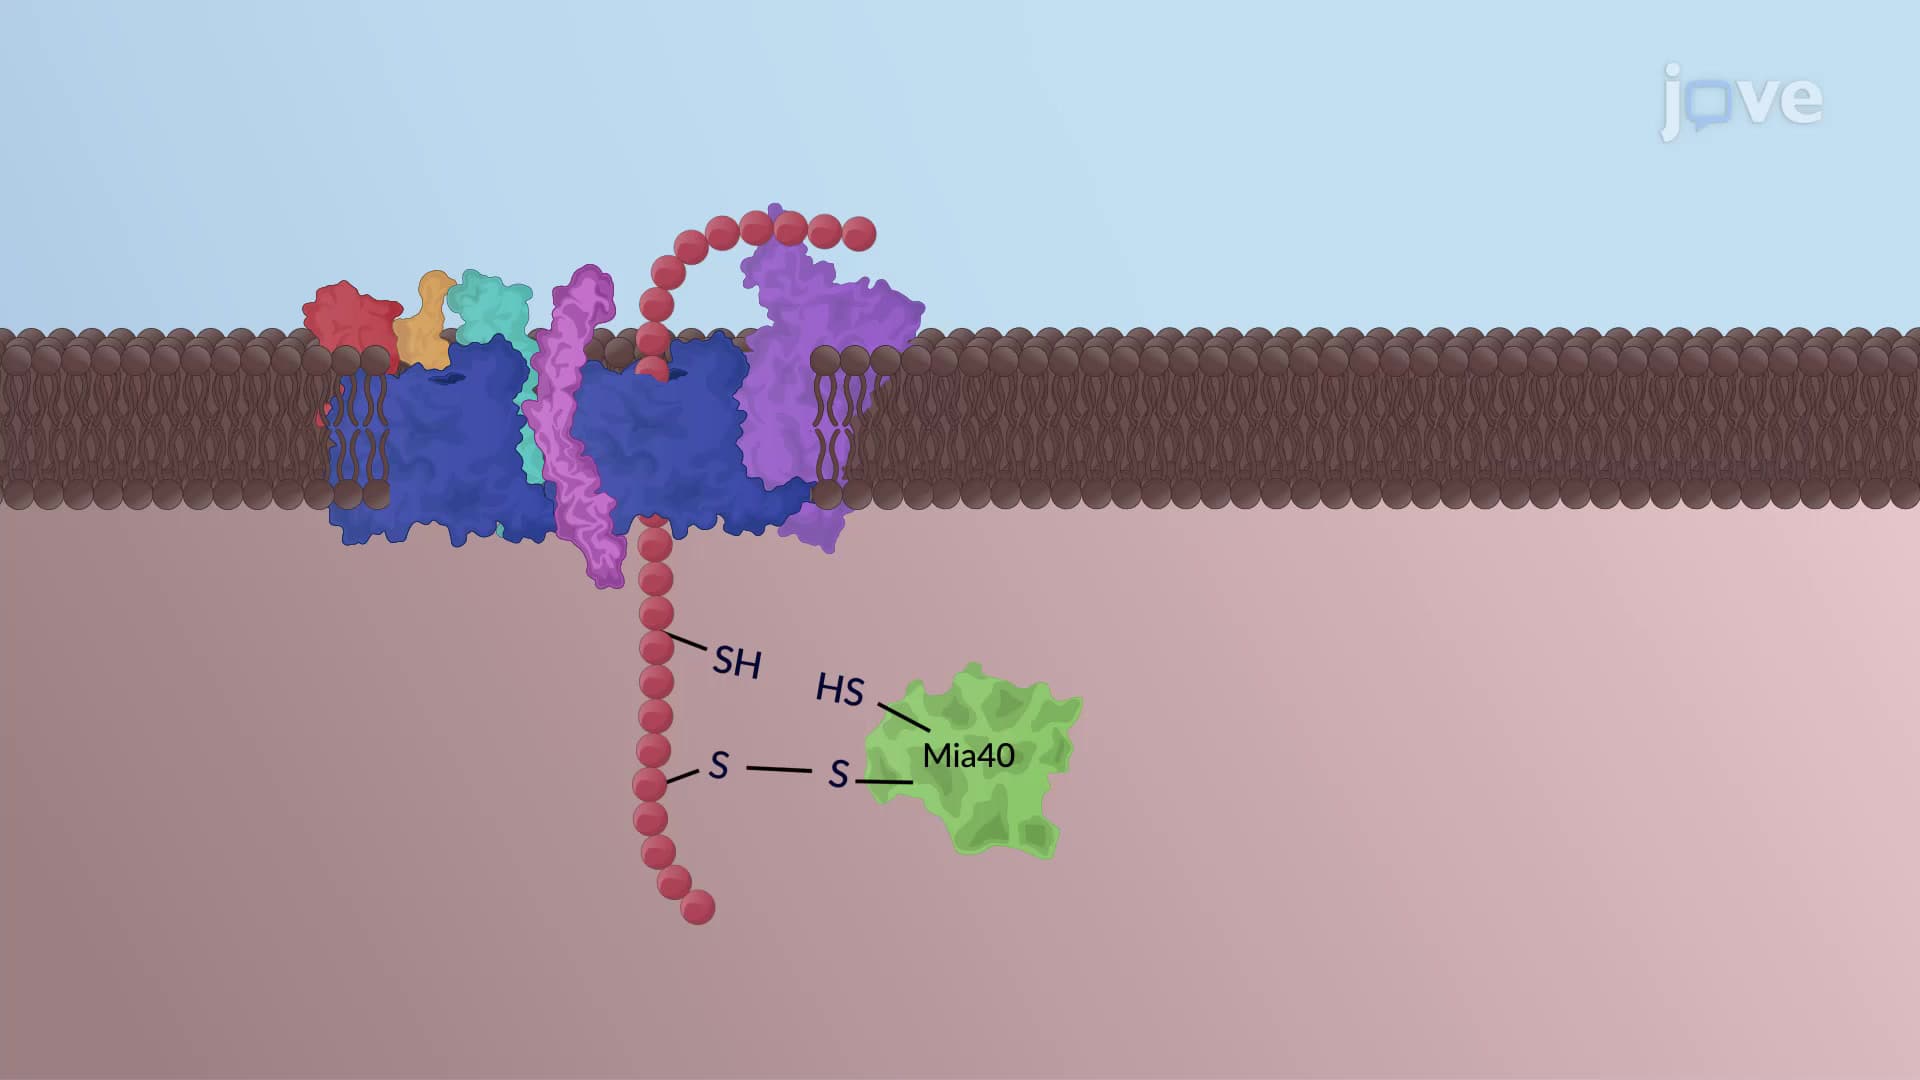
Translocation of Proteins into the Mitochondria
3.0K
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.0K
 01:32
Export of Misfolded Proteins out of the ER
3.5K
After folding, the ER assesses the quality of secretory and membrane proteins. The correctly folded proteins are cleared by the calnexin cycle for transport to their final destination, while misfolded proteins are held back in the ER lumen. The ER chaperones attempt to unfold and refold the misfolded proteins but sometimes fail to achieve the correct native conformation. Such terminally misfolded proteins are then exported to the cytosol by ER-associated degradation or ERAD pathway for...
3.5K
 01:29
Protein Folding Quality Check in the RER
3.7K
ER is the primary site for the maturation and folding of soluble and transmembrane secretory proteins. The calnexin cycle is a specific chaperone system that folds and assesses the confirmation of N-glycosylated proteins before they can exit the ER lumen. The primary players of this quality check pipeline are the lectins, ER-resident chaperones, and a glucosyl transferase enzyme. In case the calnexin system in the lumen fails to salvage a misfolded protein, it is transported to the cytoplasm...
3.7K
 03:00
Molecular Chaperones and Protein Folding
17.8K
The native conformation of a protein is formed by interactions between the side chains of its constituent amino acids. When the amino acids cannot form these interactions, the protein cannot fold by itself and needs chaperones. Notably, chaperones do not relay any additional information required for the folding of polypeptides; the native conformation of a protein is determined solely by its amino acid sequence. Chaperones catalyze protein folding without being a part of the folded protein.
The...
The...
17.8K