
关于激活和调节氨酸-氨酸-NuMA复合物的结构和功能见解
bioRxiv : the preprint server for biology
|December 9, 2024

概括
核转化器 (NuMA) 蛋白激活细胞分裂的dynein电机. 酸化调节了NuMA的作用.
科学领域:
- 细胞生物学 细胞生物学
- 分子生物学分子生物学
- 生物物理学的生物物理.
背景情况:
- 核转化器 (NuMA) 蛋白质对于细胞分裂期间组织微管是至关重要的.
- 努马与dynein电机相互作用,调节螺旋杆形成和皮层力.
研究的目的:
- 阐明NuMA功能的机制和调节.
- 了解NuMA如何与dynein和微管相互作用.
主要方法:
- 在体外溶解试验测定.
- 低温电子显微镜 (cryo-EM) 是一种电子显微镜.
- 活细胞成像 活细胞成像
主要成果:
- 确定了丁氨酸/丁氨酸/NuMA (DDN) 复合物的结构.
- 努马的N端驱动着丁氨酸的运动性;C端抑制了微管的动态.
- 线性酸化激活了NuMA和dynein,形成了类似星体的结构.
结论:
- 努马激活是由酸化和蛋白质相互作用调节的.
- 努马和丁氨酸一起工作,以聚焦微管子的减值末端.
- 努马的局部化进一步由皮质蛋白LGN控制.
相关概念视频
 01:32
Microtubule Associated Motor Proteins
7.7K
Eukaryotic cells have different motor proteins for transporting various cargo within the cell. These motor proteins differ based on the filament they associate with, the direction they move within the cell, and the type of cargo they transport. Motor proteins that associate with microtubules are known as microtubule-associated motor proteins. There are two families of microtubule-associated motor proteins —Kinesins and Dyneins. Both these proteins assist in the transport of cellular...
7.7K
 01:43
The Movement of Organelles and Vesicles
4.4K
In eukaryotic cells, cytoskeletal filaments such as actin, microtubules, and intermediate filaments form a mesh-like cytoskeletal network. These filaments serve as tracks for transporting cellular cargo. Specialized motor proteins use the chemical energy stored in adenosine triphosphate (ATP) for this transport. During interphase, microtubules are polarized, with the plus-end towards the cell periphery and the minus-end towards the cell center. Two microtubule-associated motor proteins,...
4.4K
 01:39
Anaphase A and B
4.0K
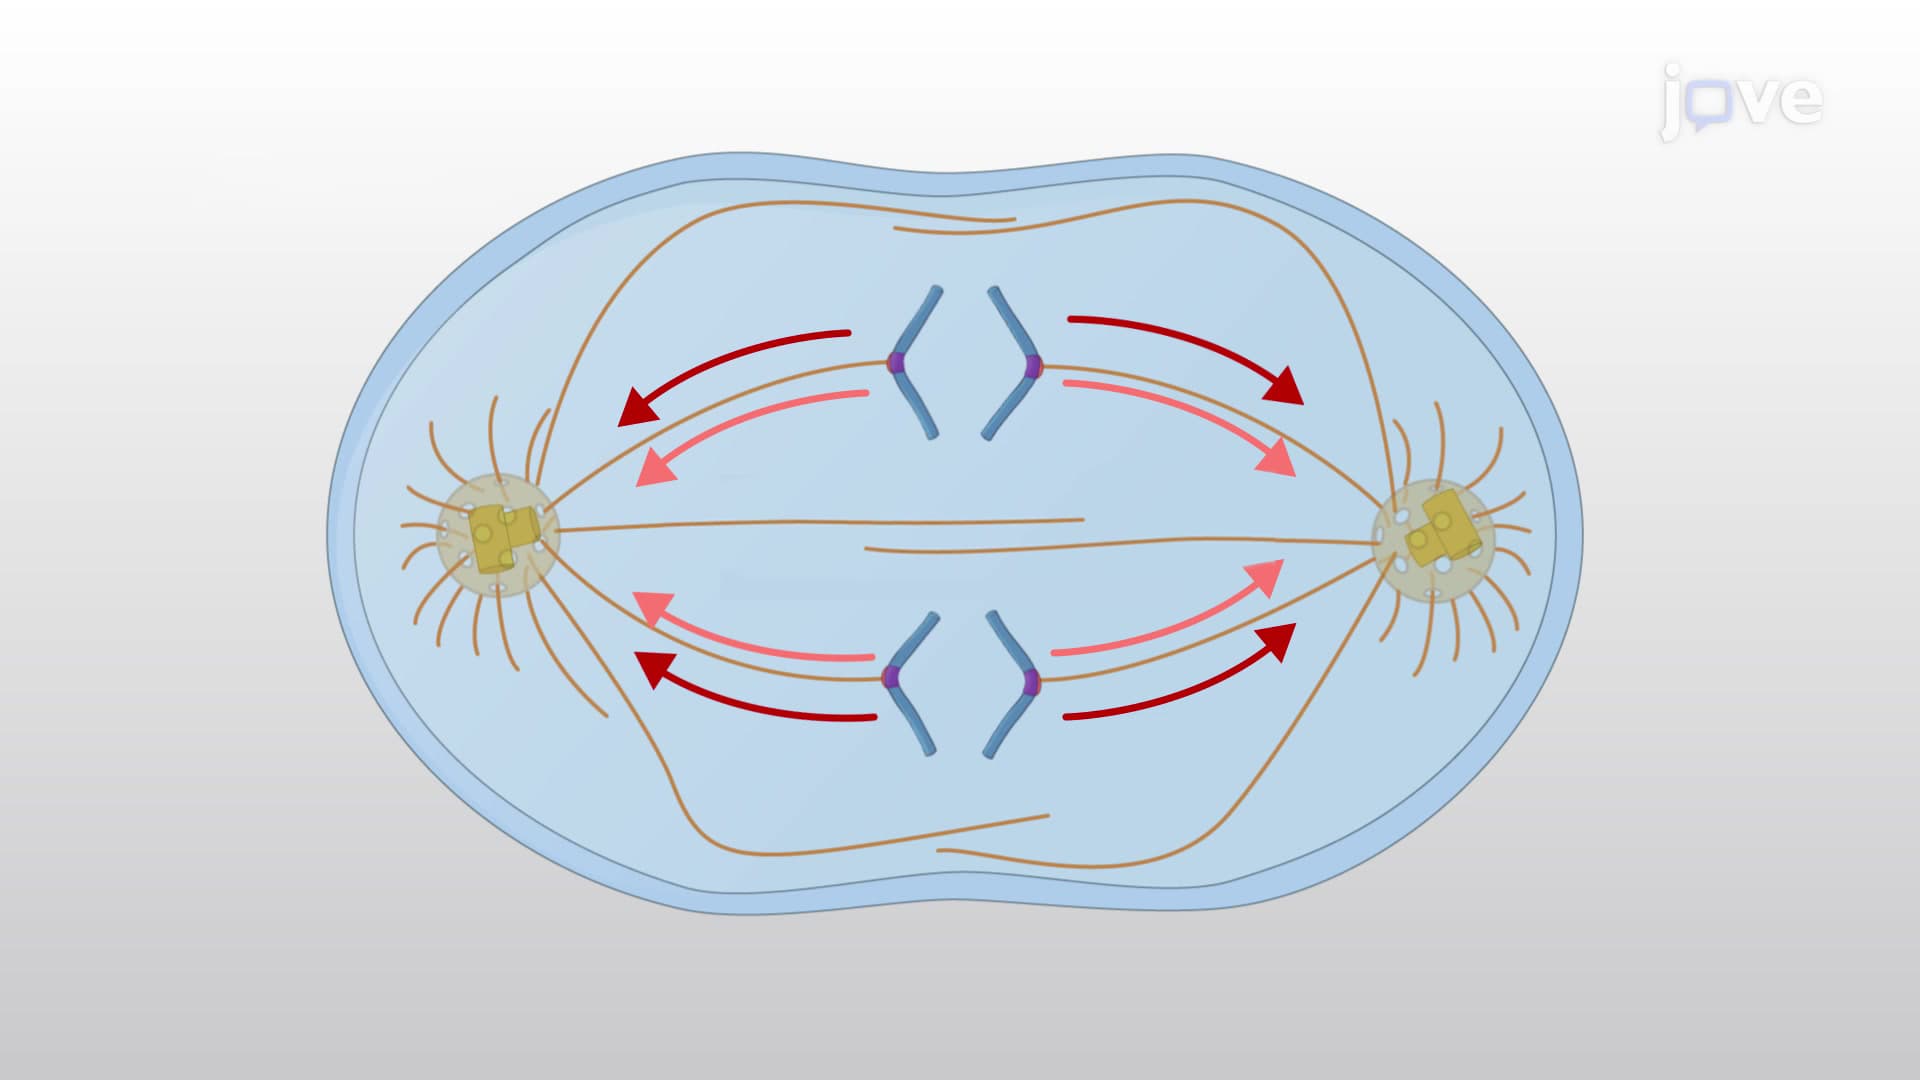
Microtubules form through the end-to-end polymerization of tubulin heterodimers. Kinetochore microtubules originate from the spindle poles, and their plus-ends connect with the kinetochores on sister-chromatids. Ndc80 protein complexes, present on the kinetochore, form low-affinity links with the plus end of these kinetochore microtubules.
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
4.0K
 01:32
Assembly of Complex Microtubule Structures
1.8K
Complex microtubule structures are present in resting cells and in dividing cells. In resting cells, they are responsible for maintaining the cellular architecture, tracks for intracellular transport, positioning of organelles, assembly of cilia and flagella. They mediate the bipolar spindle assembly for chromosomal segregation and positioning of the cell division plate in dividing cells. The formation of microtubule complex structures depends on the cell type, cell stage, and cell function.
1.8K
 01:32
Pinching-off of Coated Vesicles
3.1K
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
3.1K
 01:14
Generation of Straight or Branched Actin Filaments
2.9K
The straight or branched structure formation of actin filaments is controlled by nucleating proteins such as the formins and Arp2/3 complex. Formin-mediated assembly results in straight filaments, whereas Arp2/3 protein complex-mediated assembly results in branched actin filaments.
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
2.9K