
由几种植物Toll/interleukin-1受体含有免疫蛋白诱导的下游信号在升高的温度下是稳定的
Héloïse Demont1, Céline Remblière1, Raphaël Culerrier1
1Laboratoire des Interactions Plantes-Microbes-Environnement (LIPME), Université de Toulouse, INRAE, CNRS, 31326 Castanet-Tolosan, France.
Cell reports
|February 21, 2025

概括
通过核酸结合的氨酸丰富的重复受体 (NLRs) 介导的植物免疫反应在高温下减弱. 这项研究揭示了单独的Toll/interleukin-1受体 (TIR) 域在热应激下保持信号传输,与全长NLR不同.
科学领域:
- 植物生物学 植物生物学
- 分子免疫学分子免疫学
- 植物病原体相互作用
背景情况:
- 植物免疫力,特别是由核酸结合的氨酸丰富重复受体 (NLRs) 介导的反应,在最佳生长温度之外经常被抑制.
- 这种取决于温度的植物免疫反应减弱背后的分子机制尚未完全理解.
- 众所周知,N端的Toll/互白素-1受体 (TIR) 域足以启动免疫信号传递.
研究的目的:
- 研究植物NLR介导免疫的温度依赖调节的分子机制.
- 为了确定单独的Toll/interleukin-1受体 (TIR) 域是否在触发免疫信号时,与全长NLR相比,具有不同的温度敏感性.
- 了解气候变化对植物疾病耐药性的影响.
主要方法:
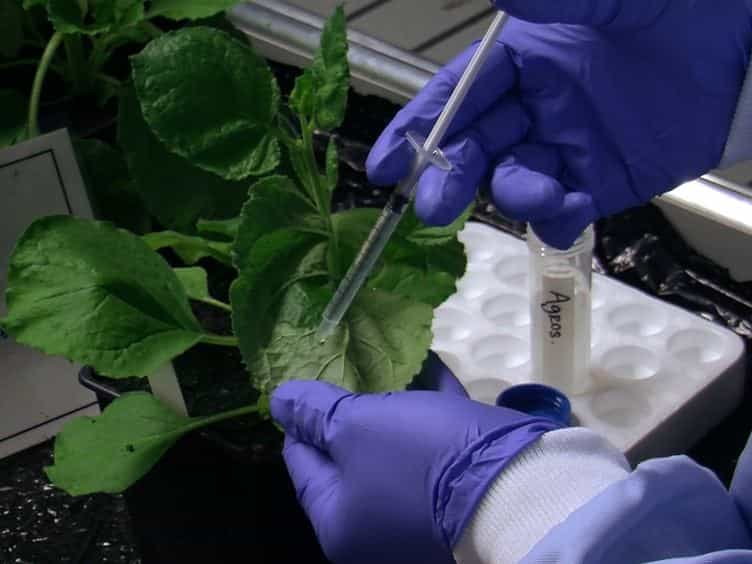
- 条件激活两个具有良好特征的TIR含有NLRs (TNLs) 和它们在Arabidopsis中孤立的TIR域.
- 下游信号通路的分析,包括增强的疾病易感性1 (EDS1) /助手NLRs与RPW8类似的N终端CCR域 (RNL) 要求和酸通路激活.
- 在允许温度和高温 (30°C) 的信号通路维护的比较.
主要成果:
- 在允许的温度下,全长的TNL及其孤立的TIR域触发了相同的信号通路.
- 这种信号通路,当单独由TIR域诱导时,在高温 (30°C) 中保持.
- 然而,在高温下,全长TNL引发的信号无法维持.
结论:
- TIR域具有内在的特性,允许在更高的温度下持续免疫信号,独立于完整的NLR结构.
- 温度显著影响全长NLR的功能,这表明一个关键的监管机制.
- 进一步研究温度对NLRs的影响对于在全球变暖的背景下增强植物抗病能力至关重要.
相关概念视频
 02:45
Responses to Heat and Cold Stress
13.3K
Every organism has an optimum temperature range within which healthy growth and physiological functioning can occur. At the ends of this range, there will be a minimum and maximum temperature that interrupt biological processes.
13.3K
 01:25
Cell Signaling in Plants
5.6K
Plant cells communicate to coordinate their cycle of growth, flowering and fruiting, and activities in roots, shoots, and leaves in response to the changing environmental conditions. Plant signaling is distinct from animal signaling. Plants primarily utilize enzyme-linked receptors, whereas the largest class of cell-surface receptors in animals are G-protein coupled receptors (GPCRs). Unlike animals, receptor tyrosine kinases are rare in plants. Instead, plants have a diverse class of...
5.6K
 01:16
TGF - β Signaling Pathway
7.2K
The TGF-β signaling pathway regulates cell growth, differentiation, adhesion, motility, and development. TGF-β ligands that induce TGF-β signaling are synthesized in their latent form. Several proteases or cell surface receptors such as integrins act upon the latent form, releasing the active ligand. There are three types of mammalian TGF-βs: (TGF-β1, TGF-β2, and TGF-β3) that bind as homodimers or heterodimers to TGF-β receptors. The TGF-β receptors...
7.2K
 01:31
Regulation of the Unfolded Protein Response
2.4K
Inositol-requiring kinase one or IRE1 is the most conserved eukaryotic unfolded protein response (UPR) receptor. It is a type I transmembrane protein kinase receptor with a distinctive site-specific RNase activity. As the binding mechanics of the misfolded proteins with the N-terminal domain of IRE-1 are unclear, three binding models — direct, indirect, and allosteric -- are proposed for receptor activation. Nevertheless, it is known that once a misfolded protein associates with IRE1, it...
2.4K
 02:26
Defenses Against Pathogens and Herbivores
23.0K
Plants present a rich source of nutrients for many organisms, making it a target for herbivores and infectious agents. Plants, though lacking a proper immune system, have developed an array of constitutive and inducible defenses to fend off these attacks.
23.0K
 01:20
The JAK-STAT Signaling Pathway
8.6K
Several cytokine receptors have tightly bound Janus kinase or JAK proteins attached at their cytosolic tail. Small signaling molecules such as cytokines, growth hormones, or prolactins bind to the cytokine receptors and initiate their dimerization. The dimerization brings the cytosolic JAKs together that trans-phosphorylate and activates each other. The activated JAKs now phosphorylate cytosolic tails of the cytokine receptors, which serve as binding sites for adaptor proteins such as SH2...
8.6K