
双链纤维素寡合体强制展开的结构机制
Farkhad Maksudov1, Anna D Protopopova2, Rustem I Litvinov2
1Department of Chemistry, University of Massachusetts, Lowell, Massachusetts 01854, United States.
The journal of physical chemistry. B
|April 14, 2025

概括
研究人员使用AFM,模拟和ML探索了纤维素寡合物纳米机理. 双链纤维素寡合体较少伸展,但更硬,揭示了对血块生物力学的洞察力.
科学领域:
- 生物物理学的生物物理.
- 材料科学 材料科学 材料科学
- 生物化学 生物化学
背景情况:
- 血栓是由纤维素聚合物形成的,这些聚合物在应对机械力时会变形.
- 纤维素纤维的伸展性对凝块功能至关重要,但潜在的机制仍然不清楚.
研究的目的:
- 为了研究双链交联纤维素寡合体 (FO) 的纳米机理.
- 阐明纤维素纤维延长和伸展背后的分子机制.
主要方法:
- 原子力显微镜 (AFM) 用于测量强力延伸形状.
- 计算机模拟以模拟FO解.
- 机器学习 (ML) 用于分析实验和模拟数据.
主要成果:
- 实验数据显示,展开力和延伸的显著分散,归因于卷轴-卷轴波动.
- 模拟显示,FO解涉及合的D:D接口解离,γ结节展开和卷轴转换.
- 与单链寡合体相比,双链FO的延展性降低,但刚性和稳定性增加.
结论:
- 纤维素寡合物纳米机理的特点是,在卷轴内发生联结的展开和重新折叠事件.
- 双链结构有助于纤维素的机械性质,影响凝块的稳定性和伸展性.
- 这些发现提供了关于纤维素动态结构行为的亚分子起源的见解.
相关概念视频
 03:03
Amyloid Fibrils
9.1K
Amyloid fibrils are aggregates of misfolded proteins. Under most circumstances, misfolded proteins are either refolded by chaperone proteins or degraded by the proteasome. However, in the case of a mutation or a disease, these proteins can accumulate to form large clusters and often further assemble to form elongated fibers, called fibrils.
Amyloid deposits were observed as early as 1639 in the liver and the spleen. In 1854, Rudolph Virchow performed iodine staining,...
Amyloid deposits were observed as early as 1639 in the liver and the spleen. In 1854, Rudolph Virchow performed iodine staining,...
9.1K
 01:22
Protein Folding
116.7K
Overview
116.7K
 03:00
Molecular Chaperones and Protein Folding
17.6K
The native conformation of a protein is formed by interactions between the side chains of its constituent amino acids. When the amino acids cannot form these interactions, the protein cannot fold by itself and needs chaperones. Notably, chaperones do not relay any additional information required for the folding of polypeptides; the native conformation of a protein is determined solely by its amino acid sequence. Chaperones catalyze protein folding without being a part of the folded protein.
The...
The...
17.6K
 01:11
Formation of Higher-order Actin Filaments
2.9K
The polymerization of G-actin monomers into filamentous F-actin is a multi-step process. Once the F-actins are formed, they can bundle together in different arrangements to form higher-order networks and regulate cellular functions. Common examples include the formation of lamellipodia and filopodia at the cell's leading edge by actin reorganization in a migrating cell. The microvilli on the brush border epithelial cells are also formed through the F-actin network.
The high-order actin...
The high-order actin...
2.9K
 01:39
Mechanism of Filopodia Formation
2.2K
Filopodia are thin, actin-rich cellular protrusions that play an important role in many fundamental cellular functions. They vary in their occurrence, length, and positioning in different cell types, suggesting their diverse roles.
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
Their main function is to guide migrating cells during normal tissue morphogenesis or cancer metastasis by recognizing and making initial contacts with the extracellular matrix. However, they can also act as stationary cell anchors or help to establish communication...
2.2K
 02:15
Protein and Protein Structure
77.4K
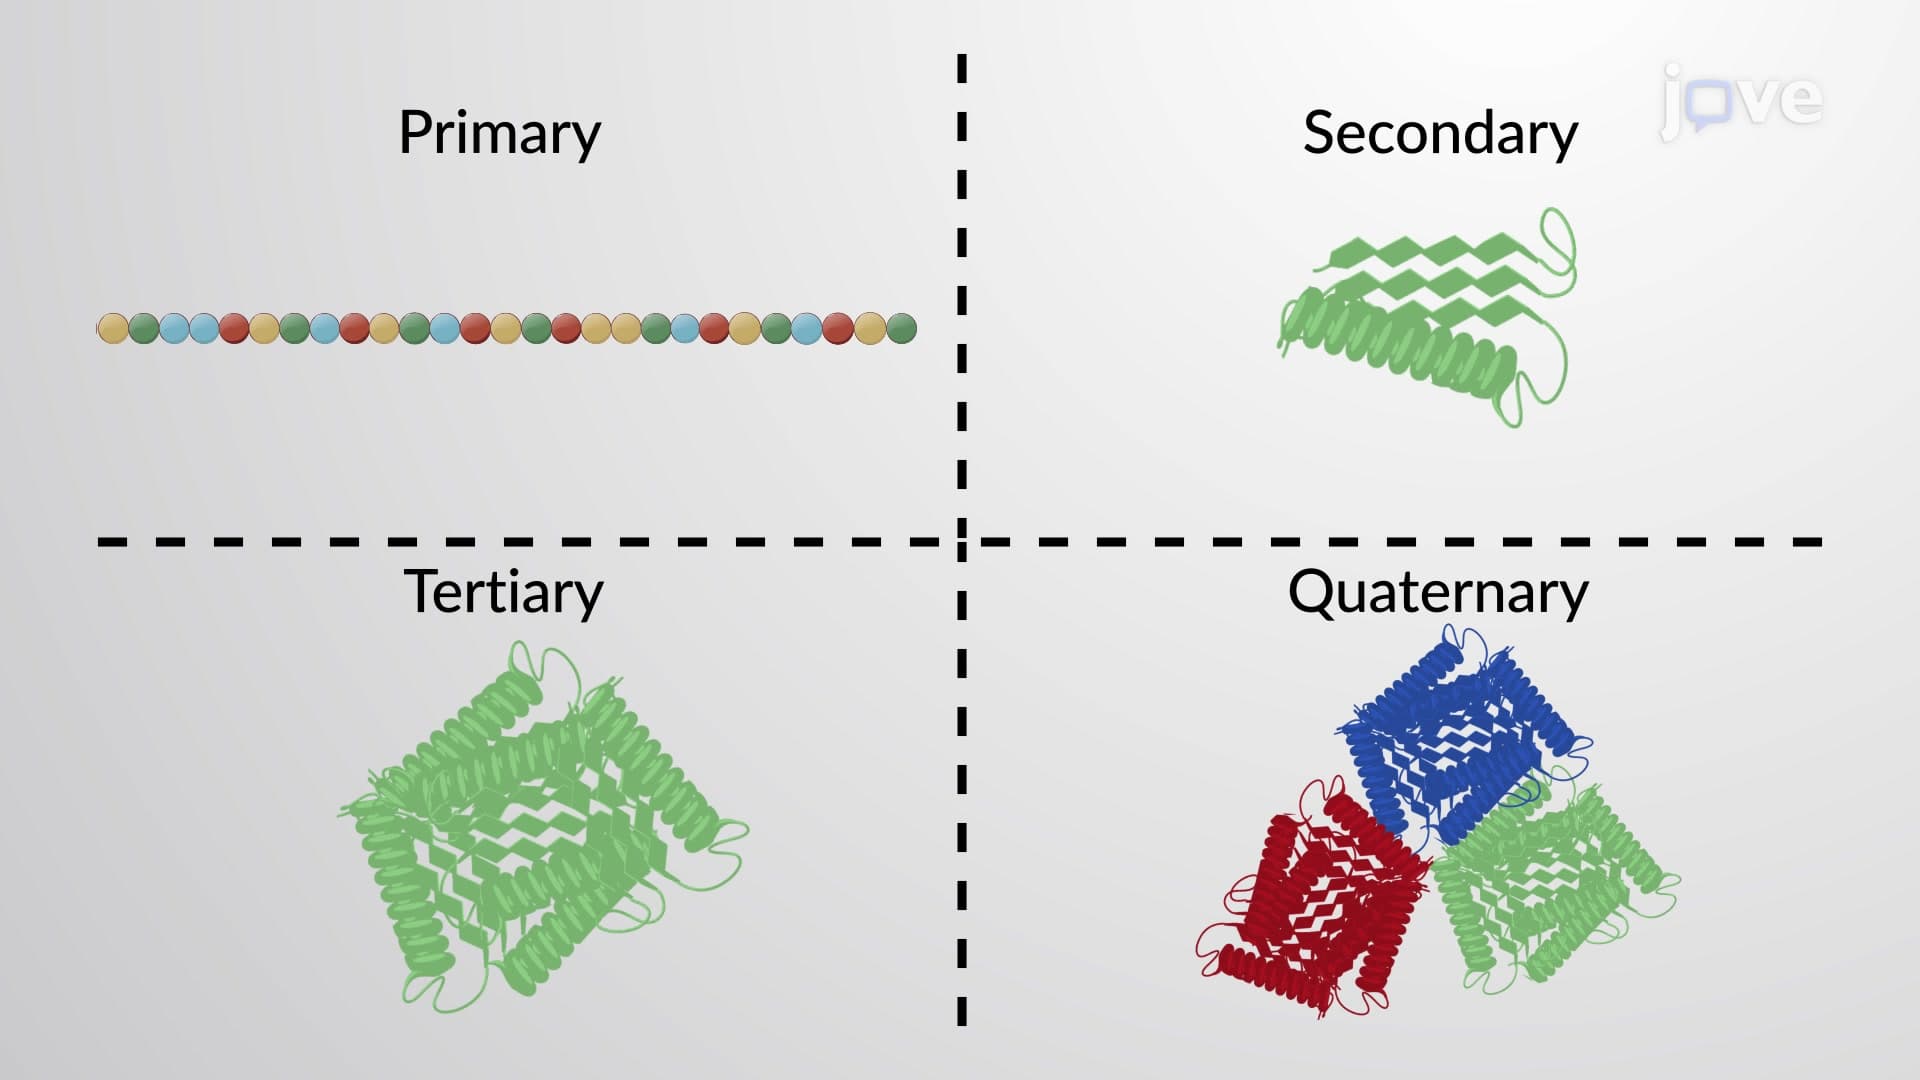
Proteins are one of the most abundant organic molecules in living systems and have the most diverse range of functions of all macromolecules. Proteins may be structural, regulatory, contractile, or protective. They may serve in transport, storage, or membranes; or they may be toxins or enzymes. Their structures, like their functions, vary greatly. They are all, however, amino acid polymers arranged in a linear sequence.
A protein's shape is critical to its function. For example, an enzyme...
A protein's shape is critical to its function. For example, an enzyme...
77.4K